Carbon Degradation-Driven Hypoxia Enhances Phosphorus Mobilization and Nutrient Stoichiometric Imbalance Under Climate Warming and Atmospheric Nutrient Loading in the Ganga River">Carbon Degradation-Driven Hypoxia Enhances Phosphorus Mobilization and Nutrient Stoichiometric Imbalance Under Climate Warming and Atmospheric Nutrient Loading in the Ganga River
Carbon Degradation-Driven Hypoxia Enhances Phosphorus Mobilization and Nutrient Stoichiometric Imbalance Under Climate Warming and Atmospheric Nutrient Loading in the Ganga River
Received: 05 June 2026 Revised: 13 August 2026 Accepted: 15 September 2026 Published: 20 September 2026

© 2026 The authors. This is an open access article under the Creative Commons Attribution 4.0 International License (https://creativecommons.org/licenses/by/4.0/).
1. Introduction
The stoichiometric balance of nitrogen (N) and phosphorus (P) is a fundamental determinant of nutrient limitation, productivity, ecological dynamics, and biogeochemical functioning in freshwater ecosystems [1,2]. Increasing anthropogenic pressures have altered this balance at multiple scales, primarily through enhanced atmospheric nutrient deposition, intensive land use, urban-industrial release, and climate-driven environmental changes [3,4]. Rivers, as integrators of catchment-level processes, are particularly sensitive to such disturbances. A growing body of work suggests that the growth of photosynthetic biota and primary production in freshwaters is frequently limited by the availability of nitrogen and phosphorus [5,6]. This happens due to the altered availability to demand ratios and N:P stoichiometry, as observed in human-impacted rivers and estuaries [7,8]. Such changes are largely driven by anthropogenic nutrient enrichment and hydrological modifications.
In addition to external nutrient enrichment, riverine N:P stoichiometry is strongly influenced by internal biogeochemical processes, including intensive denitrification, sediment-phosphorus release, and coupled redox reactions occurring within sediments, and at the sediment-water interface [9,10]. In freshwater ecosystems, redox-dependent P release and retention [11], together with the intensity of denitrification [12], can significantly affect the absolute and relative availability of P and N. Sediments can therefore act as both sinks and sources of nutrients, and their nutrient stoichiometry reflects the combined influence of long-term external loading and in-situ biogeochemical processes. Variations in the N:P ratios at the sediment-water interface (SWI) subsequently affect nutrient availability and dissolved oxygen (DO) concentration in the overlying water column [13].
Reduced DO conditions, including hypoxia, in rivers are often linked to excessive nutrient loading, which promotes eutrophication and microbial oxygen consumption [14]. Climate warming and carbon flushing from external sources drive further hypoxia by accelerating the biodegradation of recalcitrant organic carbon, thereby intensifying oxygen consumption [15], alongside disruptions to sediment redox conditions. This oxygen depletion facilitates the reductive dissolution of iron-bound phosphorus in sediments, leading to internal P loading and disruption of N:P stoichiometry [16,17]. Such a stoichiometric imbalance favors phosphorus-tolerant species over nitrogen-dependent ones, ultimately altering the community structure and ecosystem functioning [18]. Further, loss of dissolved oxygen, coupled with nutrient imbalances, is a major driver of ecological degradation, often resulting in the decline of sensitive taxa and proliferation of opportunistic or bloom-forming organisms [19,20].
Despite growing understanding of these biogeochemical shifts, the synergistic effects of atmospheric deposition, dissolved oxygen, and climate warming on riverine stoichiometry and associated shifts remain insufficiently understood. This study aims to address this knowledge gap by investigating how atmospheric deposition, coupled with point and non-point sources, in-stream redox conditions, and microbial processes, govern nutrient stoichiometric variability and microbial functioning in the Ganga River. Understanding these linkages, especially under a changing climate scenario, is crucial for predicting ecological responses to global change and improving the effectiveness of nutrient management strategies in large tropical river basins. By integrating field observations and controlled incubation studies, this research provides a more holistic understanding of the interactions among dissolved oxygen dynamics, nutrient cycling, and sediment biogeochemical processes in river ecosystems under anthropogenic stressors and changing climatic conditions.
2. Materials and Methods
2.1. Study Area
The Ganga River Basin represents a diverse landscape ranging from the Himalayan highlands to highly fertile agricultural plains, constituting more than 73% of the total area, supporting over 43% of India’s population. The basin experiences significant anthropogenic pressures from urbanization, agricultural runoff, industrial discharges, groundwater extraction, and hydrological regulation. The climate of the region is tropical monsoonal, characterized by hot summers from April to June, a humid rainy season from July to September, and cooler winter conditions from November to February, with March and October serving as transitional periods. Climatic condition in Tarai region is sub-tropical. Approximately 90% of the annual precipitation (870–1130 mm) occurs during the monsoon season.
During the study period, relative humidity ranged from 27 to 83% during summer and from 58 to 99% during the monsoon season, while daytime summer temperature reached up to 46 °C. The present study was conducted along a 518 km long middle stretch of the Ganga River, between Kanpur (26.51° N; 80.32° E) and Varanasi (25.33° N; 83.04° E) (Figure 1). This river segment experiences substantial environmental stress due to combined urban, industrial, and agricultural inputs, alongside climate warming, making it an important region for investigating changes in nutrient dynamics, pollution impacts, and biogeochemical processes. Flow (water discharge) of the river is highly variable, with sites subject to damming, water extraction, etc. During summer (lean flow months), the average water discharge of the river at Varanasi ranges from 1000 to 3000 m3·s−1.
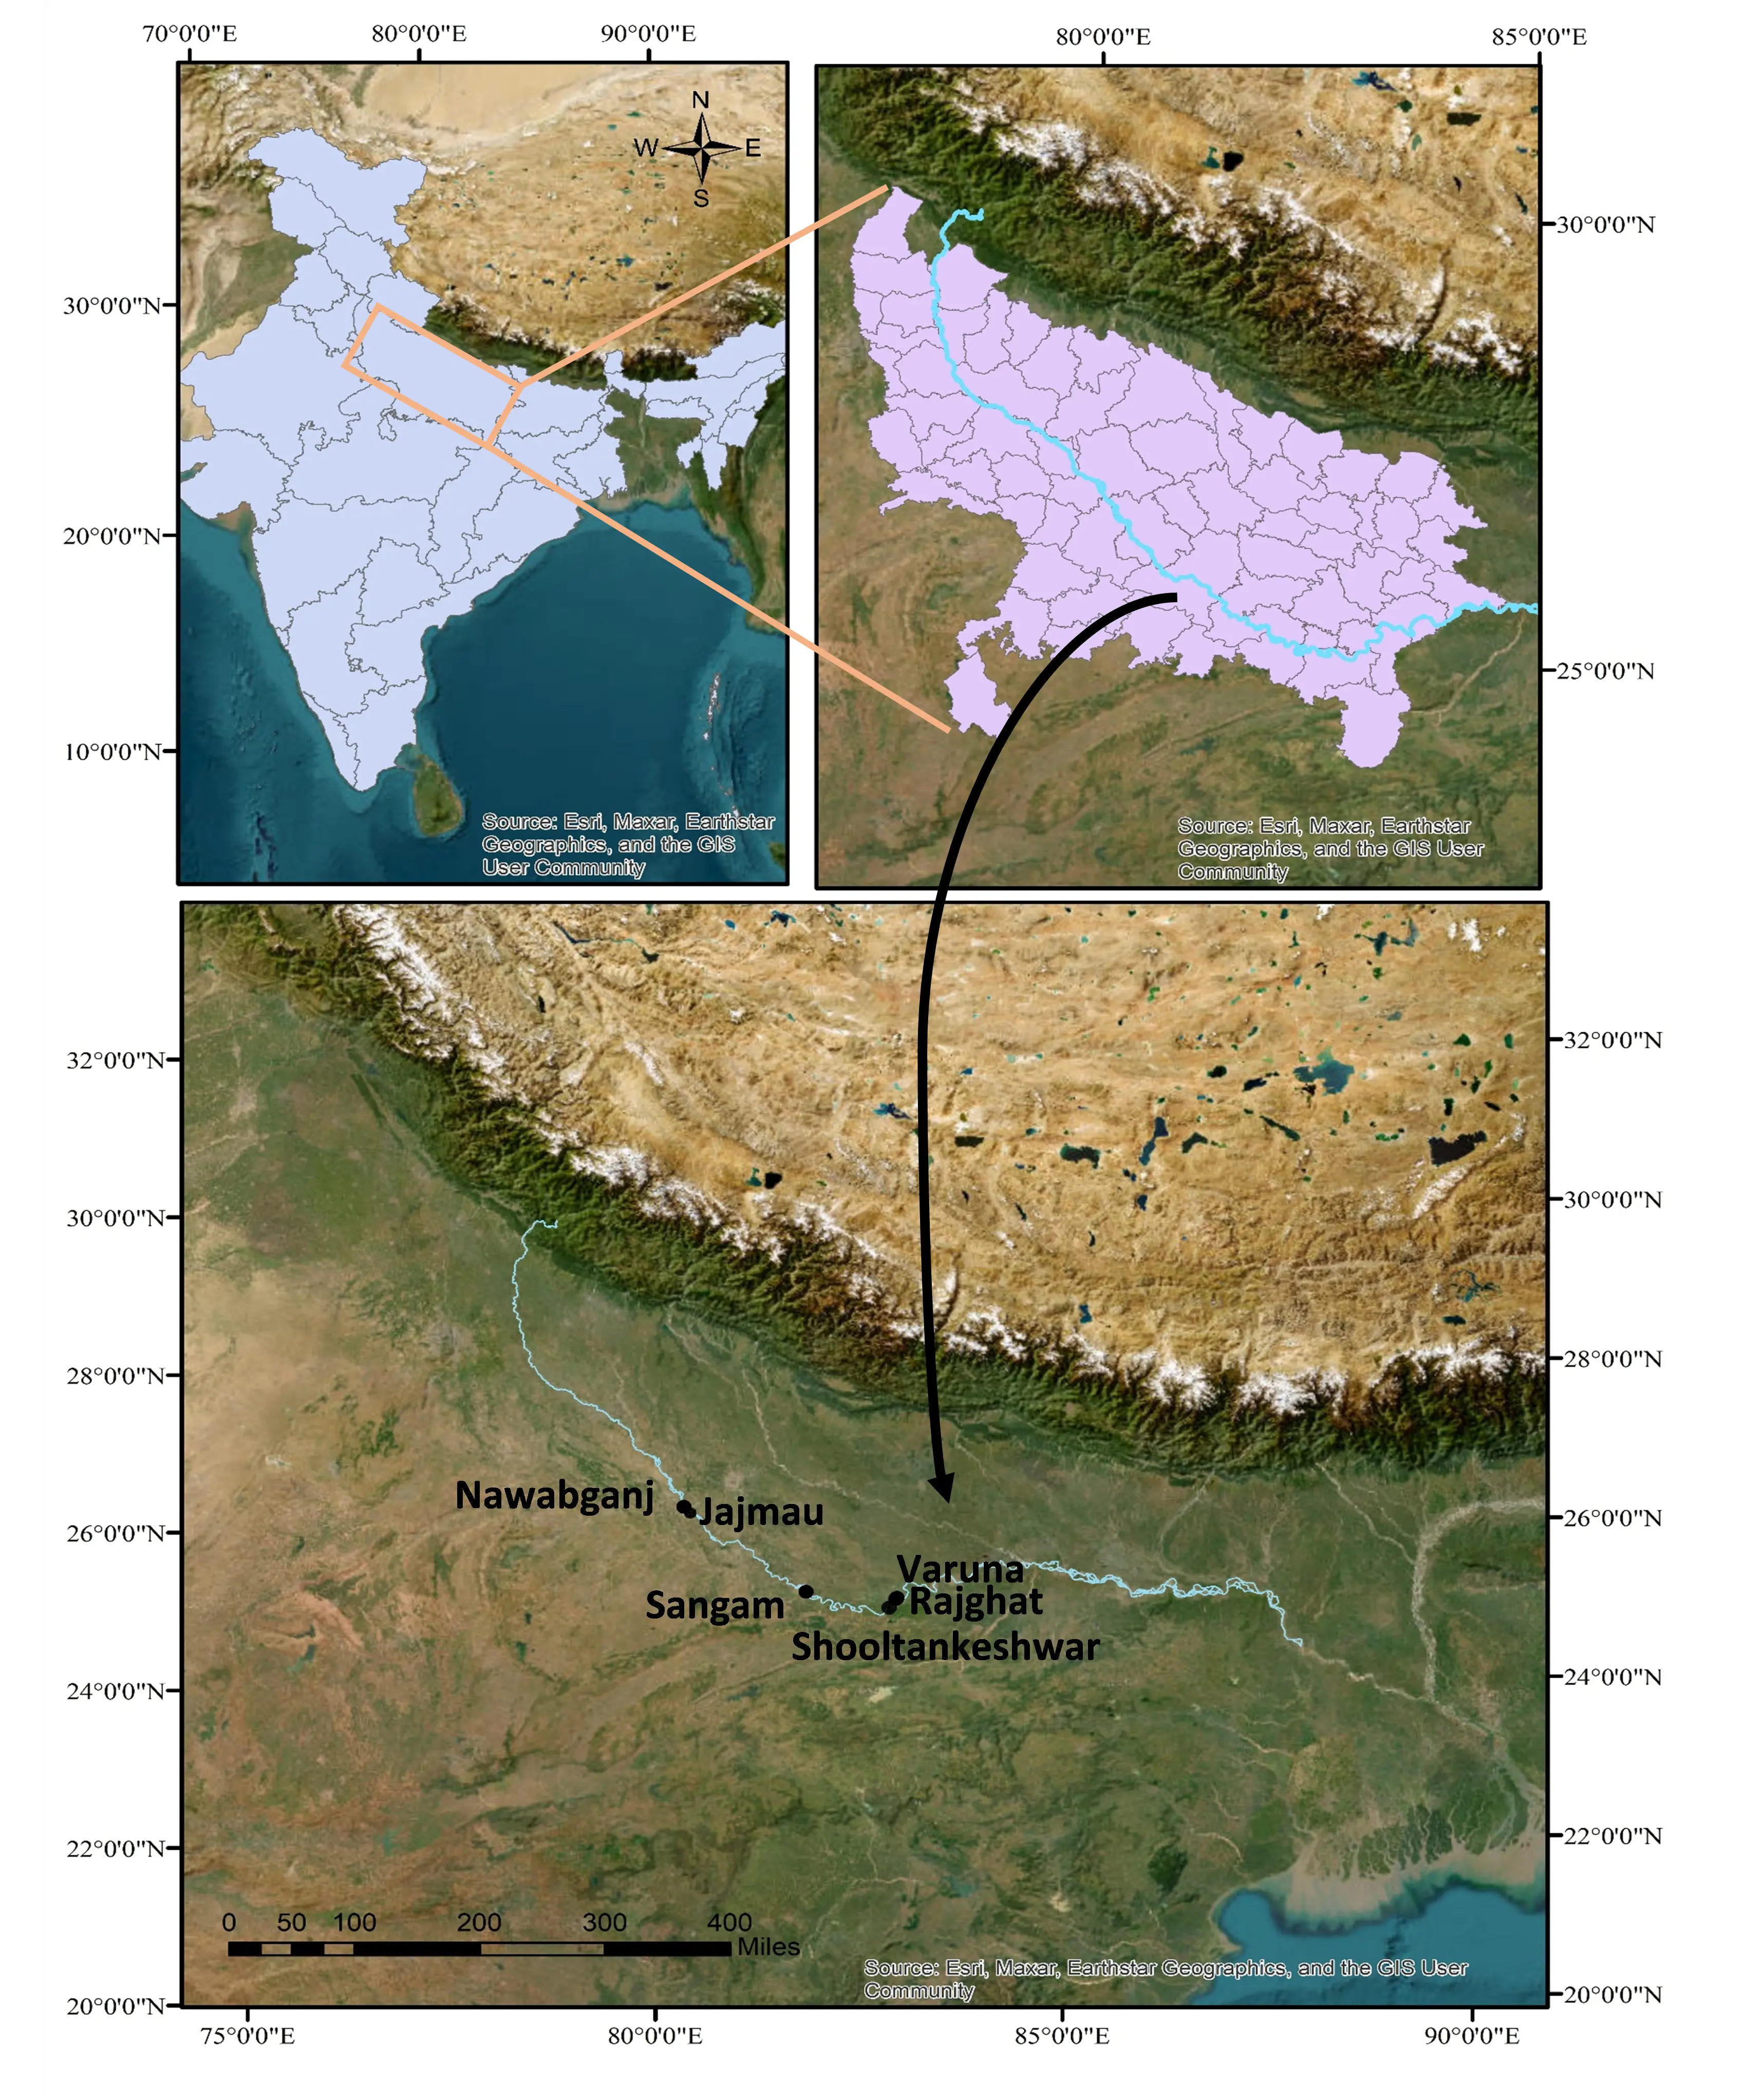
Figure 1. Map presenting the study sites: Nwabganj = Nwbj; Jajmau = Jjmu; Sangam = Sngm; Shoolta1nkeshwar = Shlktr; Rajghat = Rjht; Varuna = Vrna.
2.2. Experimental Protocol
In-situ and incubation experiments were conducted across spatially distinct locations, representing varying degrees of anthropogenic influences and environmental conditions along the middle stretch of the Ganga River. Sampling stations were selected to capture major gradients in pollution load, urban-industrial discharge, tributary influence, and relatively less-disturbed river conditions. Six sampling stations were considered along the study segment: Nawabganj (Nwbj), Jajmau (Jjmu), Sangam (Sngm), Shooltankeshwar (Shlktr), Rajghat (Rjht), and Varuna River confluence (Vrna). Three sub-sites were selected at each station for sample collection to account for local spatial variability. Nawabganj (Nwbj), situated upstream to Kanpur, is a relatively less polluted site, whereas Jajmau (Jjmu), located in Kanpur, represents a major leather industrial cluster and receives substantial inputs of tannery effluents, urban sewage, and other oxygen-demanding substances (ODS) [21]. Sangam (Sngm), situated near Prayagraj, represents the confluence of the River Yamuna and the Ganga, resulting in intense mixing of water, sediments, nutrients, and carbon. Shooltankeshwar (Shlktr), located upstream of Varanasi, experiences comparatively lower anthropogenic disturbance and pollution load. Rajghat (Rjht), situated downstream of Varanasi city, is strongly influenced by urban sewage discharge and industrial effluents. The Varuna (Vrna) River is among the most polluted tributaries of the Ganga, and contributes substantial loads of sewage and industrial waste to the main channel [22]. The Shlktr, a relatively less-disturbed sub-catchment, represents a reference site for comparison of changes observed at more impacted study sites along the study stretch.
2.3. Sample Collection
Water and sediment samples were collected twice a year during the summer months (April and May) for four consecutive years (2021–2024). Samples of water and sediment were collected in triplicate from three sub-sites of each station (n = 18 for each year) from a 25 m reach of the river. Sediment samples (depth: 0–10 cm) were collected using stainless steel corers. Water samples were collected from the sediment-water interface (1.5 to 6.0 m water column depth) using water-depth samplers. Immediately after collection, the samples were placed in the ice boxes and transferred to the laboratory for further analysis. Sediment samples were segregated into two parts: one part was kept intact for measuring sediment-P release, while the other part was kept at room temperature for 3–4 days for air drying. The air-dried samples were then grounded and sieved (2-mm mesh) for further analysis.
2.4. Measurements of Biogeochemical Variables
For the measurement of dissolved oxygen at the sediment-water interface (DOsw), the DO in BOD bottles was fixed at the sampling site and quantified volumetrically in the laboratory following the Winkler method [23]. The difference between measured DO and pure water DO at saturation under similar conditions was used to calculate the dissolved oxygen deficit [24]. Nitrate concentrations in water and sediment samples were determined using the brucine suphanilic acid and phenol di-sulphonic acid method, respectively [25,26], while ammonia was measured following the phenate method [27]. Total nitrogen (TN) was measured using the Kjeldahl method, while sulfate (SO42−) concentration was determined by the turbidimetry method. Total organic carbon (TOC) was quantified using the Walkley and Black method [28] and a TOC analyzer (LOTIX combustion TOC analyzer, Teledyne Tekmar, US16161003, Mason, OH, USA). Phosphate was estimated as per Murphy and Riley [29]. Chlorophyll-a, extracted in acetone, was determined spectrophotometrically [30] and conductivity using a multiparameter tester (Model 161E, Electronics India, Ambala Cantt, India).
The sediment P-release was estimated through controlled incubation studies. Here, the core samples were placed in a settling column (height: 50 cm; diameter: 9.6 cm) and kept in the dark for 72 h. Water collected from the corresponding sampling site was then carefully added above the sediment cores. The overlying water was mechanically stirred gently to avoid stratification effects [31]. During incubation, the temperature was maintained to the field conditions. To evaluate the impacts of climate warming, replicates of three sets were prepared and incubated at two levels of temperature rise (+1 °C and +2 °C) alongside the normal corresponding temperature (28.20–28.80 °C) incubation set-up. The initial and periodic quantification of reactive P concentration was performed according to the ammonium molybdate-stannous chloride method. This method relies on a chemical extraction process followed by direct spectrophotometric analysis [23]. For measuring sediment-P flux, samples were collected at 12 h intervals, and sediment-P fluxes were calculated from the increase in the concentration of P in the overlying water during incubation. The flux was quantified using a mass-balance approach, considering the remaining P in the water after completion of incubation and the amount removed during sampling.
For heavy metal analysis, sediment samples were dried at room temperature, homogenized, and sieved (2-mm mesh). After digestion in a tri-acid mixture at a ratio of 5:1:1 (HNO3/HCl/HClO4) in a microwave digestion system (SINEO model MDS-6G 06G623, Shanghai, China), the samples were analyzed in a Perkin Elmer atomic absorption spectrophotometer (Analyst 800, Parkin Elmer, Shelton, CT, USA). The detection limits were 0.0008 (Cd), 0.003 (Cr), 0.001 (Cu), 0.006 (Ni), 0.015 (Pb), and 0.001 (Zn) mg/L. The standard stock solutions and drift blanks (Sisco Research Laboratories) were used to calibrate the atomic absorption spectrophotometer (AAS) for the respective metal. For spiking and recovery of samples, standard solutions were prepared using nitrate salts of Cd, Cr, Ni, and Pb and granules of Zn and Cu (99% purity). Different tri-acid digestion ratios were evaluated to optimize metal recovery, and the 5:1:1 acid mixture yielded an average recovery efficiency of approximately 99%. Microbial biomass C (Cmic) was determined by the chloroform fumigation extraction procedure [32]. Phenol oxidase was determined as described by Sinsabaugh and Findlay [33], and alkaline phosphatase (AP) as per Tabatabai and Bremner [34]. The β-d-glucosidase was assayed following Eivazi and Tabatabai [35], while nitrate reductase was assayed following Reddy and Angelo [36].
The CO2 emission at the land-water interface (LWI) was collected in steel chambers (height: 23 cm; diameter: 22 cm). Each chamber was equipped with a small fan to distribute air and a thermometer to record temperature. The chambers were inverted and fixed 5 cm deep to ensure a seal against ambient air, and the gas was withdrawn through a rubber fitted valve. For quality control and to avoid changes in temperature and moisture regime, attempts were made to collect samples at identical times. A polypropylene syringe with a three-way stopper was used to withdraw gas from the headspace at 1-h intervals. Samples were brought in an icebox and analyzed in a Trace 1110 Thermo Fisher Analyzer, Dreieich, Germany. The accuracy was validated by repeated calibration with standard gas samples. The CO2 flux (mg·m−2·h−1) was quantified using the rate of change in CO2 concentration within the chamber, headspace volume, atmospheric pressure, temperature, and the universal gas constant.
Atmospheric deposition (AD) of nutrients was monitored over a 4-year period (2021–2024). The nutrient deposition was measured with bulk samplers made up of 5 L high density polyethylene bottles, equipped with Teflon funnels. To prevent bird nesting and external contamination, the samplers, devised with PVC needles, were maintained at a height of 2 m and samples collected at fortnightly intervals following an identical protocol. Thymol was used as a biocide in the collection bottle to prevent changes in nutrient concentration [37]. Prior to analysis, the funnels were rinsed with distilled water to recover particles deposited on the funnel walls. A 50 mL sample was collected in the bottle, and a 50 mL sample of the rinsing water was filtered using a pre-combusted Whatman glass fiber filter (0.7 µm). The concentrations of nitrate (NO3−), ammonium (NH4+), sulfate (SO42−), and phosphate (PO43−) were measured in filtered samples spectrophotometrically.
2.5. Statistical Analysis
All measured variables are presented as mean values ± standard error (SE). Samples of water and sediment were collected in triplicate from three sub-sites of each station (n = 18 for each year). As the samples were collected during summer low flow, a period of minimum variance, we consider n rather than n − 1 (Bessel’s correction) when calculating the SE. Correlation coefficients and dynamic fit regression models were used to evaluate relationships between total heavy metal concentrations and enzyme activities. Correlation significance was estimated at p < 0.05, 0.01, and 0.001. Principal component analysis (PCA) was employed (Past; version 3.0) to identify major environmental variables governing biogeochemical patterns across the study sites. Variables were standardized before analysis. Multivariate statistical analysis (MANOVA; Wilks’ Lambda test) was performed in SPSS (version 27) to test the effects of site, year, temperature, and their interactions. Statistical significance was evaluated at a confidence level of 95% (p < 0.05). Statistical analyses and graphical visualizations were performed using SigmaPlot (version 15.0) and IBM SPSS Statistics 20.
3. Results and Discussion
3.1. Atmospheric Deposition
The Indo-Gangetic Plains (IGP) in South Asia are characterized by high atmospheric aerosol loading and pronounced seasonal variability in atmospheric composition due to intensive urbanization, industrial activity, and agricultural emissions [38,39]. Consistent with these regional characteristics, substantial spatial variability in atmospheric nutrient deposition was observed across the study sites (Figure 2). Atmospheric deposition of nitrate (AD–NO3−) in the watershed ranged from 92.4 (Shlktr) to 168.6 (Jjmu) µmol·m−2·yr−1. Similarly, deposition of ammonium (AD–NH4+) ranged from 78.2 (Shlktr) to 325.4 (Jjmu) µmol·m−2·yr−1, phosphate (AD–PO43−) from 3.2 (Shlktr) to 17.4 (Jjmu) µmol·m−2·yr−1, and sulfate (AD–SO42−) from 5.8 (Shlktr) to 20.8 (Jjmu) µmol·m−2·yr−1. On the spatial scale, annual atmospheric deposition-driven nitrogen (AD–N) and phosphorus (AD–P) inputs were higher at Jjmu and Rjht, followed by Vrna and Sngm, whereas Nwbj and Shlktr exhibited comparatively lower values.
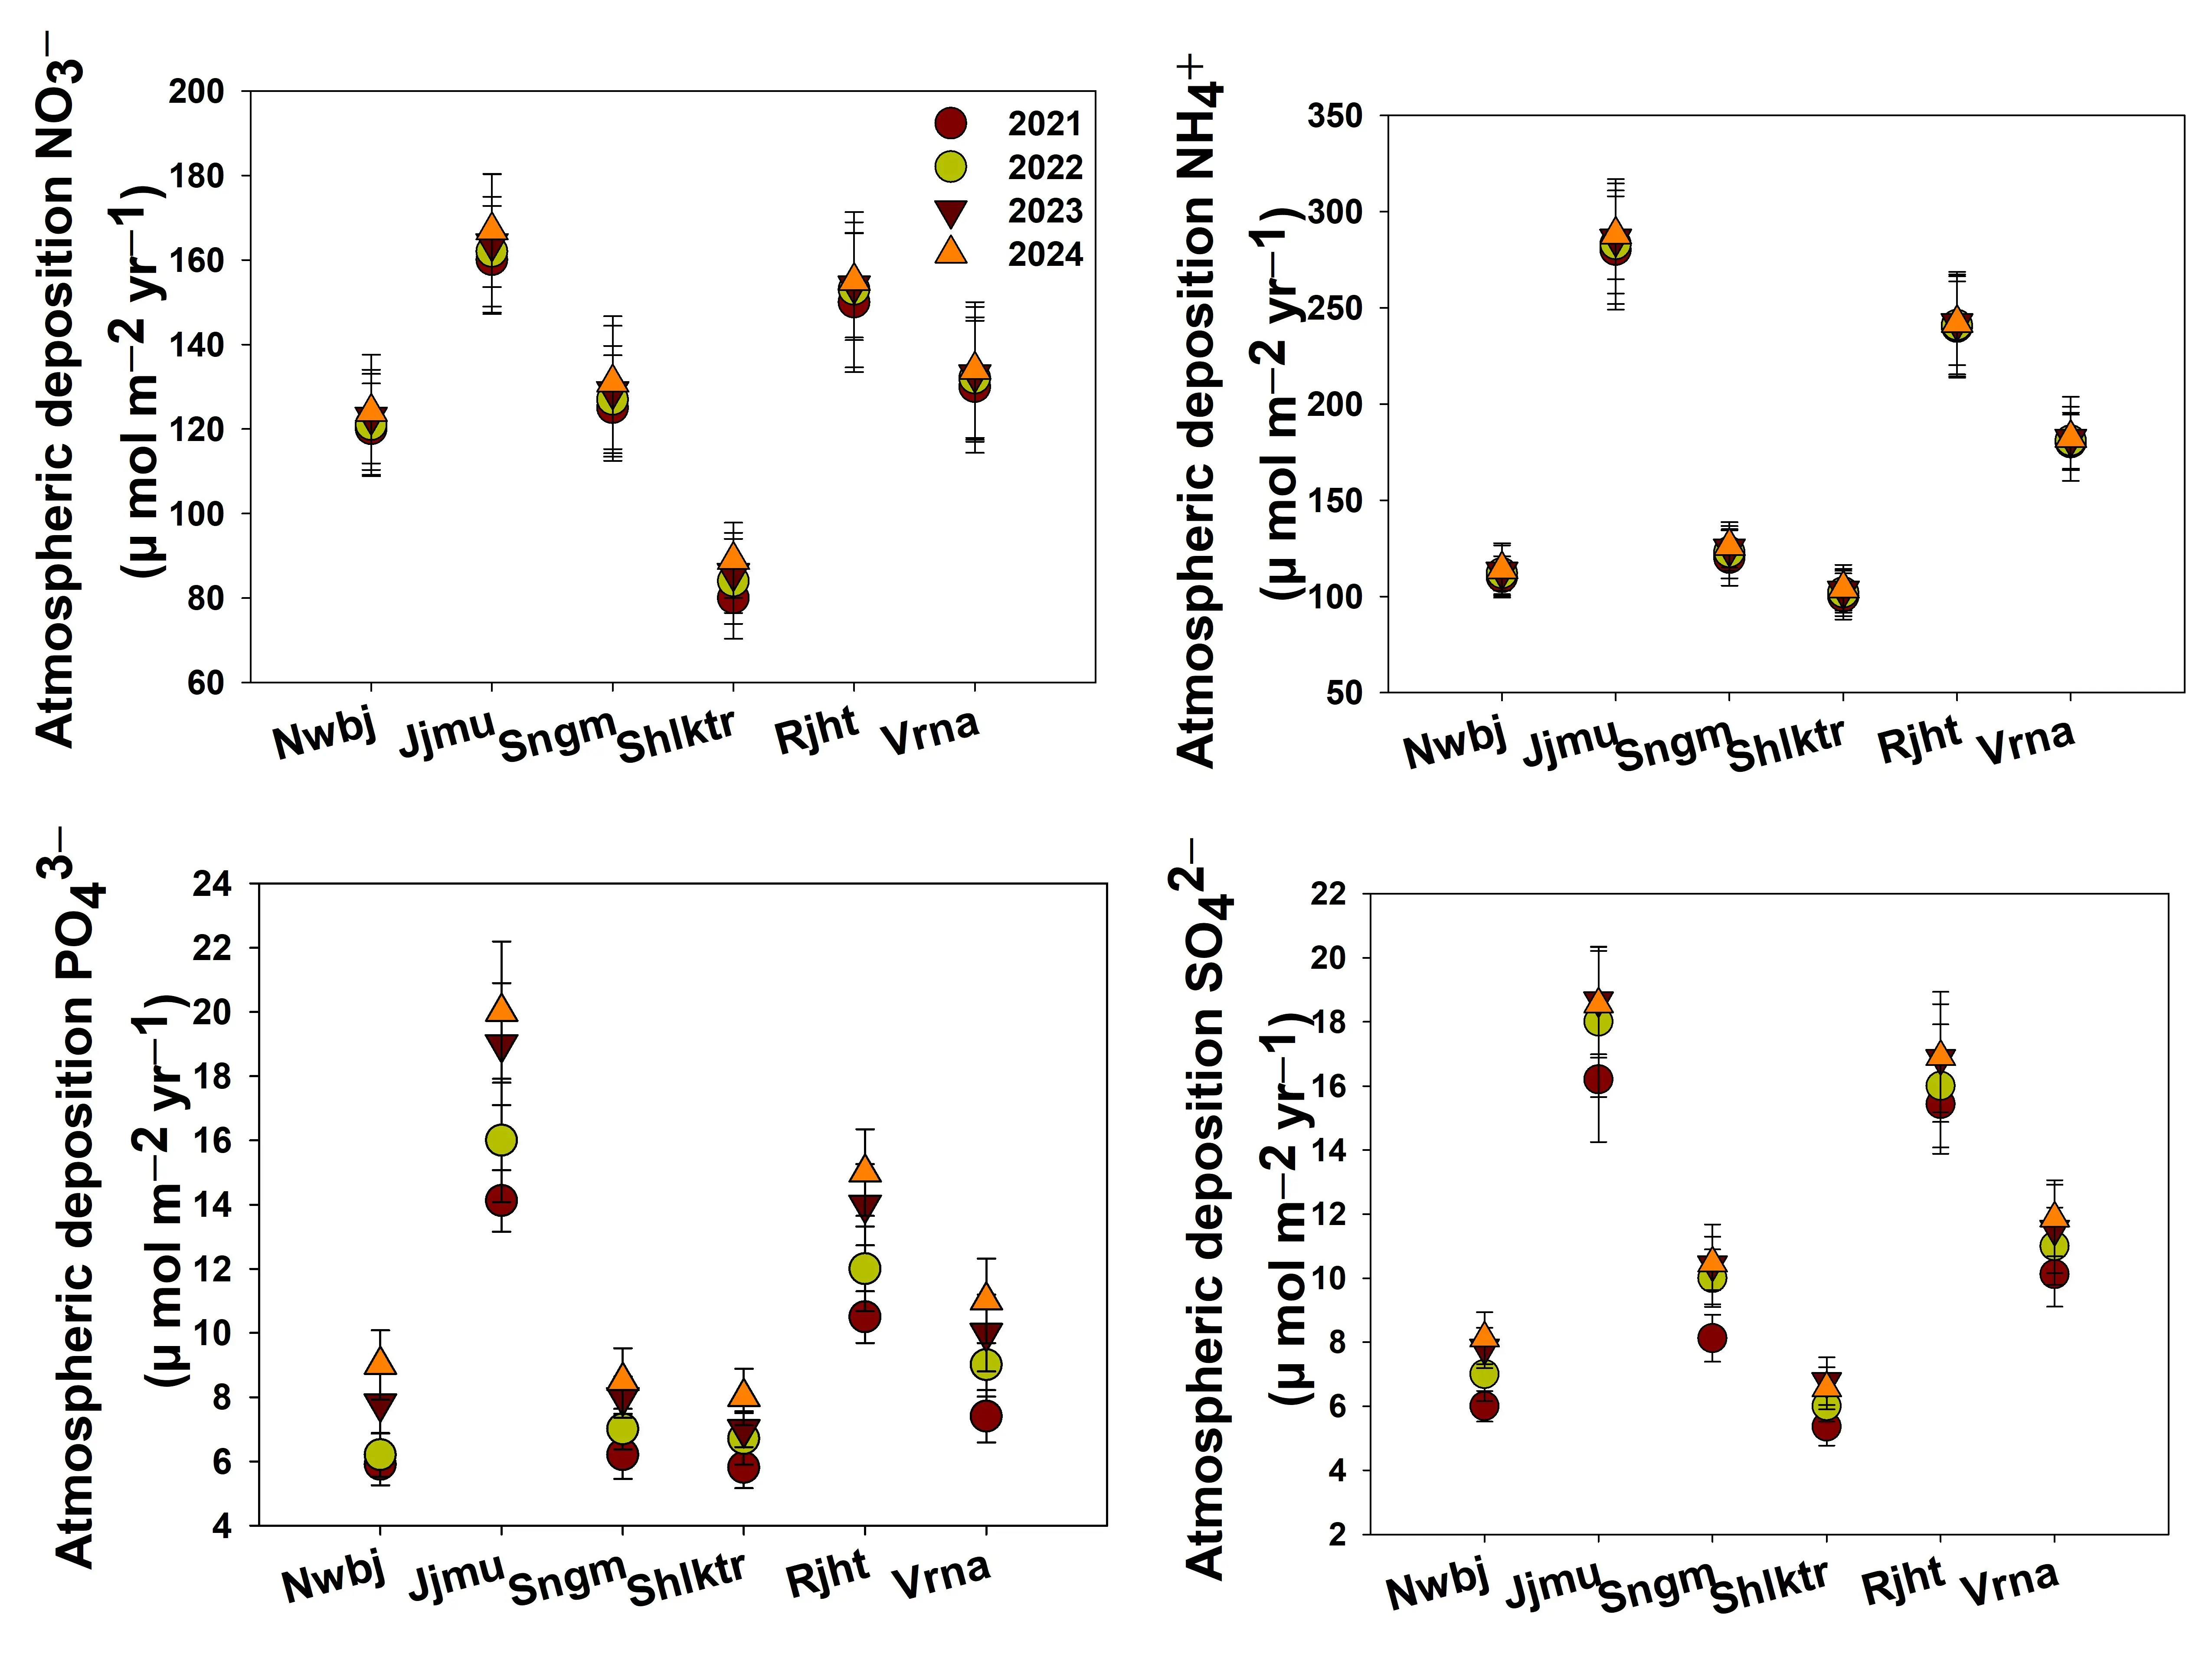
Figure 2. Spatio-temporal variations in the rate of atmospheric deposition of major nutrient ions in the Ganga River Basin.
Overall, the minimum depositions were consistently recorded at Shlktr and the maximum at Jjmu. Between 2021 and 2024, the overall AD–NO3−, AD–NH4+, AD–PO43−, and AD–SO42− increased by approximately 42%, 48%, 55%, and 39% respectively. Progressive increase in atmospheric deposition of reactive nitrogen and phosphorous across the study period suggests increasing anthropogenic influence.
Our previous studies show that the Ganga River Basin receives about 2.77 Tg of reactive N and 130 Gg of reactive P input through atmospheric deposition [40,41]. Direct input on the water surface enhances riverine productivity, whereas from the watershed, it enhances DOC flushing through runoff [42], and both collectively constrain benthic concentrations of dissolved oxygen [10].
3.2. Water Quality Attributes
The physicochemical characteristics of water revealed strong spatial heterogeneity across the study stretch of the Ganga River (Table 1). The pH remained slightly alkaline at all sites (7.59–8.84), with the highest average at Jjmu (8.10 ± 0.51), suggesting potential for higher microbial activity and phosphorus mobility. Conductivity, salinity, and total dissolved solids (TDS) were found to be consistently high at Jjmu and Rjht, reflecting higher ionic load and pollution burden from urban-industrial discharge.
Table 1. Physicochemical characteristics of water at different sampling sites of the Ganga River during the low flow period.
|
Parameters |
Nwbj |
Jjmu |
Sngm |
Shlktr |
Rjht |
Vrna |
|---|---|---|---|---|---|---|
|
pH |
7.60–7.77 7.64 ± 0.43 |
7.78–8.84 8.10 ± 0.51 |
7.67–8.06 7.85 ± 0.49 |
7.59–7.77 7.69 ± 0.5 |
7.71–8.21 7.91 ± 0.51 |
7.69–8.09 7.89 ± 0.5 |
|
Conductivity (µS·cm−1) |
292–338.67 314.25 ± 18.5 |
440.14–511.36 472.27 ± 29.93 |
319.89–399.39 373.59 ± 24.63 |
289.71–329.67 312.67 ± 21.06 |
390.73–4335.12 417.69 ± 28.04 |
292.71–353.67 356.67 ± 21.06 |
|
Salinity (ppm) |
102–123.24 112.66 ± 6.56 |
151.05–185.49 167.92 ± 10.97 |
117.96–142.42 129.35 ± 8.23 |
92.90–115.88 104.55 ± 7.11 |
125.91–152.69 139.30 ± 9.37 |
100.90–125.88 104.55 ± 7.11 |
|
TDS (ppm) |
210–240.48 227.06 ± 13.4 |
295.09–358.95 330.58 ± 21.32 |
274.90–319.71 298.66 ± 19.33 |
205.79–236.76 221.11 ± 14.87 |
301.79–338.32 321.64 ± 21.62 |
255.79–266.76 241.11 ± 16.87 |
|
CO3− (ppm) |
0.96–1.40 1.21 ± 0.06 |
4.10–4.91 4.44 ± 0.28 |
1.29–1.77 1.58 ± 0.1 |
0.97–1.30 1.16 ± 0.08 |
2.39–3.49 2.95 ± 0.2 |
1.97–2.30 2.16 ± 0.08 |
|
Free CO2 (ppm) |
0.45–0.79 0.58 ± 0.03 |
3.20–4.11 3.57 ± 0.22 |
0.70–1.13 0.89 ± 0.05 |
0.48–0.91 0.68 ± 0.04 |
2.39–3.39 2.92 ± 0.20 |
0.78–2.91 1.68 ± 0.06 |
|
HCO3− (ppm) |
8–32.06 19.49 ± 1.24 |
26.00–65.17 48.48 ± 3.61 |
11.99–36.85 24.45 ± 1.8 |
7.99–28.97 16.74 ± 1.18 |
22.98–52.89 38.75 ± 2.83 |
15.99–36.97 20.74 ± 2.18 |
Conductivity ranged from 289.71 to 511.36 µS·cm−1 across the study sites, with the highest mean value observed at Jjmu (472.27 ± 29.93 µS·cm−1), followed by Rjht (417.69 ± 28.04 µS·cm−1). Similarly, salinity and TDS exhibited maxima at Jjmu, with mean values of 167.92 ± 10.97 ppm and 330.58 ± 21.32 ppm, respectively. Concentrations of carbonate (CO3−2), free CO2, and bicarbonate (HCO3−) were substantially higher at Jjmu and Rjht compared with the relatively less-disturbed sites. Free CO2 concentrations ranged from 0.45 to 4.11 ppm, while HCO3− concentrations varied between 7.99 and 65.17 ppm across the study stretch. The elevated free CO2 and bicarbonate concentrations at Jjmu and Rjht likely reflect intense organic matter decomposition, microbial respiration, and enhanced carbon mineralization associated with high organic loading.
Concentrations of dissolved nutrients exhibited marked spatial and temporal variability across the study sites (Figure S1). The nutrient (NO3−, PO43−, SO42−, NH4+ and TN) concentrations were found highest (381.23 µg·L−1, 199.81 µg·L−1, 142.34 µg·L−1, 37.81 µg·L−1, and 1.43 mg·L−1 respectively) at Jjmu and the lowest (208 µg·L−1, 98.71 µg·L−1, 60 µg·L−1, 12 µg·L−1, and 0.34 mg·L−1 respectively) at Shlktr. The total organic carbon (TOC) concentrations ranged from 13.21 to 27.34 mg·L−1. The synchronous increase in TOC and nutrient concentrations indicates strong coupling between organic enrichment and nutrient accumulation. Heavy metal concentrations exhibited spatial patterns broadly similar to those observed for nutrient distributions, with consistently higher concentrations at Jjmu and comparatively lower concentrations at the relatively less-disturbed Shlktr (Figure S2). Zinc showed the highest concentration (160 µg·L−1) and Cd, the lowest (2.21 µg·L−1). Metal concentrations at Jjmu were approximately 2.32–7.12 times higher than those measured at Shlktr, indicating substantial anthropogenic enrichment associated with industrial discharge and urban effects [43].
Sestonic chlorophyll-a (Chl-a) concentrations exhibited marked spatial variability across the study sites, with maxima (46.56 µg·L−1) at Sngm and minima (22.13 µg·L−1) at Shlktr (Figure S3a). Gross primary productivity (GPP) followed a similar spatial pattern, with maximum productivity at Sngm (13.43 mg·C·m−2·h−1) and minimum at Shlktr (6.56 mg·C·m−2·h−1) (Figure S3b). The elevated Chl-a biomass and GPP at Sngm likely reflect enhanced nutrient availability and favorable conditions for primary production associated with confluence-driven supply of nutrients.
Dissolved oxygen at the sediment-water interface (DOsw) showed a spatial trend opposite to nutrient enrichment and organic loading (Figure S3c). The highest concentration of DOsw was found at Shlktr (4.32 mg·L−1), and the lowest at Jjmu (1.87 mg·L−1), whereas an opposite trend appeared for DODsw with maxima (7.67 mg·L−1) at Jjmu and minima (4.22 mg·L−1) at Shlktr. High DODsw at Jjmu and downstream sites suggests intensified microbial respiration and organic matter decomposition under polluted conditions. Such oxygen-depleted conditions may alter redox-sensitive sediment processes, including internal phosphorus release and altered nutrient recycling within the river system.
3.3. Sediment Characteristics, Carbon Dynamics and Oxygen Linkages
Sediment-P release exhibited substantial spatial variability across the study sites, ranging from 1.2 to 10.2 mg·m−2·day−1, with the highest release observed at Jjmu and the lowest at Shlktr (Figure S3f). Spatially, sediment-P release showed an inverse relationship with dissolved oxygen concentration at the sediment-water interface (DOsw).
The concentration of readily mineralizable carbon in sediments ranged from 146.21 µg·C·g−1 at Shlktr to 415.67 µg·C·g−1 at Jjmu, while recalcitrant carbon varied between 99.45 µg·C·g−1 (Shlktr) and 231.25 µg·C·g−1 (Jjmu). The CO2 flux at the land-water interface varied between 78.98 mg·m−2·h−1 (Shlktr) and 275.63 mg·m−2·h−1 (Sngm). The emission flux increased marginally over time. Notably, CO2 emission at Sngm was approximately twofold higher than that observed at Jjmu, suggesting enhanced carbon mineralization and respiratory activity in the confluence region. Microbial biomass carbon also varied substantially among the sampling sites, with the highest value observed at Sngm (332.18 µg·g−1) and the lowest at Nwbj (128.91 µg·g−1) (Figure S4). The elevated microbial biomass and CO2 fluxes at Sngm likely reflect increased substrate availability and enhanced microbial processing associated with nutrient-rich mixing zones and enhanced organic matter turnover.
Readily mineralizable carbon at Jjmu was over 3-folds higher than that at Shlktr, whereas recalcitrant carbon was nearly 2.3-fold higher, indicating Jjmu as a hotspot of carbon enrichment. Atmospheric deposition N:P ratios declined by 20–30% between 2021 and 2024 at several sites, indicating progressively increasing phosphorus enrichment relative to nitrogen. River water N:P ratios at Jjmu and Rjht were 3 to 4 folds lower than those at Shlktr. Moreover, Jjmu and Rjht displayed high C:N ratios (21.28 in water and 16.64 in sediment). Specifically, river water C:N ratios at Jjmu and Rjht were approximately twofold higher than those observed at Shlktr (Figure 3).
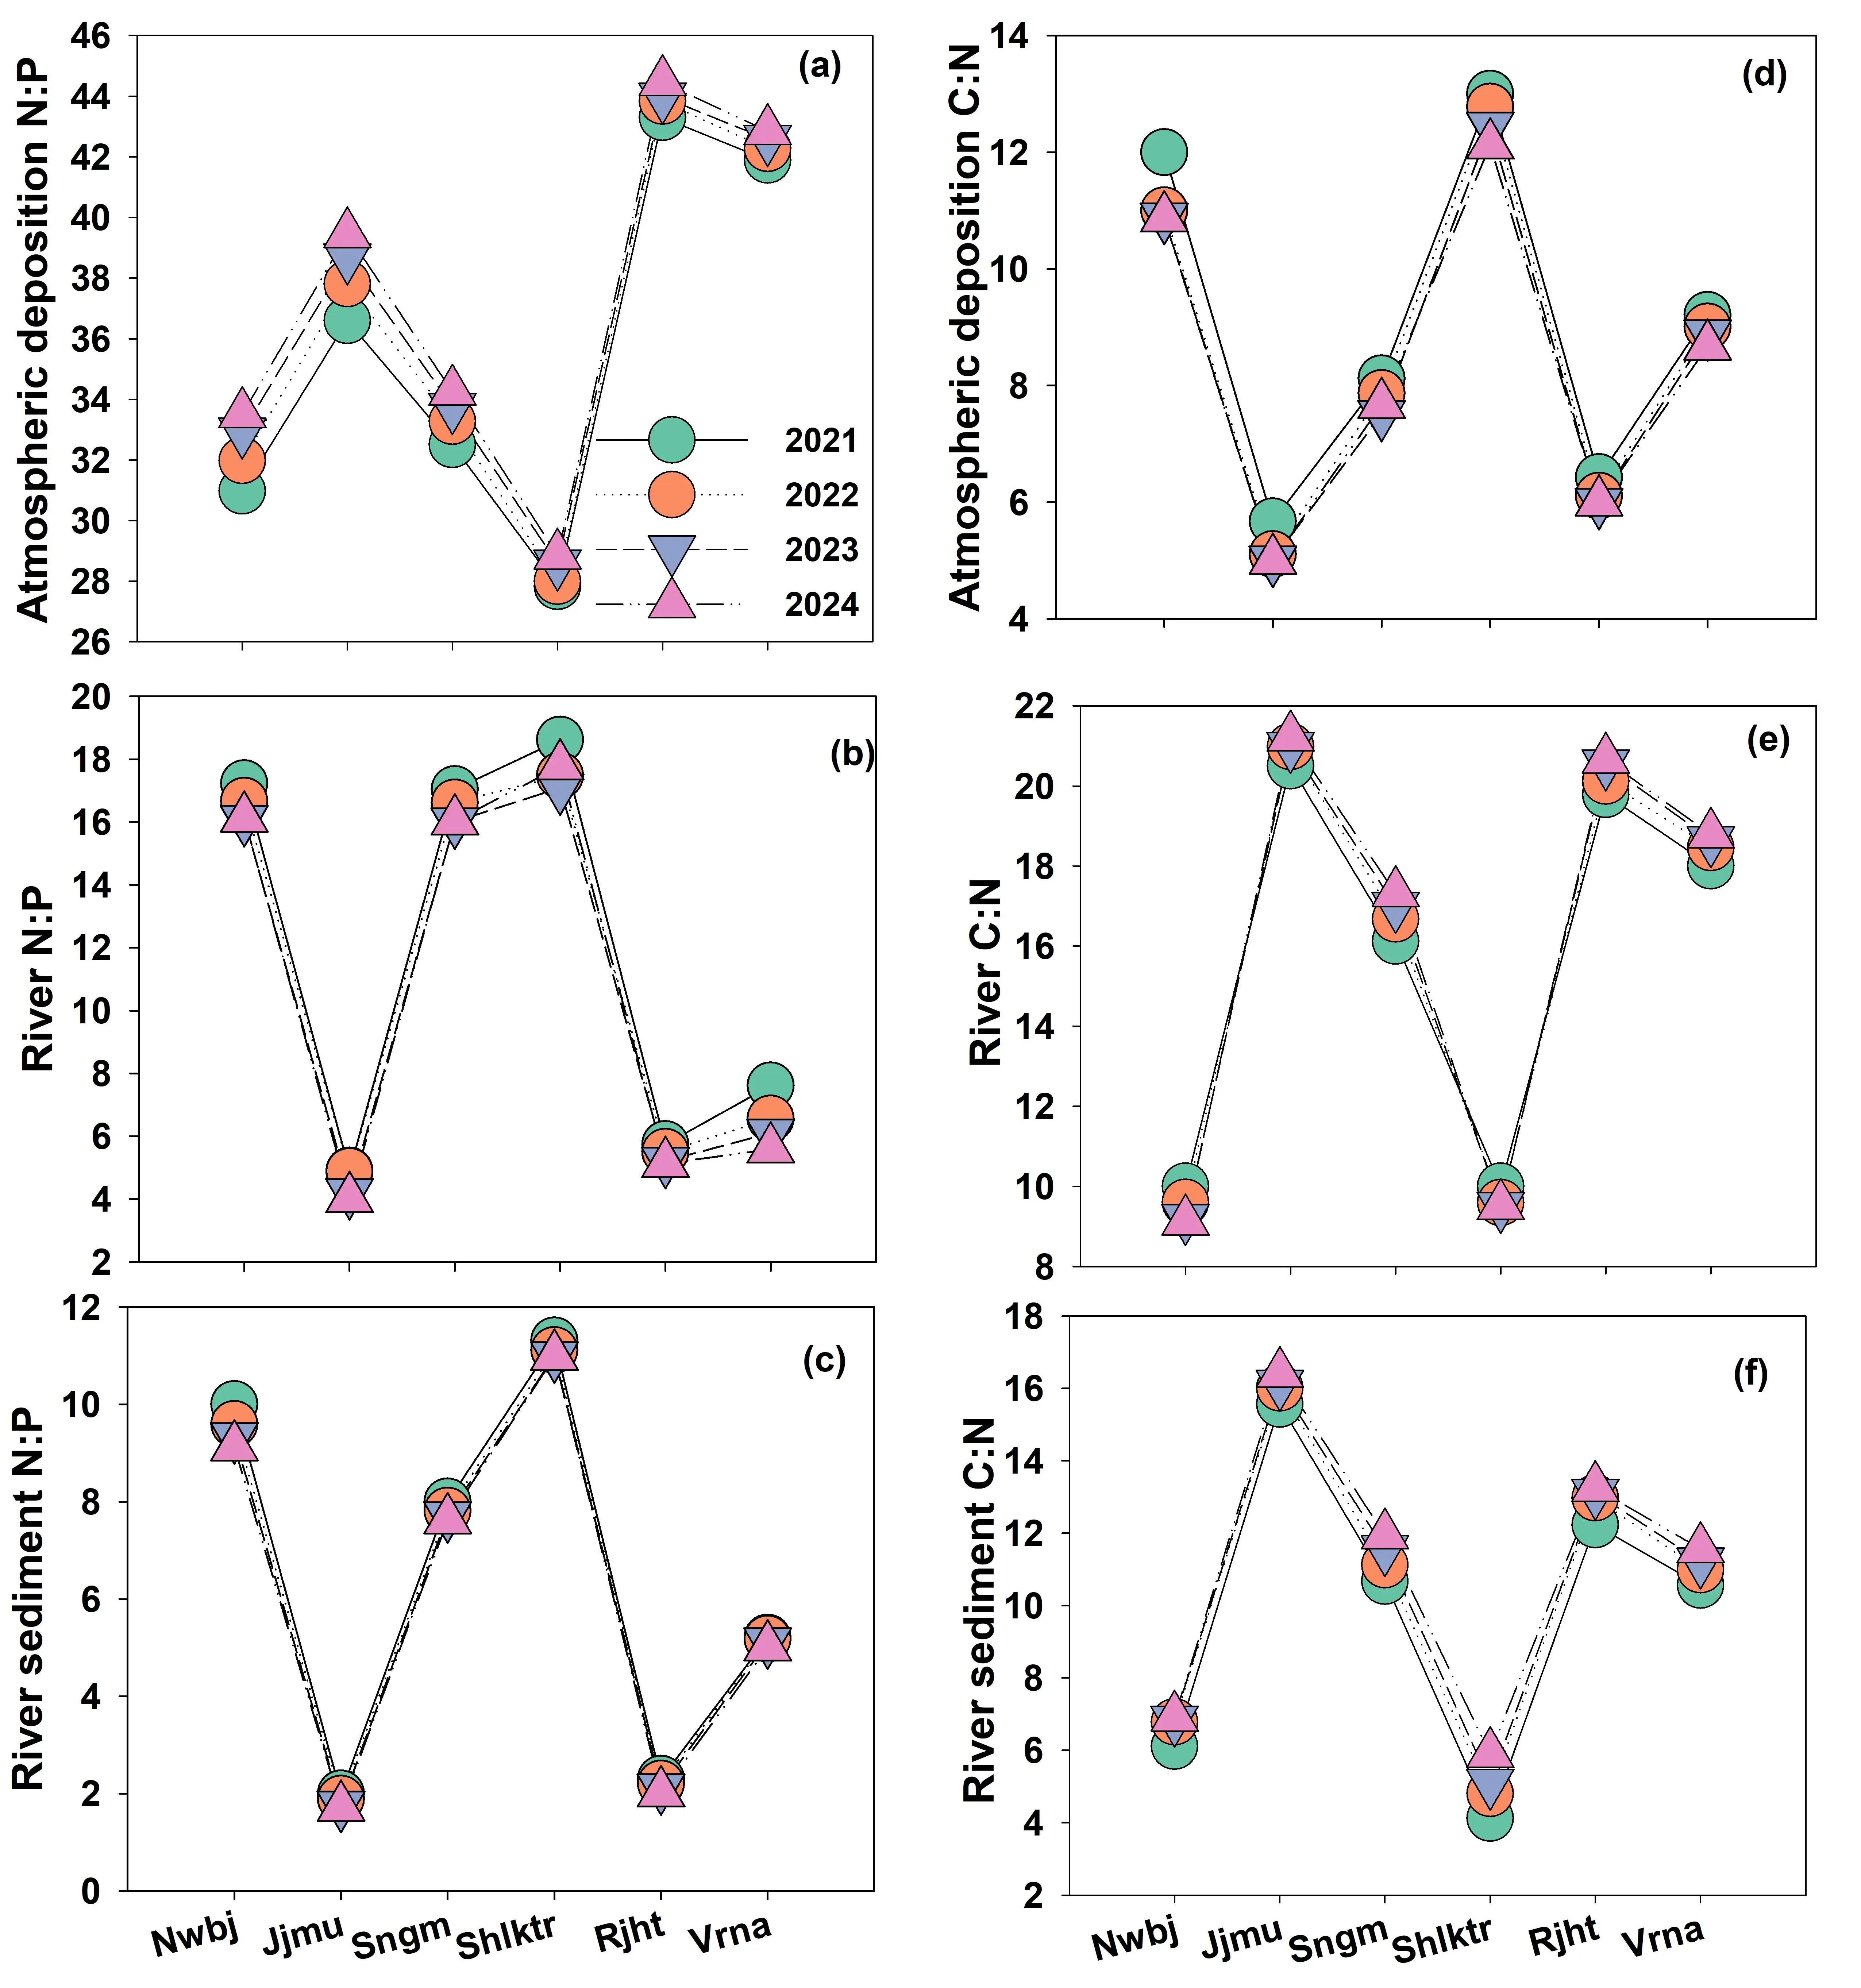
Figure 3. N:P stoichiometric ratio in: (a) atmospheric deposition (b) river water (c) river sediment and C:N ratio in: (d) atmospheric deposition (e) river water and (f) river sediment in the Ganga River.
The elevated microbial biomass and labile carbon concentrations at Sngm were accompanied by substantially higher CO2 fluxes, indicating increased microbial respiration and active carbon turnover at the confluence zone. Elevated CO2 emissions suggest that a considerable fraction of organic carbon was lost through respiration rather than retained by the all as biomass (reduced apparent carbon use efficiency). In contrast, Jjmu exhibited high concentrations of both readily mineralizable and recalcitrant carbon but comparatively lower microbial biomass and CO2 fluxes, indicating the effect of other stressors [44].
River water and sediment C:N ratios also appear high at Jjmu, reaching 21.28 and 16.64, respectively, suggesting substantial organic carbon enrichment relative to nitrogen. High C:N ratios may constrain microbial processes and the efficiency of microbial carbon utilization (lower apparent carbon use efficiency). The abundance of readily mineralizable carbon promotes rapid microbial degradation and substantial oxygen demand at the sediment-water interface, whereas the persistence of recalcitrant carbon sustains sedimentary C-accumulation. These patterns indicate strong coupling among organic carbon accumulation, microbial carbon degradation, and oxygen depletion, particularly at nutrient-enriched sites, with likely impacts on redox-dependent processes at the sediment-water interface.
3.4. Enzyme Activities
Alkaline phosphatase activity (APA) exhibited pronounced spatial variability across the study sites and showed an inverse relationship with phosphate concentration. The activity of this microbial enzyme was found to be the highest (380.12 µm·p-Np·g−1·h−1) at Shlktr and lowest (90.45 µm·p-Np·g−1·h−1) at Jjmu (Figure 4).
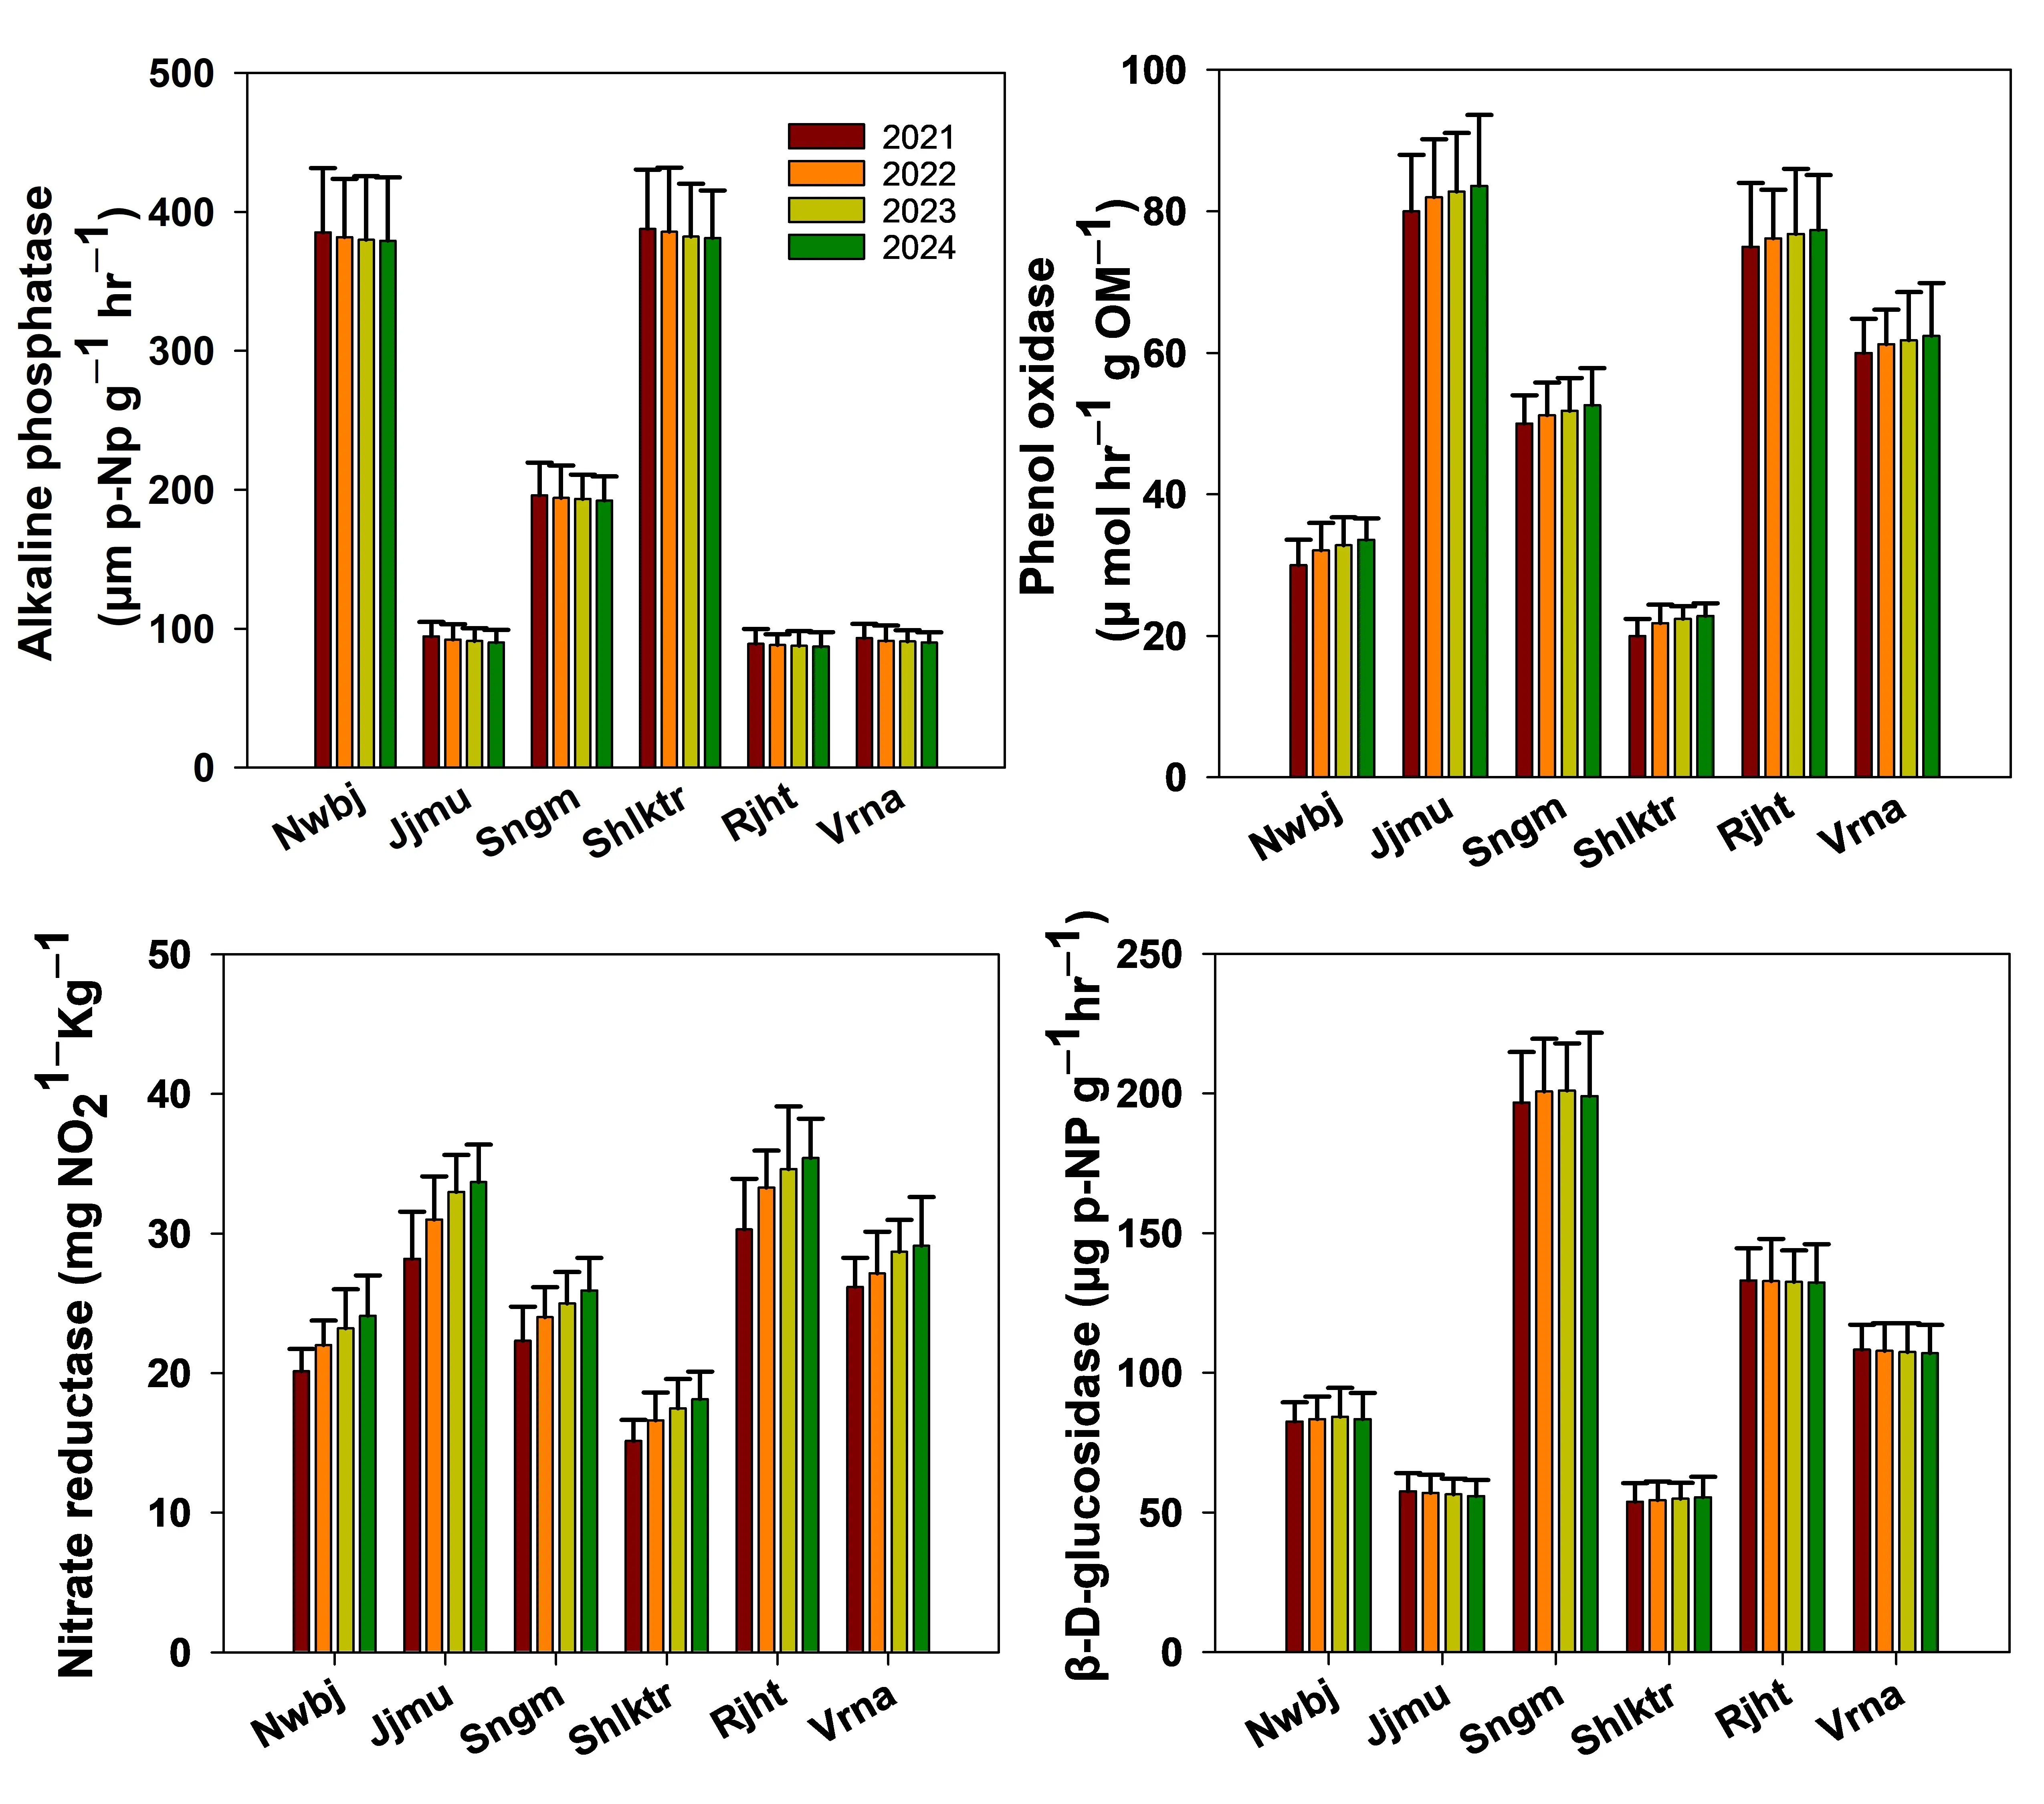
Figure 4. The spatial and temporal variations in the activities of extracellular enzymes assayed in the river sediment.
The reduced APA at nutrient-enriched sites indicates lower microbial activity with respect to enzymatic phosphorus acquisition. In contrast, elevated APA at Shlktr indicates enhanced microbial phosphorus acquisition under a relatively phosphorus poor condition. This is consistent with previous studies demonstrating enzymatic upregulation under phosphorus deficiency [45]. Similar findings have been reported for riverine sediments, where alkaline phosphatase activity acts as a sensitive indicator of P availability [46].
The activity of nitrate reductase ranged from 15.12 mg·NO2−·Kg−1 to 35 mg·NO2−·Kg−1 (Figure 4). Nitrate concentrations remained high at Jjmu and Rjht. Also, we found the highest activity of phenol oxidase at Jjmu (86.54 µ·mol·h−1·g·OM−1) and lowest at Shlktr (22.53 µ·mol·h−1·g·OM−1) (Figure 4). However, β-D-glucosidase activity showed asynchrony with that of phenol oxidase, with activity remaining highest at Sngm. Nitrate reductase activity showed strong correspondence with dissolved oxygen deficit (DODsw) and total organic carbon (TOC), indicating microbial activity associated with carbon-rich, oxygen-poor environments. Elevated TOC stimulates microbial respiration, leading to oxygen depletion at the SWI. Under such conditions, nitrate is expected to act as an alternative electron acceptor. These patterns suggest increased denitrification and dissimilatory nitrate reduction at nutrient-enriched sites. Phenol oxidase activity indicated enhanced oxidative degradation of complex and recalcitrant organic matter under elevated organic loading [47]. Collectively, these findings suggest strong coupling among organic carbon enrichment, oxygen depletion, and microbial processes in the river.
Principal component analysis (PCA) was used to elucidate mechanistic linkages between eutrophication, metal pollution, and extracellular enzyme activities (Figure 5). PC1 explained 76.54% of the total variance and showed the impact of anthropogenic forcing segregating Jjmu, the most polluted site, far away and opposite to Shlktr, the least polluted site. The activity of alkaline phosphatase did appear opposite to the concentration of phosphate as well as sediment-P release, a redox dependent process. The β-d-glucosidase appears segregated towards C rich sites such as Sngm and Rjht, although relatively away from the phenol oxidase, indicating that the former is more sensitive to metal pollutants compared to the latter. However, the negative relationship between β-d-glucosidase and metal pollutants, once thresholds are reached, suggests the sensitivity of carbon mineralization to the metal pollution gradient. Phenol oxidase activity remained relatively closer to nutrients, metals, and C-eutrophication variables, indicating selective sensitivity and functional resilience of microbial enzymatic processes. Variables of eutrophication, such as chlorophyll a and gross primary productivity, showed relative synchrony with carbon and nutrients. Overall, eutrophication and metal stress disproportionately influenced the microbial processes that drive shifts in carbon degradation, thereby reinforcing positive feedbacks.
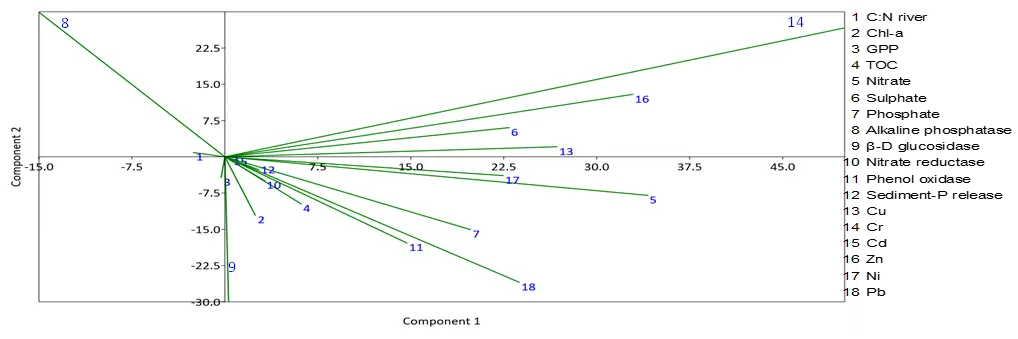
Figure 5. Principal component analysis (PCA) segregates metal pollutants, nutrient variables, and enzyme activities that explain the major proportion of the variance, linked to spatial differences in water and sediment chemistry.
3.5. Incubation Studies
Nitrate reductase activity increased progressively with experimental warming, by about 15% at 1 °C rise and nearly 22% at 2 °C rise in temperature. The activity of phenol oxidase increased in a similar pattern (Figure 6). The increased temperature sensitivity of these enzymes suggests that warming may intensify microbial nitrogen transformation and organic matter degradation in the river sediments, reinforcing back to hypoxic conditions. The CO2 emission fluxes also increased with temperature, rising up to 24% on a 2 °C rise although the microbial biomass carbon (MBC) did not show a concurrence (Figure 7).
A simultaneous increase in enzyme activity and CO2 release, together with reduced microbial biomass, suggests enhanced respiratory carbon loss under warming. These observations suggest that future climate warming, which enhances microbial enzyme activities and CO2 release, will constrain microbial community to translate a proportionate amount of C to cellular biomass.
Denitrification in aquatic ecosystems is strongly influenced by a decline in dissolved oxygen availability [48]. This study demonstrated temperature dependent acceleration of multiple interconnected biogeochemical processes, including DO depletion, increased sediment-P release, and nitrate reductase activity. These warming-induced effects appear relatively more prominent at Jjmu, Rjht, and Vrna, where carbon and nutrient loads were found to be high.
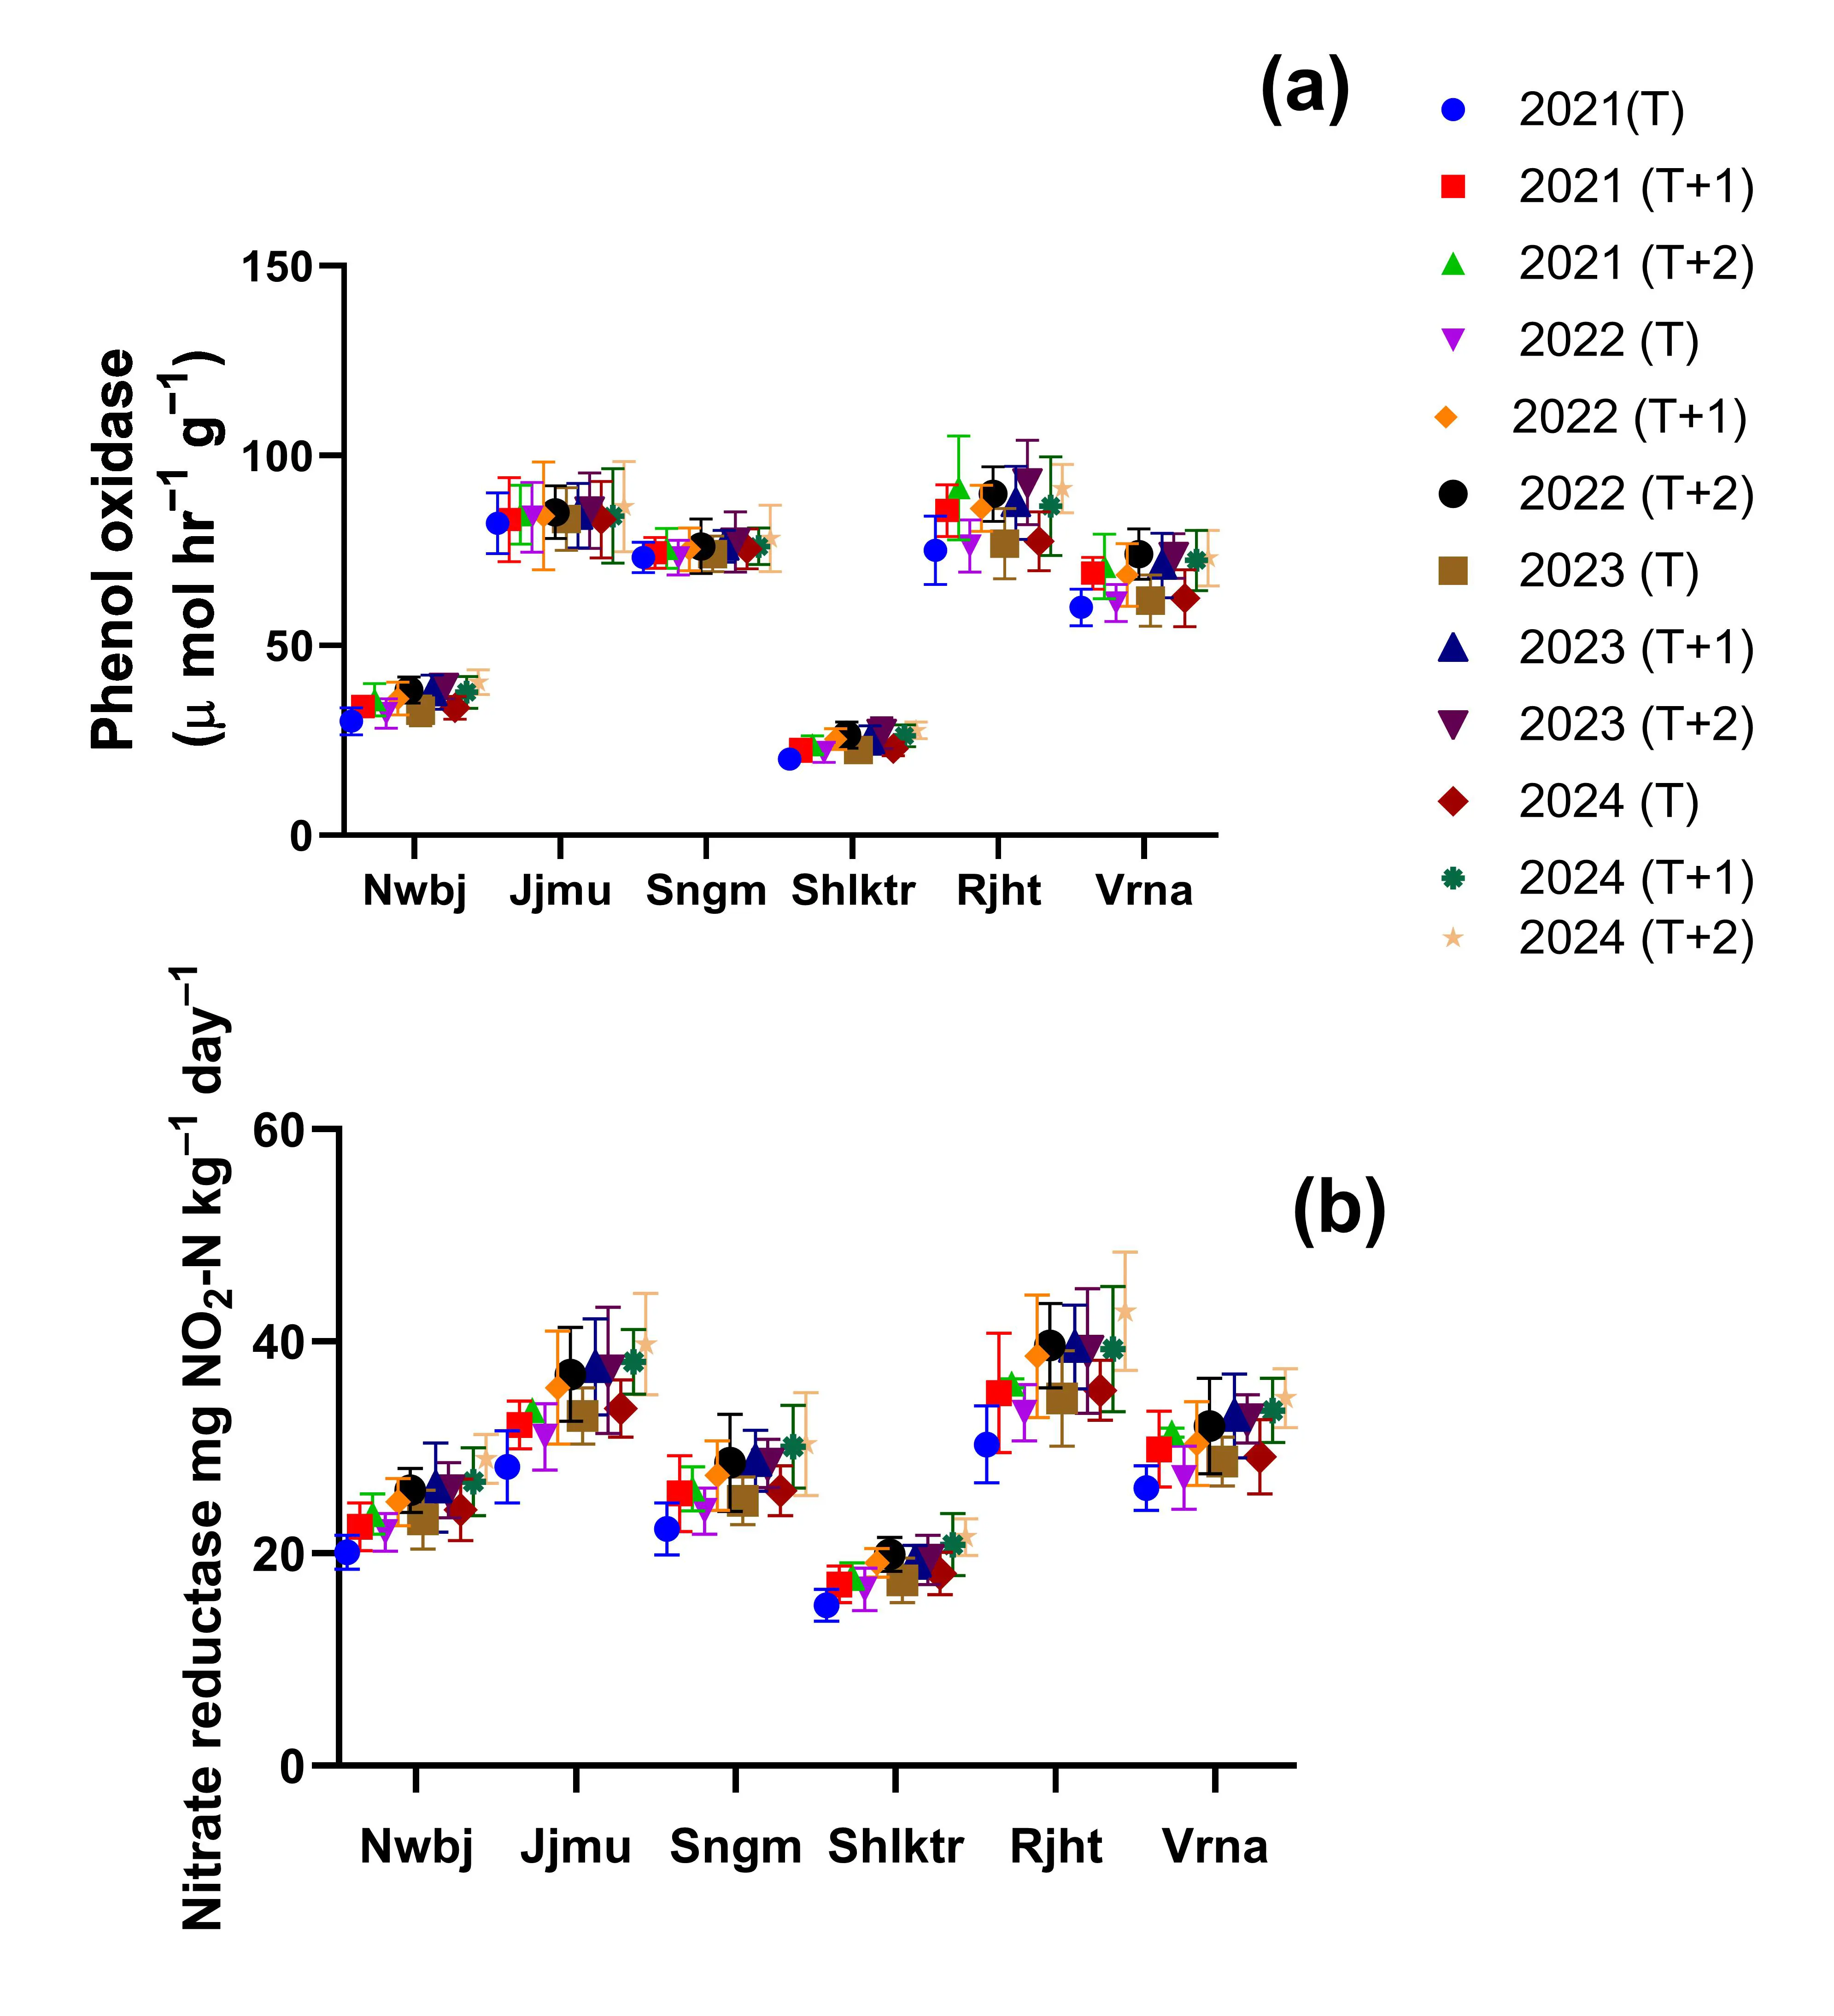
Figure 6. Effects of climate warming on nitrate reductase (a) and phenol oxidase (b) activities in sediment collected from the Ganga River.
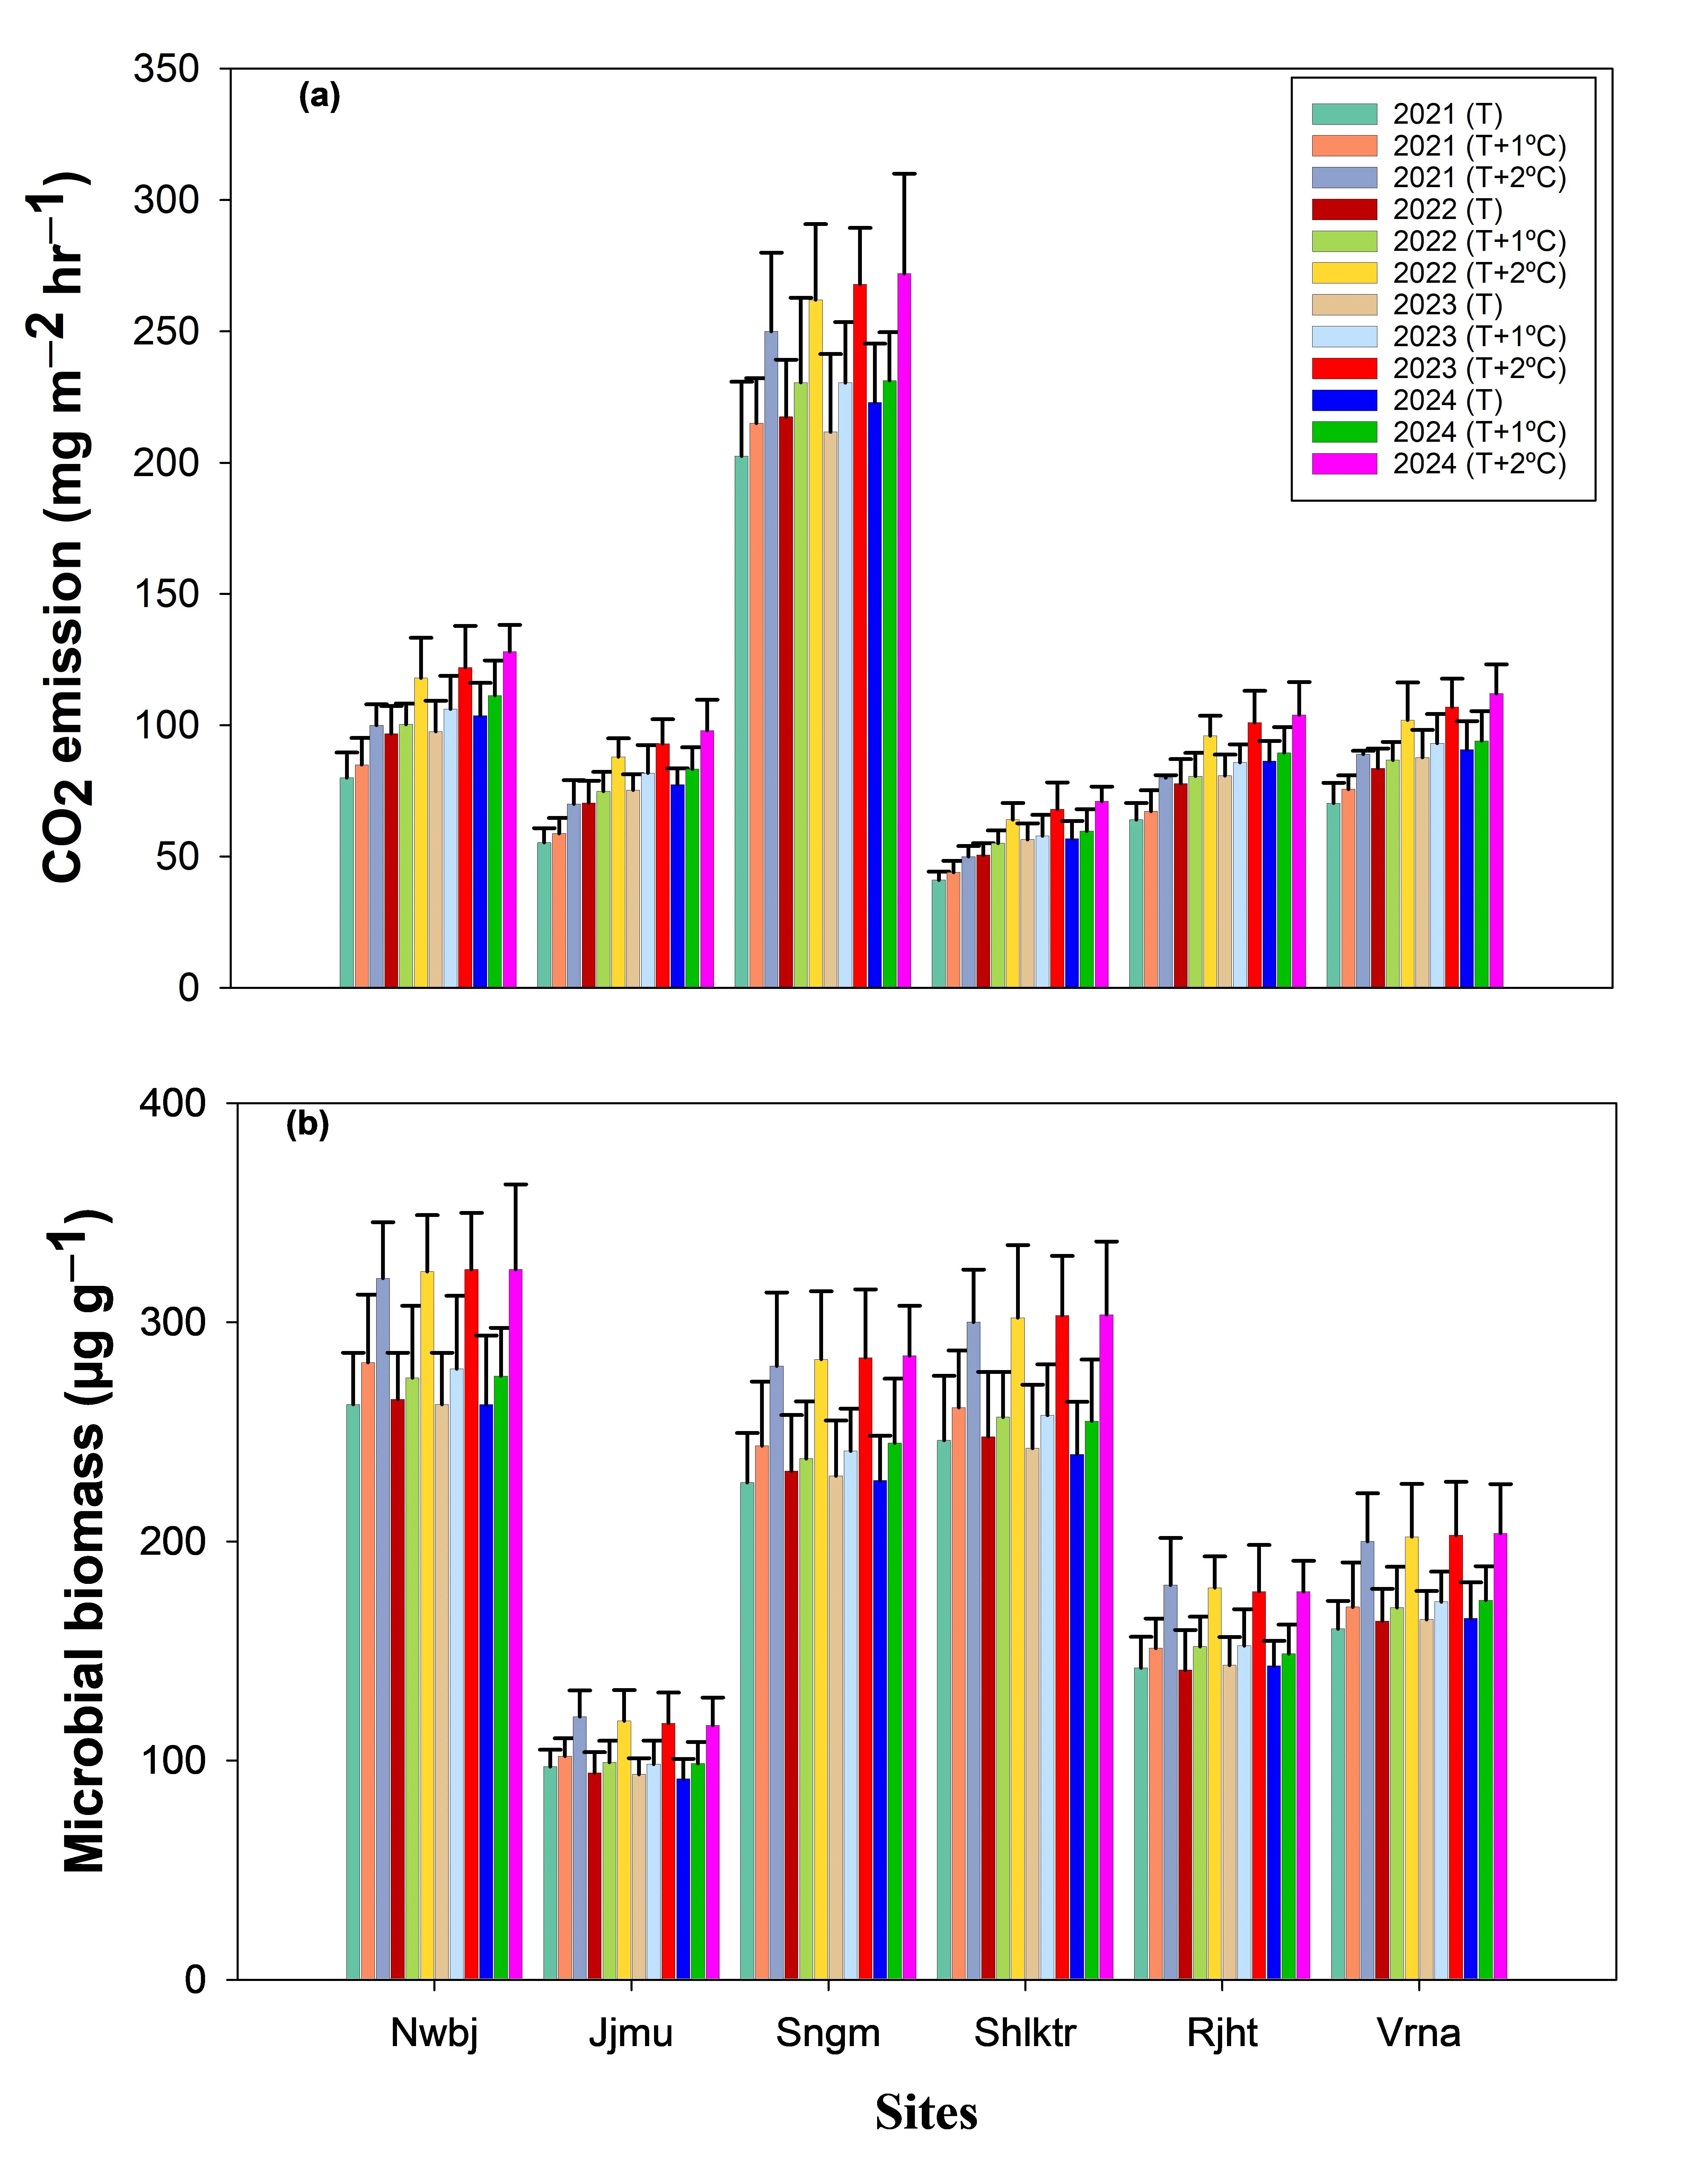
Figure 7. Effects of climate warming on CO2 emission (a) and microbial biomass carbon (b) in the Ganga River.
Previous studies have shown that warming can modify aquatic microbial and biogeochemical functioning. Ribalet et al. [49] demonstrated that Prochlorococcus productivity initially increased with temperature but declined beyond ~28 °C, suggesting that warming drives biogeochemical transformations up to a physiological limit. The amplified microbial metabolism under warmer conditions is consistent with known enzymatic Q10 responses and implies that ongoing climate warming will alter nutrient stoichiometric balance and nitrogen loss pathways in tropical rivers.
A declining trend in microbial biomass carbon (Figure 7) indicates reduced apparent carbon use efficiency (CUE) under warming conditions. Elevated temperature accelerated microbial metabolism and enzyme activities, thereby enhancing the decomposition of carbon fractions and respiratory CO2 loss. However, the concomitant decline in MBC suggests that the carbon was increasingly directed toward respiration rather than biomass synthesis. Collectively, these findings highlight that warming stimulates heterotrophic activity and CO2 flux from sediments but simultaneously constrains microbial growth efficiency, potentially destabilizing sediment carbon pools and amplifying carbon–climate feedbacks. Similar temperature-driven reductions in microbial apparent CUE and enhanced respiration have also been reported previously in aquatic sediments and soils [50].
3.6. N:P and C:N Ratios
The N:P ratio in atmospheric deposition remained above 20 across the study sites, with the lowest values at Shlktr and the highest at Jjmu. In contrast, river water N:P ratios were found below 16 at Jjmu, Rjht, and Vrna (Figure 3). The lowest river water N:P ratio was recorded at Jjmu (4.31) and the highest at Shlktr (18.62). Relative N limitation is indicated by DIN/DIP < 10 [51]. Atmospheric deposition N:P ratios showed significant positive correlations with the river N:P ratios at hypoxic (r2 = 0.74; p < 0.005) and oxic (r2 = 0.92; p < 0.001) sites. The river water N:P ratios also showed strong positive correlations with DOsw at hypoxic (r2 = 0.84; p < 0.005) as well as oxic (r2 = 0.96; p < 0.001) sites (Figure 8). Elemental variations further revealed comparatively higher P enrichment at Jjmu, Rjht, and Vrna (Figure 8). In bed sediments, the N:P ratio remained below 16 at all sites, with the highest value recorded at Shlktr (11.78) and the lowest at Jjmu (2.0) Sediment N:P ratios showed significant positive correlation at oxic sites (r2 = 0.71; p < 0.005) and negative correlation at hypoxic sites (r2 = 0.76; p < 0.005).
River water N:P ratios showed negative linear relationships with sediment-P release and sulfate concentration under oxic as well as hypoxic conditions, although the relationships were relatively stronger under hypoxia (r2 = 0.92 vs. 0.82; p < 0.001 for sediment-P release, and r2 = 0.84 vs. 0.72; p < 0.005 for sulfate) (Figure 8). These patterns indicate loss of nitrogen through denitrification, driven by oxygen-poor, carbon-rich conditions. Altered coupling of N and P cycles points to a stoichiometric imbalance sustained by sediment phosphorus release and nitrate removal under low-oxygen regimes, which weaken Fe-P associations, facilitating P mobilization from the sediments [52,53].
The C:N ratio in atmospheric deposition exhibited substantial spatial variability, with the highest value at Sngm (12.36) and the lowest at Jjmu (4.78). In contrast, the river water C:N ratio remained highest at Jjmu (21.76) and lowest at Shlktr (9.12), suggesting retention of carbon or loss of nitrogen. The concurrence of high C:N ratios, increased nitrate reductase activity, and reduced microbial biomass suggests enhanced respiratory carbon loss and altered microbial carbon processing under nutrient-enriched conditions. Overall, these stoichiometric shifts are indicative of alterations in biogeochemical cycling and ecosystem functioning in the river.
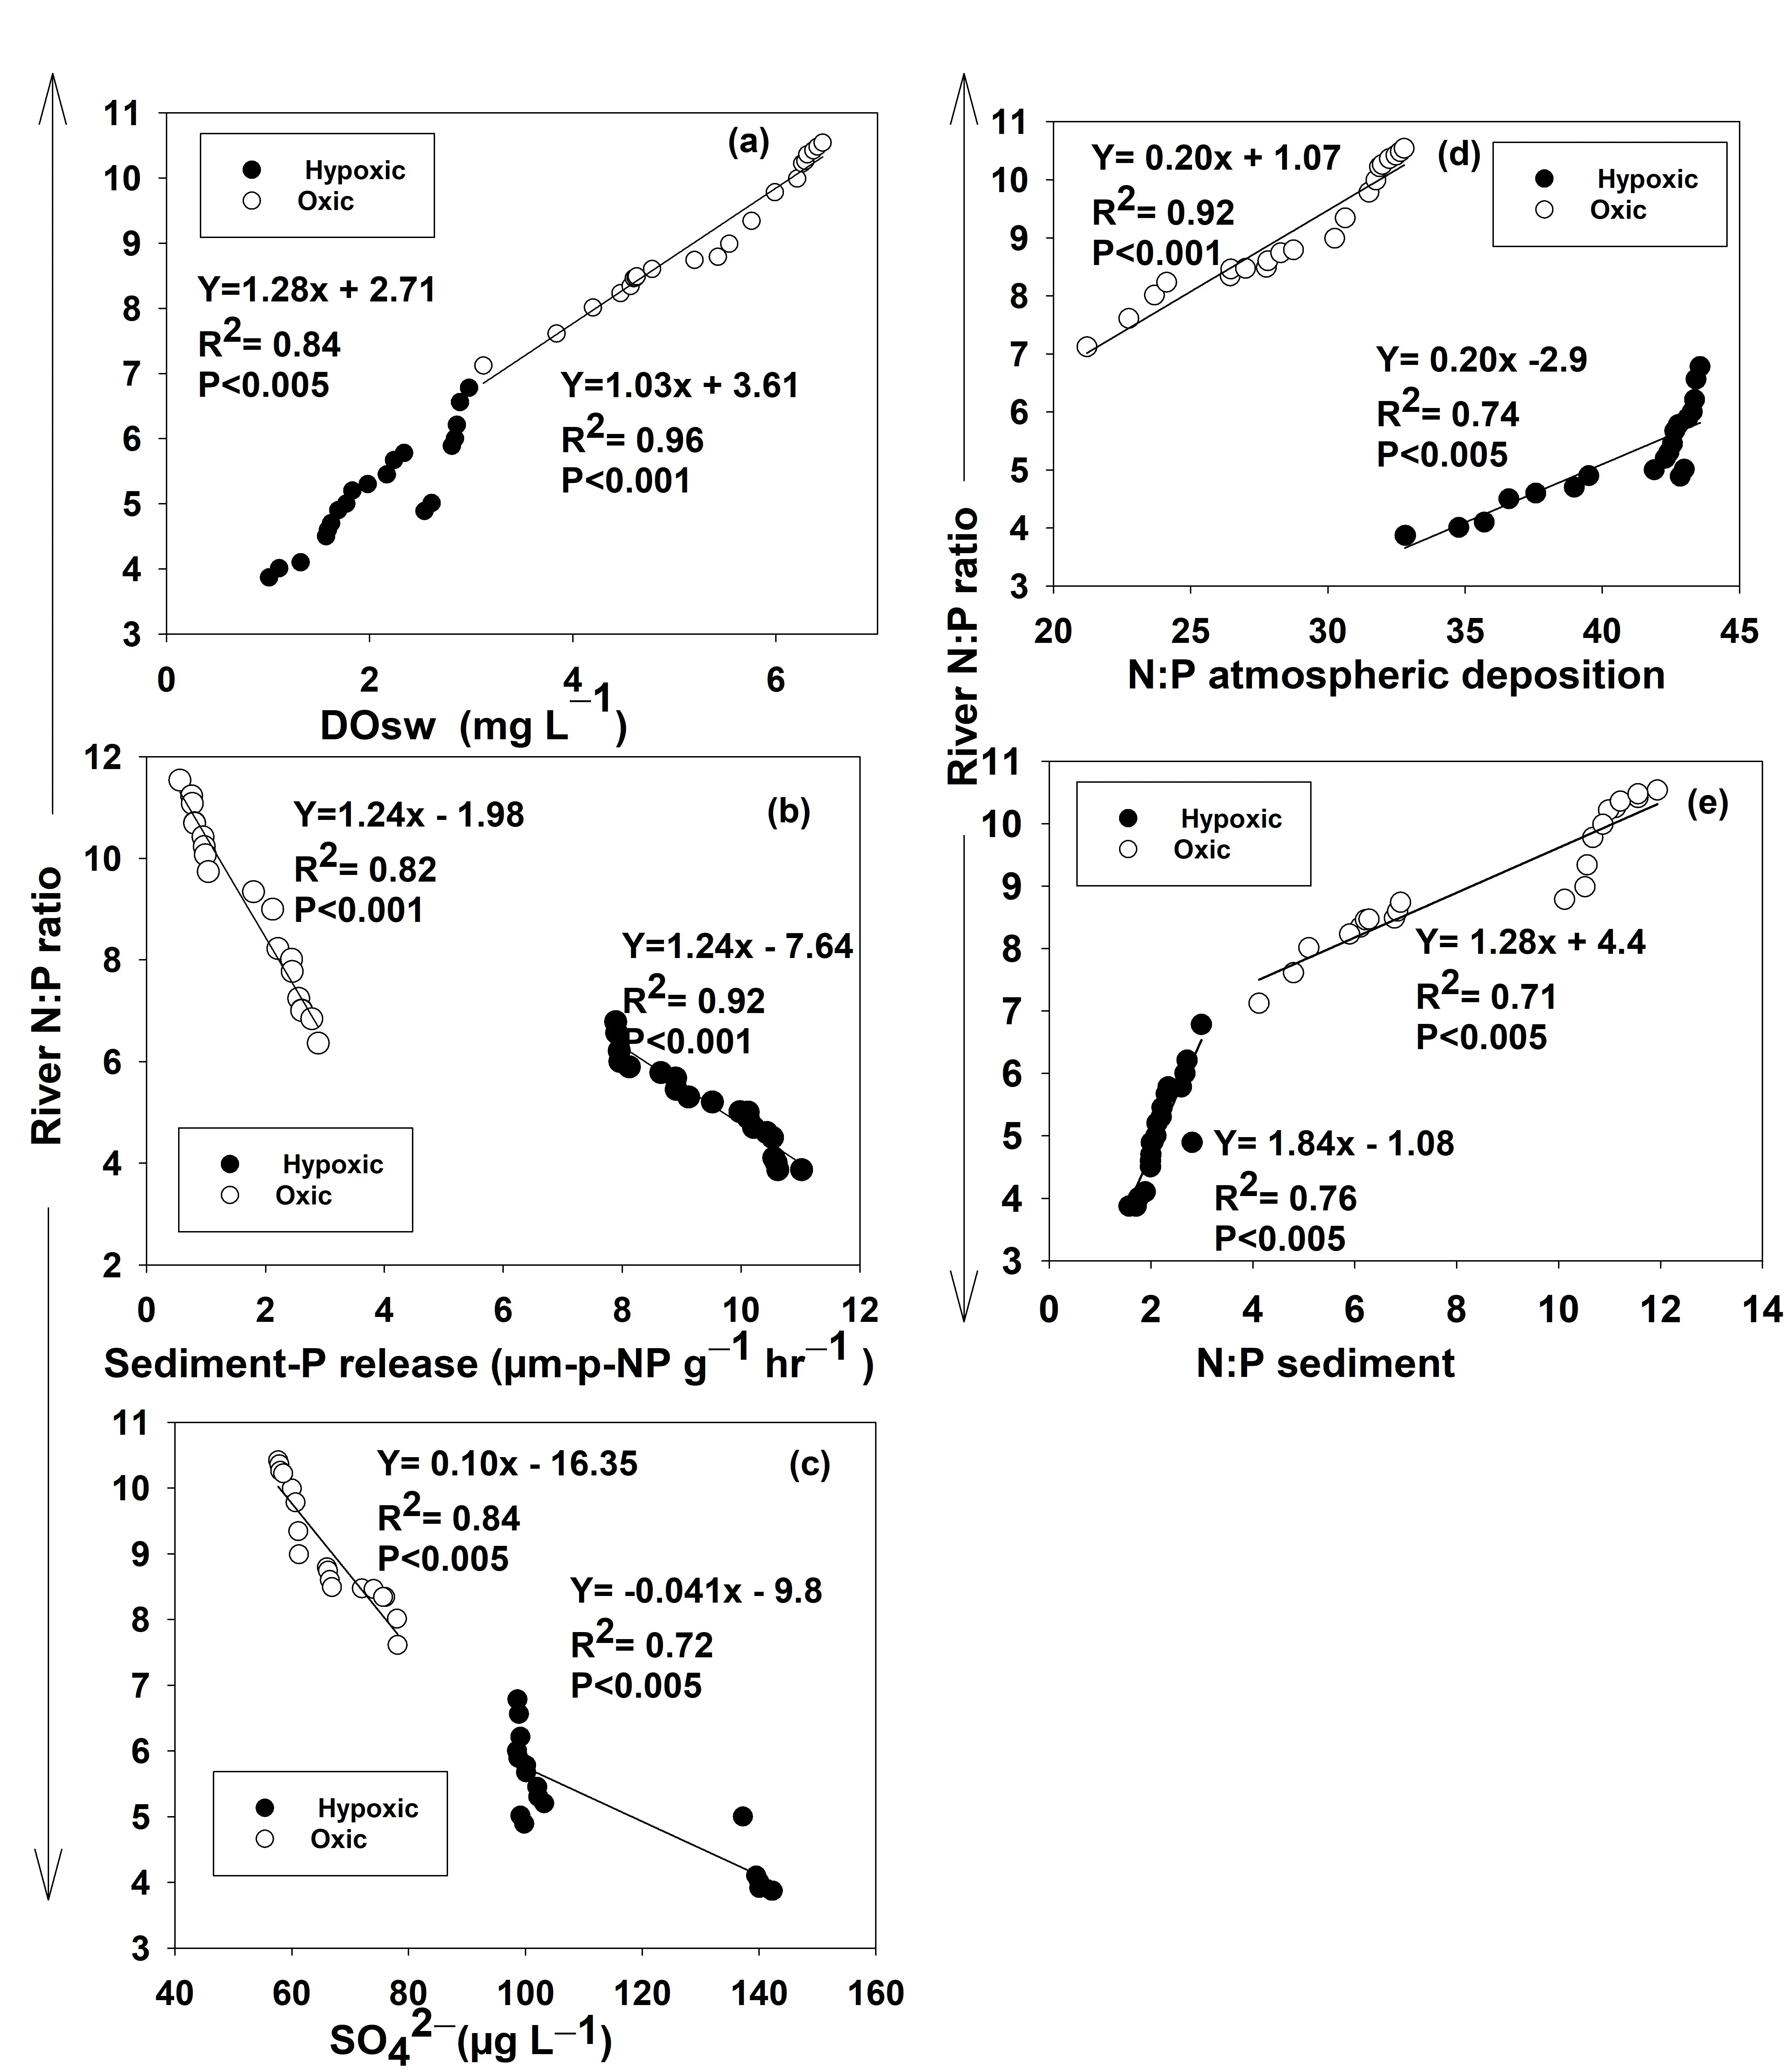
Figure 8. Scatter plot presenting significant correlations between: (a) DOsw and river N:P ratio, (b) sediment-P release and river N:P ratio, (c) SO42− and river N:P ratio, (d) N:P ratio of atmospheric deposition and river N:P ratio, and (e) N:P ratio of sediment and that of river at both hypoxic and oxic sites.
3.7. Statistical Validation
We assessed the relationships of nutrient stoichiometry with other determinants (Figure 8). The N:P ratios in river water were found to be strongly associated (R2 = 0.74–0.92; p < 0.005–0.001) with atmospheric N:P ratio. The river N:P ratios were found to be negatively associated with sediment-P release (R2 = 0.82–0.92; p < 0.001) as well as with the concentration of sulphate (R2 = 0.84; p < 0.001) (Figure 8). We tested the effects of site, year, temperature, and their interactions on major determinants of microbial processes and feedbacks (Table 2). The independent effects of site, year, and temperature have all been found highly significant (p < 0.001). However, the interactions of these determinants, except site × temperature (p < 0.001), did not appear significant. This indicates that despite the complexity of C substrate and microbial processing due to the presence of other stressors, riverine CO2 emission will remain sensitive to future climate warming.
Table 2. The F values obtained through multivariate analysis of variance (MANOVA; Wilks’ Lambda Test).
|
Determinants |
|||||||
|---|---|---|---|---|---|---|---|
|
Variables |
S |
Y |
T |
S × Y |
S × T |
T × Y |
S × Y × T |
|
NR |
153.91 * |
37.59 * |
17.17 * |
0.87 NS |
0.241 NS |
0.331 NS |
0.034 NS |
|
PO |
534.34 * |
43.56 * |
18.54 * |
1.5 NS |
0.049 NS |
0.20 NS |
0.033 NS |
|
MBC |
375.86 * |
79.76 * |
10.76 * |
1.36 NS |
0.034 NS |
0.056 NS |
0.021 NS |
|
CO2 |
787.88 * |
55.72 * |
26.41 * |
3.01 * |
0.128 NS |
0.116 NS |
0.034 NS |
|
SPR |
187.26 * |
39.24 * |
19.53 * |
0.63 NS |
0.197 NS |
0.291 NS |
0.036 NS |
S: site; Y: year; T: temperature; NR: nitrate reductase; PO: phenol oxidase; MBC: microbial biomass carbon; CO2: CO2 emission; SPR: sediment-P release. Independent effects of site, year, and temperature were found to be highly significant (p < 0.001) *. Interactions did not appear significant, except for Site × Temperature for CO2 emission. NS: not significant.
Principal component analysis (PCA) was used to elucidate mechanistic linkages between eutrophication, metal pollution, and extracellular enzyme activities. The PC1, which explained 76.54% of the total variance, shows the impacts of anthropogenic forcing segregating Jjmu, the most polluted site, far away and opposite to Shlktr, the least polluted site. The PC2, which explained 20.60% of the total variance, segregated alkaline phosphatase opposite to the concentration of phosphate as well as sediment-P release, a redox dependent process. The β-d-glucosidase appears segregated towards C rich sites such as Sngm and Rjht, although relatively away from the phenol oxidase, indicating that the former is more sensitive to metal pollutants compared to the latter. The negative relationship between β-d-glucosidase and metal pollutants alter a certain threshold indicates the sensitivity of carbon mineralization along metal pollution gradient. Phenol oxidase remained relatively closer to nutrients, metals, and C-eutrophication variables, indicating selective sensitivity and resilience of microbial enzymatic processes. Variables of eutrophication, such as chlorophyll a and gross primary productivity, showed relative synchrony with carbon and nutrients. Overall, eutrophication and metal stress in the Ganga River influenced microbial processes, shifting in carbon degradation and thereby reinforcing the positive feedbacks.
The activity of β-d-glucosidase increased initially, but after reaching a certain threshold, it declined sharply with increasing concentrations of metal pollutants. The phenol oxidase activity exhibited a partial mismatch. When regressed against the concentration of total heavy metal (THM), both β-d-glucosidase (R2 = 0.80; p < 0.001) and phenol oxidase (R2 = 0.96; p < 0.001) showed a positive dependence (Figure 9), possibly connecting to a concurrent increase in organic substrates, and then declined after reaching to a certain threshold. However, for β-d-glucosidase, the threshold concentration appears smaller relative to those of phenol oxidase, indicating high sensitivity of the former. The β-d-glucosidase activity is used as a signature of C-acquisition [44], and a pronounced decline in the activity of this enzyme indicates suppression of carbon-degrading microbial processes and consequently the amount of CO2 release at metal polluted sites. These patterns suggest that, although some enzymes are relatively less sensitive to stressors such as metal pollutants, elevated concentrations of heavy metals suppress microbial extracellular enzyme activities and alter carbon metabolism in large rivers. This is relevant to the riverine carbon budget and the release of greenhouse gases.
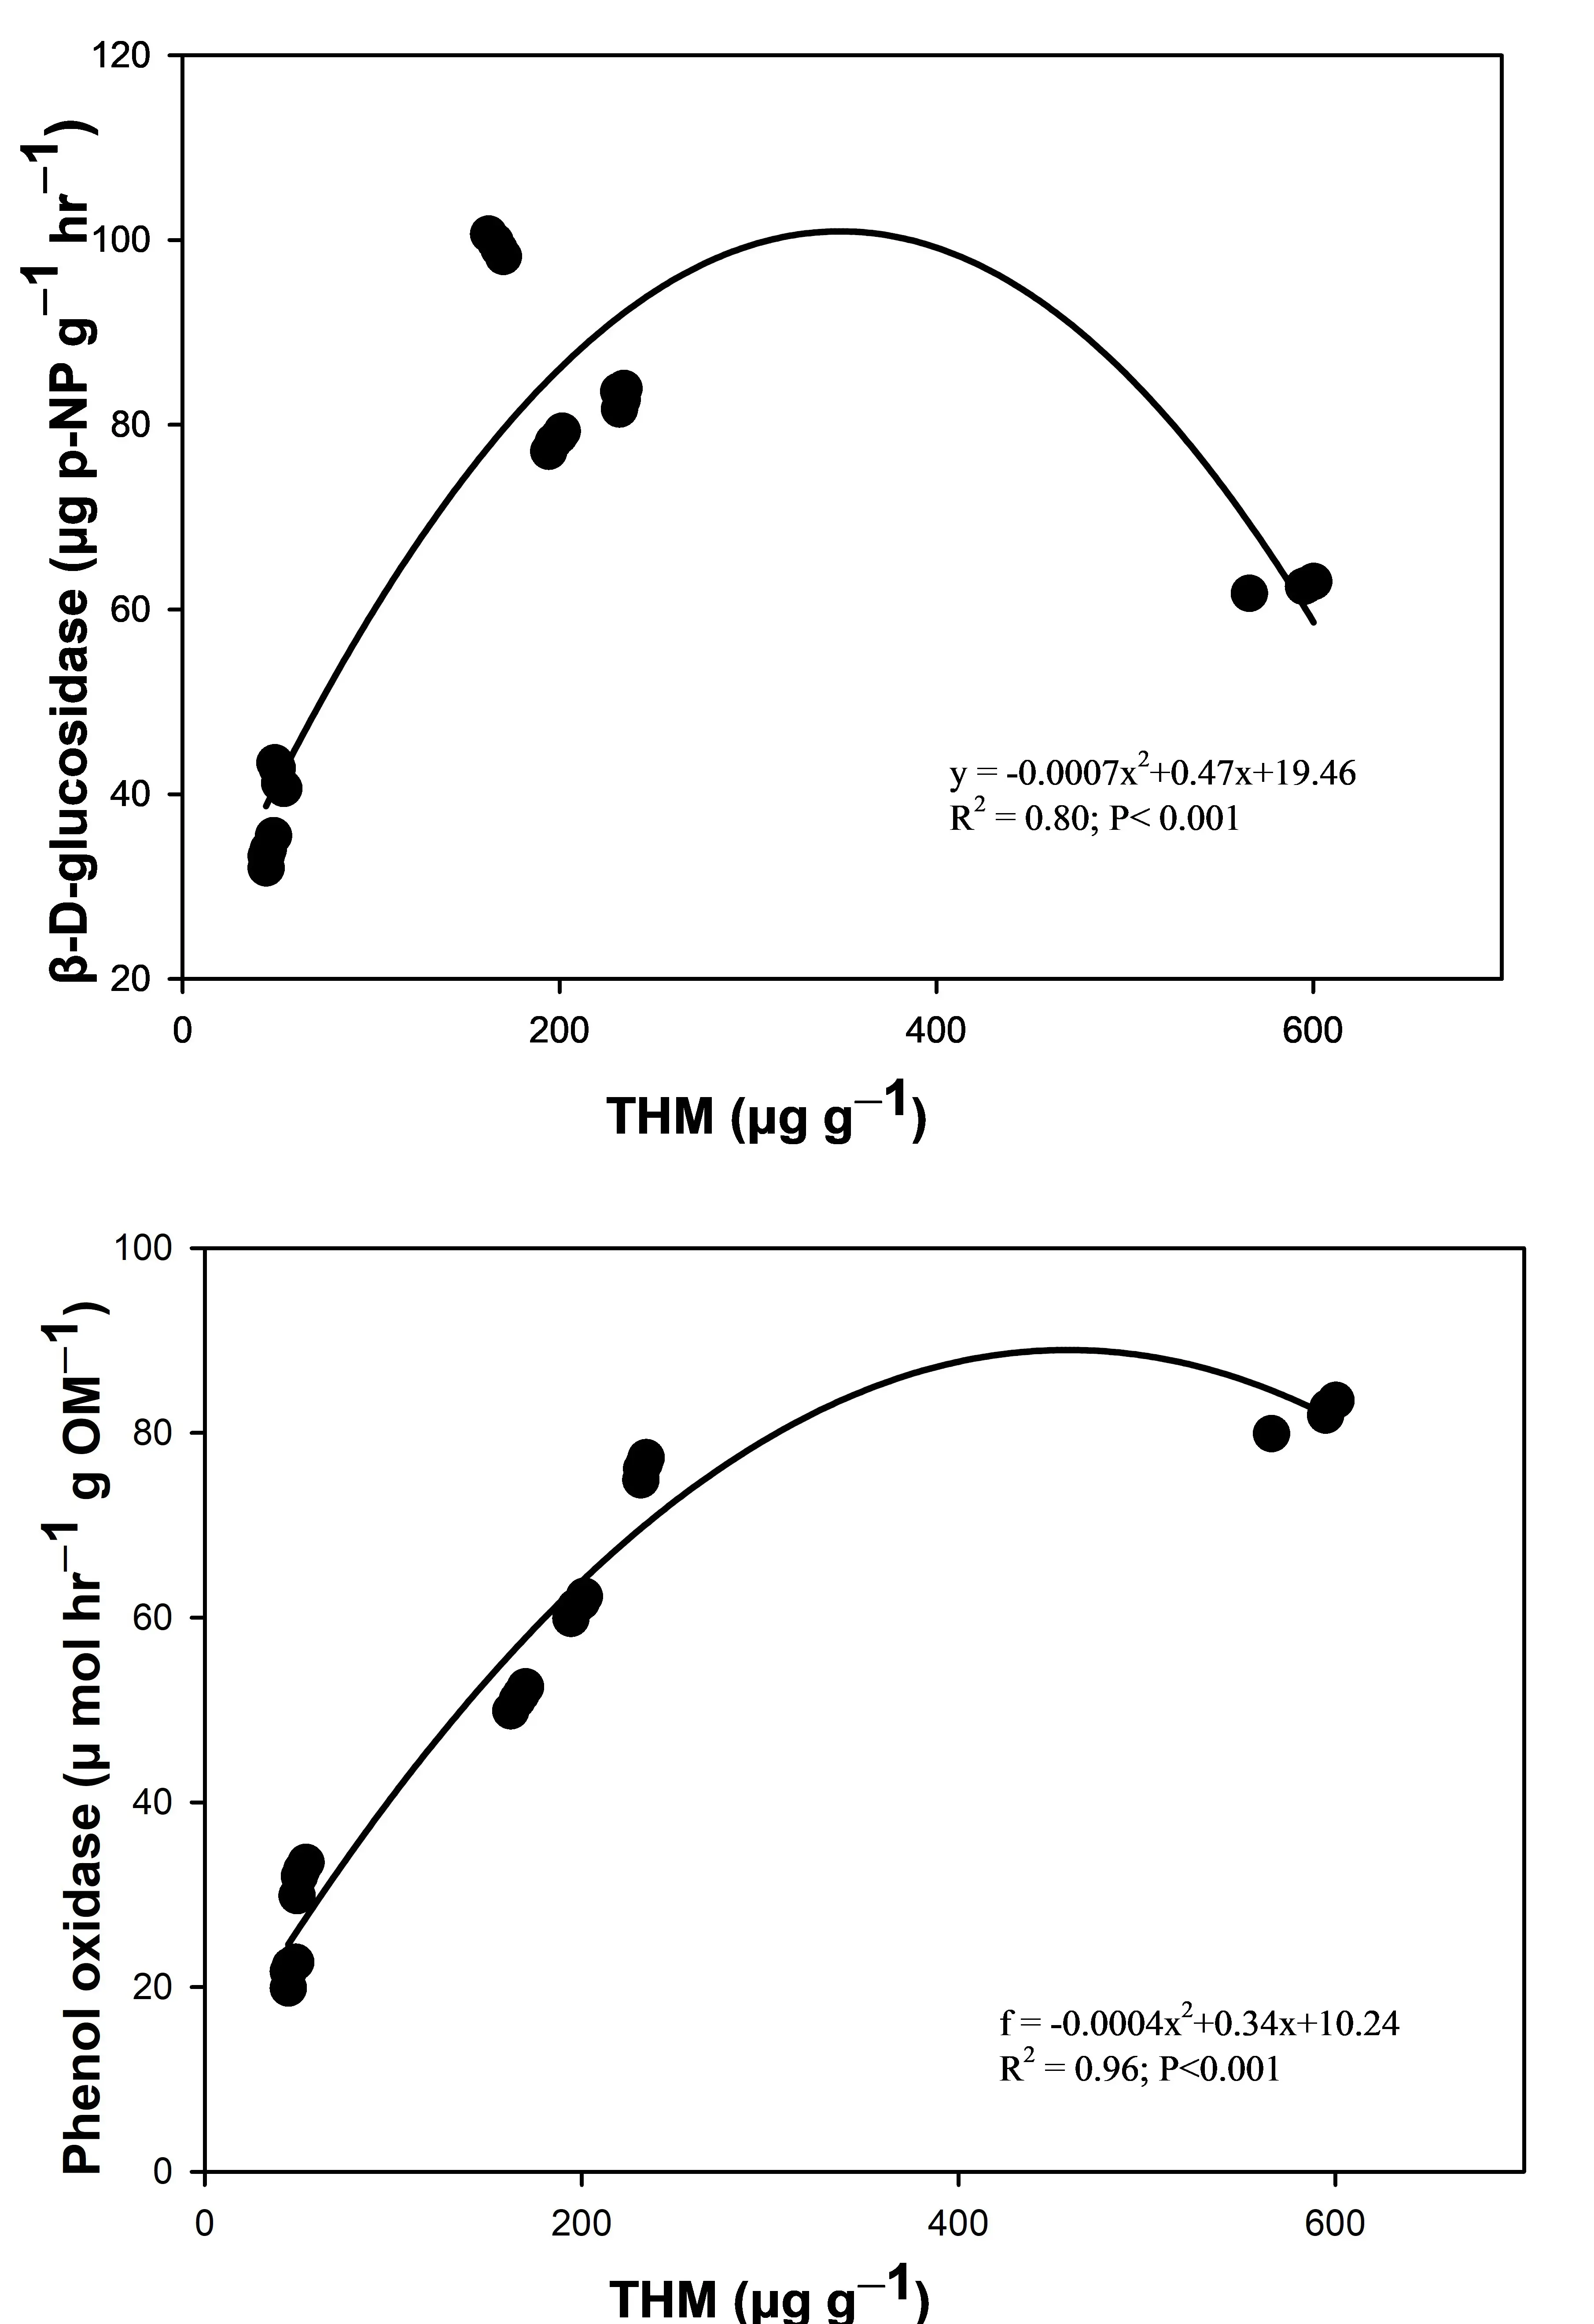
Figure 9. A dynamic fit regression model to test the relationships between total heavy metals (THM) and enzyme activities.
4. Conclusions
Our study concludes that although the severity of water quality degradation depends on the proportion of anthropogenic interventions, the overall changes result from how a river responds to those interventions through interconnected biogeochemical processes. Massive loading of carbon and nutrients and associated oxygen depletion strongly influence nutrient stoichiometry and microbial functioning in the middle stretch of the Ganga River. High concentrations of readily mineralizable carbon and recalcitrant carbon at polluted sites coupled with elevated CO2 flux, indicated a high rate of microbial respiration and organic matter turnover. Enhanced carbon degradation triggered increased microbial oxygen demand and reduced dissolved oxygen concentrations at the sediment-water interface, resulting in ecosystem feedbacks. Despite enhanced degradation, microbial biomass carbon declined by warming, indicating enhanced carbon loss relative to microbial biomass accumulation under climate warming. Such warming-enhanced shifts may progressively alter riverine productivity, microbial functioning, and overall watershed-scale biogeochemical stability. These findings suggest that human interventions, coupled with potential self-reinforcing biogeochemical feedbacks, likely trigger benthic niche transformation and consequently further degrade the river ecosystem. Moreover, the observed coupling among atmospheric deposition, organic carbon loading, and in-stream nutrient release/loss suggests that watershed-scale anthropogenic drivers alter riverine biogeochemical functioning and oxygen-sensitive nutrient cycling. The study emphasizes the importance of integrating climate warming, watershed-scale nutrient cycling, and riverine biogeochemical processes in future river management and climate impact assessment frameworks.
Supplementary Materials
The following supporting information can be found at: https://www.sciepublish.com/article/pii/1229, Figure S1: Spatio-temporal variations in the concentrations of nutrients and total organic carbon (TOC) in the Ganga River water; Figure S2: Spatio-temporal variations in the concentrations of metal pollutants in the Ganga River water; Figure S3: Spatio-temporal variations in: (a) Chl-a biomass, (b) gross primary productivity (GPP), (c) dissolved oxygen at sediment-water interface (DOsw), (d) Dissolved oxygen deficit at sediment-water interface, (e) SRP and (f) sediment-P release at study sites; Figure S4: Spatio-temporal trends in: (a) recalcitrant carbon, (b) readily mineralizable carbon, (c) CO2 emission and (d) microbial biomass C.
Acknowledgements
The authors are grateful to the Head, Department of Botany, Banaras Hindu University for the necessary facilities. The University Grant Commission (Grant No. 190520187517, 211610168097 and 240510225142 awarded to B.G., S.P. and A.V., respectively), New Delhi, and Institute of Eminence (Grant No. R/Dev/D/IoE/Incentive/2022–23/47664), Banaras Hindu University are gratefully acknowledged for the funding support.
Author Contributions
Methodology, B.G. and J.P.; Validation, J.P.; Formal analysis, B.G., S.P. and A.V.; Investigation, B.G., S.P., A.V. and J.P.; Data curation, B.G., S.P. and A.V.; Writing-original draft, B.G.; Funding acquisition, B.G., S.P., A.V. and J.P.; Conceptualization, J.P.; Writing-review and Editing, J.P.; Visualization, J.P.; Supervision, J.P.; Project administration, J.P.
Ethics Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The data can be made available on request.
Funding
This work was supported by University Grants Commission, India (Grant No. 190520187517, 211610168097 and 240510225142 awarded to B.G., S.P. and A.V. respectively) and IoE Banaras Hindu University (Grant No. R/Dev/D/IoE/Incentive/2022-23/47664)
Declaration of Competing Interest
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
References
- Elser JJ, Bracken MES, Cleland EE, Gruner DS, Harpole WS, Hillebrand H, et al. Global analysis of nitrogen and phosphorus limitation of primary producers in freshwater, marine and terrestrial ecosystems. Ecol. Lett. 2007, 10, 1135–1142. DOI:10.1111/j.1461-0248.2007.01113.x [Google Scholar]
- Schlenker C, Pinckney JL. Evaluating potential changes from nitrogen to phosphorus nutrient limitation of phytoplankton growth in north inlet estuary, SC. Estuaries Coasts 2025, 48, 137. DOI:10.1007/s12237-025-01565-6 [Google Scholar]
- Carpenter SR, Caraco NF, Correll DL, Howarth RW, Sharpley AN, Smith VH. Nonpoint pollution of surface waters with phosphorus and nitrogen. Ecol. Appl. 1998, 8, 559–568. DOI:10.2307/2641247 [Google Scholar]
- Galloway JN, Aber JD, Erisman JW, Seitzinger SP, Howarth RW, Cowling EB, et al. The nitrogen cascade. Bioscience 2003, 53, 341–356. DOI:10.1641/0006-3568(2003)053[0341:TNC]2.0.CO;2 [Google Scholar]
- Hecky RE, Kilham P. Nutrient limitation of phytoplankton in freshwater and marine environments: A review of recent evidence on the effects of enrichment. Limnol. Oceanogr. 1988, 33, 796–822. DOI:10.4319/lo.1988.33.4part2.0796 [Google Scholar]
- Elser JJ, Marzolf ER, Goldman CR. Phosphorus and nitrogen limitation of phytoplankton growth in the freshwaters of North America: A review and critique of experimental enrichments. Can. J. Fish Aquat. Sci. 1990, 47, 1468–1477. DOI:10.1139/f90-165 [Google Scholar]
- Chen N, Peng B, Hong H, Turyaheebwa N, Cui S, Mo X. Nutrient enrichment and N:P ratio decline in a coastal bay–river system in southeast China: The need for a dual nutrient (N and P) management strategy. Ocean Coast. Manag. 2013, 81, 7–13. DOI:10.1016/j.ocecoaman.2012.07.013 [Google Scholar]
- Wu K, Chen L, Wang Q, Li Y, Zheng Y, Ma Q, et al. Seasonal dynamics of nitrogen and phosphorus in wetland plants: Implications for efficient eutrophication control. Sustainability 2025, 17, 3443. DOI:10.3390/su17083443 [Google Scholar]
- Liu X, Li M, Chen J, Xu YJ, Zhang W, Chen Z, et al. Natural and reservoir-induced channel changes in the Yangtze River Tidal Reach. J. Hydrol. 2022, 605, 127398. DOI:10.1016/j.jhydrol.2021.127398 [Google Scholar]
- Jaiswal D, Naaz N, Gupta S, Madhav K, Pandey J. Diurnal oscillation in dissolved oxygen at sediment-water interface fuels denitrification-driven N removal in Ganga River. J. Hydrol. 2023, 619, 129301. DOI:10.1016/j.jhydrol.2023.129301 [Google Scholar]
- Welch EB, Cooke GD. Internal phosphorus loading in shallow lakes: Importance and control. Lake Reserv. Manag. 2005, 21, 209–217. DOI:10.1080/07438140509354430 [Google Scholar]
- Downing JA, McCauley E. The nitrogen: Phosphorus relationship in lakes. Limnol. Oceanogr. 1992, 37, 936–945. DOI:10.4319/lo.1992.37.5.0936 [Google Scholar]
- Houser JN, Richardson WB. Nitrogen and phosphorus in the Upper Mississippi River: Transport, processing, and effects on the river ecosystem. Hydrobiologia 2010, 640, 71–88. DOI:10.1007/s10750-009-0067-4 [Google Scholar]
- Conley DJ, Paerl HW, Howarth RW, Boesch DF, Seitzinger SP, Havens KE, et al. Controlling eutrophication: Nitrogen and phosphorus. Science 2009, 323, 1014–1015. DOI:10.1126/science.1167755 [Google Scholar]
- Lønborg C, Álvarez–Salgado XA, Letscher RT, Hansell DA. Large stimulation of recalcitrant dissolved organic carbon degradation by increasing ocean temperatures. Front. Mar. Sci. 2018, 4, 436. DOI:10.3389/fmars.2017.00436 [Google Scholar]
- Caraco NF, Cole JJ, Likens GE. Sulfate control of phosphorus availability in lakes. Hydrobiologia 1993, 253, 275–280. DOI:10.1007/BF00050748 [Google Scholar]
- Søndergaard M, Jensen JP, Jeppesen E. Role of sediment and internal loading of phosphorus in shallow lakes. Hydrobiologia 2003, 506, 135–145. DOI:10.1023/B:HYDR.0000008611.12704.dd [Google Scholar]
- Peñuelas J, Poulter B, Sardans J, Ciais P, Van der Velde M, Bopp L, et al. Human-induced nitrogen–phosphorus imbalances alter natural and managed ecosystems across the globe. Nat. Commun. 2013, 4, 2934. DOI:10.1038/ncomms3934 [Google Scholar]
- Diaz RJ, Rosenberg R. Spreading dead zones and consequences for marine ecosystems. Science 2008, 321, 926–929. DOI:10.1126/science.1156401 [Google Scholar]
- Paerl HW, Paul VJ. Climate change: Links to global expansion of harmful cyanobacteria. Water Res. 2012, 46, 1349–1363. DOI:10.1016/j.watres.2011.08.002 [Google Scholar]
- Jaiswal D, Pandey U, Mishra V, Pandey J. Integrating resilience with functional ecosystem measures: A novel paradigm for management decisions under multiple-stressor interplay in freshwater ecosystems. Glob. Change Biol. 2021, 27, 3699–3717. DOI:10.1111/gcb.15662 [Google Scholar]
- Central Pollution Control Board (CPCB). Pollution Assessment: River Ganga; Ministry of Environment and Forests, Government of India: New Delhi, India, 2013. [Google Scholar]
- American Public Health Association. Standard Methods for the Examination of Water and Wastewater, 20th ed.; APHA: Washington, DC, USA, 1998; pp. 1–1193. [Google Scholar]
- Sánchez E, Colmenarejo MF, Vicente J, Rubio A, García MG, Travieso L, et al. Use of the water quality index and dissolved oxygen deficit as simple indicators of watersheds pollution. Ecol. Indic. 2007, 7, 315–328. DOI:10.1016/j.ecolind.2006.02.005 [Google Scholar]
- Vogel AI. A Text Book of Quantitative Inorganic Analysis, 4th ed.; ELBS and Longman: London, UK, 1971. [Google Scholar]
- Tan KH. Soil Sampling, Preparation, and Analysis, 2nd ed.; CRC Press: Boca Raton, FL, USA, 2005; pp. 255–257. [Google Scholar]
- Park GE, Oh HN, Ahn S. Improvement of the ammonia analysis by the phenate method in water and wastewater. Bull. Korean Chem. Soc. 2009, 30, 2032–2038. DOI:10.5012/bkcs.2009.30.9.2032 [Google Scholar]
- Chen L, Flynn DFB, Jing X, Kühn P, Scholten T, He JS. A comparison of two methods for quantifying soil organic carbon of alpine grasslands on the Tibetan Plateau. PLoS ONE 2015, 10, e0126372. DOI:10.1371/journal.pone.0126372 [Google Scholar]
- Murphy J, Riley JP. A modified single solution method for the determination of phosphate in natural waters. Anal. Chim. Acta. 1962, 27, 31–36. DOI:10.1016/S0003-2670(00)88444-5 [Google Scholar]
- Lorenzen CJ, Jeffrey SW. Determination of Chlorophyll in Seawater; Report of intercalibration tests, in UNESCO Technical Papers in Marine Science; UNESCO: Paris, France, 1980. [Google Scholar]
- Hu WF, Lo W, Chua H, Sin SN, Yu PHF. Nutrient release and sediment oxygen demand in a eutrophic land-locked embayment in Hong Kong. Environ. Int. 2001, 26, 369–375. DOI:10.1016/S0160-4120(01)00014-9 [Google Scholar]
- Jenkinson DS, Powlson DS. The effects of biocidal treatments on metabolism in soil—V: A method for measuring soil biomass. Soil Biol. Biochem. 1976, 8, 209–213. DOI:10.1016/0038-0717(76)90005-5 [Google Scholar]
- Sinsabaugh RL, Findlay S. Microbial production, enzyme activity, and carbon turnover in surface sediments of the Hudson River estuary. Microb. Ecol. 1995, 30, 127–141. DOI:10.1007/BF00172569 [Google Scholar]
- Tabatabai MA, Bremner JM. Use of p-nitrophenyl phosphate for assay of soil phosphatase activity. Soil Biol. Biochem. 1969, 1, 301–307. DOI:10.1016/0038-0717(69)90012-1 [Google Scholar]
- Eivazi F, Tabatabai MA. Glucosidases and galactosidases in soils. Soil Biol. Biochem. 1988, 20, 601–606. DOI:10.1016/0038-0717(88)90141-1 [Google Scholar]
- Reddy KR, D’Angelo EM. Biogeochemical indicators to evaluate pollutant removal efficiency in constructed wetlands. Water Sci. Technol. 1997, 35, 1–10. DOI:10.1016/S0273-1223(97)00046-2 [Google Scholar]
- Gillet RW, Ayers GP. The use of thymol as a biocide in rain water samples. Atmos. Environ. Part A 1991, 25, 2677–2681. DOI:10.1016/0960-1686(91)90198-G [Google Scholar]
- Sen A, Abdelmaksoud AS, Ahammed YN, Alghamdi MA, Banerjee T, Bhat MA, et al. Variations in particulate matter over Indo-Gangetic Plains and Indo-Himalayan Range during four field campaigns in winter monsoon and summer monsoon: Role of pollution pathways. Atmos. Environ. 2017, 154, 200–224. DOI:10.1016/j.atmosenv.2016.12.054 [Google Scholar]
- Sayer AM, Munchak LA, Hsu NC, Levy RC, Bettenhausen C, Jeong MJ. MODIS Collection 6 aerosol products: Comparison between Aqua’s e-Deep Blue, Dark Target, and “merged” data sets, and usage recommendations. J. Geophys. Res. Atmos. 2014, 119, 13965–13989. DOI:10.1002/2014JD022453 [Google Scholar]
- Singh R, Pandey J. Non-point source-driven carbon and nutrient loading to Ganga River (India). Chem. Ecol. 2019, 35, 344–360. DOI:10.1080/02757540.2018.1554061 [Google Scholar]
- Siddiqui E, Pandey J, Pandey U, Mishra V, Singh AV. Integrating atmospheric deposition-driven nutrients (N and P), microbial and biogeochemical processes in the watershed with carbon and nutrient export to the Ganga River. Biogeochemistry 2020, 147, 149–178. DOI:10.1007/s10533-019-00634-w [Google Scholar]
- Pandey U, Pandey J. Impact of DOC trends resulting from changing climatic extremes and atmospheric deposition chemistry on periphyton community of a freshwater tropical lake of India. Biogeochemistry 2013, 112, 537–553. DOI:10.1007/s10533-012-9747-7 [Google Scholar]
- Jaiswal D, Pandey J. An ecological response index for simultaneous prediction of eutrophication and metal pollution in large rivers. Water Res. 2019, 161, 423–438. DOI:10.1016/j.watres.2019.06.030 [Google Scholar]
- Jaiswal D, Pandey J. Carbon dioxide emission coupled extracellular enzyme activity at land-water interface predict C-eutrophication and heavy metal contamination in Ganga River, India. Ecol. Indic. 2019, 99, 349–364. DOI:10.1016/j.ecolind.2018.12.046 [Google Scholar]
- Li H, Cai Y, Song C, Cao Z, Li J, Qin Z, et al. Comparison of phosphorus migration and transformation characteristics in sediments of lakes within the Yangtze River basin and reservoirs on the Wujiang River. J. Soils Sediments 2024, 24, 991–1001. DOI:10.1007/s11368-023-03698-2 [Google Scholar]
- Yang Y, Duan X, Liang S, Zhang M, Li S, Li H, et al. Role of phosphorus concentration and the nitrogen to phosphate ratio in the synergistic stimulation of alkaline phosphatase activity in Laizhou Bay, China, coastal waters. Biogeoscience 2025, 23, 1609–1623. DOI:10.5194/bg-23-1609-2026 [Google Scholar]
- Sinsabaugh RL. Phenol oxidase, peroxidase and organic matter dynamics of soil. Soil Biol. Biochem. 2010, 42, 391–404. DOI:10.1016/j.soilbio.2009.10.014 [Google Scholar]
- De Klein JJM, Overbeek CC, Jørgensen CJ, Veraart AJ. Effect of temperature on oxygen profiles and denitrification rates in freshwater sediments. Wetlands 2017, 37, 975–983. DOI:10.1007/s13157-017-0933-1 [Google Scholar]
- Ribalet F, Dutkiewicz S, Monier E, Armbrust EV. Future ocean warming may cause large reductions in Prochlorococcus biomass and productivity. Nat. Microbiol. 2025, 10, 2441–2453. DOI:10.1038/s41564-025-02106-4 [Google Scholar]
- Thomas SC, Tamadonfar KO, Seymour CO, Lai D, Dodsworth JA, Murugapiran SK, et al. Position-specific metabolic probing and metagenomics of microbial communities reveal conserved central carbon metabolic network activities at high temperatures. Front. Microbiol. 2019, 10, 1427. DOI:10.3389/fmicb.2019.01427 [Google Scholar]
- Song Y, Li M, Liu X, Li W, Yao H, Liu Y, et al. Effects of riverine nutrient enrichment and sediment reduction on high primary productivity zone in the Yangtze River estuary: Historical reconstruction and future perspective. Front. Mar. Sci. 2025, 12, 1529744. DOI:10.3389/fmars.2025.1529744 [Google Scholar]
- Gupta B, Pandey S, Pandey J. High concentration of sulfate coupled with climate warming generates ecosystem feedback under sub-oxic conditions at sediment-water interface in the Ganga River. Bull. Environ. Contam. Toxicol. 2023, 111, 40. DOI:10.1007/s00128-023-03790-w [Google Scholar]
- Wang P, Xing X, Wang X, Hu B. Spatial distribution and coupling of carbon, nitrogen, phosphorus, and sulfur functional genes in a highly dam-regulated international river. Environ. Res. 2025, 287, 122988. DOI:10.1016/j.envres.2025.122988 [Google Scholar]