Blastospores of Entomopathogenic Fungi Emerge as the Promising Active Ingredients in Biocontrol Agents: Progressive View on Its Industrial Production and Biogenesis Mechanisms
Blastospores of Entomopathogenic Fungi Emerge as the Promising Active Ingredients in Biocontrol Agents: Progressive View on Its Industrial Production and Biogenesis Mechanisms
Received: 29 July 2026 Revised: 12 August 2026 Accepted: 21 August 2026 Published: 28 August 2026

© 2026 The authors. This is an open access article under the Creative Commons Attribution 4.0 International License (https://creativecommons.org/licenses/by/4.0/).
1. Introduction
Fungal entomopathogens represent a large group of filamentous fungi that infect a plethora of arthropods in natural eco-system and have great potential in pest management programs as biocontrol reagents [1]. The host infection caused by entomopathogenic fungi (EPF) features the direct penetration of the exoskeleton by infectious hypha developing from conidia that adhere to the host cuticle [2]. After invading the host body cavity, filamentous cells develop into the single thin-walled yeast-like blastospores via dimorphic transition for rapid proliferation by efficiently assimilation of various nutrients in the host hemocoel, which ultimately causes the host’s death. Therefore, the fungus’s ability to perform dimorphism is essential for the pathogen colonization and virulence [3]. In addition to being in the hemocoel, blastospores can also be produced in submerged liquid cultivation and have great potential as the main active ingredient in practical formulations [4]. The advantages of submerged fermentation (SMF) over solid-state fermentation (SSF) mainly involve better compatibility with industrial production equipment, easier control of the whole process, and simpler procedure for product recovery [5]. In comparison with aerial conidia produced via SSF [6], the SmF-produced blastospores are more hydrophilic and virulent [7,8,9,10]. In addition, SmF for blastospore production exhibits higher productive efficiency because it takes less time and space than conidiation in SSF [11,12,13]. Thus, SmF has been attracting more and more attention in production of EPF infectious cells such as Beauveria bassiana, Metarhizium anisopliae, and Isaria (formerly Paecilomyces) fumosoroseus [14,15], and blastospores were developed into biological control agents for field application (Figure 1). Here, we provide an overview of the mechanisms underlying blastospore biogenesis and technological advances in fermentation bioprocess, which will enable researchers to explore suitable parameters and tools for a productive and efficient production of blastospores.
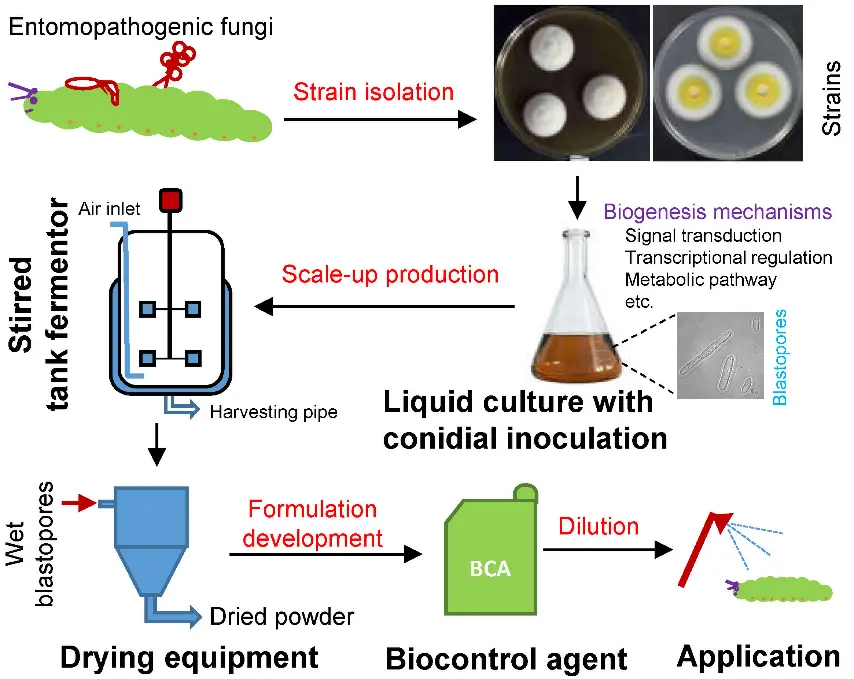
Figure 1. General procedure for developing mycoinsecticides with blastospores of entomopathogenic fungi.
2. Technologies for Blastospore Production
Commercial use of fungal biocontrol agents is highly dependent on the low-cost production of infectious propagula. To efficiently produce blastospores with high activity, a plethora of physicochemical factors are recognized and utilized to optimize fermentation process control.
2.1. Nutritional Components in Medium
The carbon (C) and nitrogen (N) sources have been considered as important factors influencing fungal blastospore yield, and their concentrations should be optimized according to fungal species and isolates (Supplementary Table S1). Kleespies and Zimmermann (1992) tested the effects of various carbohydrates and corn-steep products (nitrogen source) on blastospore yield in three strains of M. anisopliae and found that the blastospore yields of the tested strains displayed different responses to nutrient types [16]. In general, preferred carbohydrates are glucose and fructose; however, different corn steep brands yield different blastospore yields. M. flavoviride (IMI 330189) displays the maximal production on sucrose and yeast extract with a C/N ratio of 1.6 [17]. However, M. anisopliae (EAMa 01/58-Su) produces high blastospore concentration on different C/N ratios, which is dependent on the types of carbon and nitrogen sources. This strain produced the greatest amount of blastospores in a broth consisting of glucose (30 g/L) and peptone (30 g/L) at a C/N ratio of 10.66. [18]. Glucose-enriched cultures (140 g glucose/L) improve blastospore yield of M. robertsii ESALQ1426 under optimal growth conditions, with production as high as 5.9 × 10⁸ blastospores/mL within 2 days [19]. B. bassiana and I. fumosorosea produce higher blastospore concentrations in media containing cottonseed flour as a nitrogen source than acid hydrolyzed casein [11]. Combinational nitrogen source of corn steep powder and yeast extract (YE) gives M. anisopliae 416.96 a higher blastospore yield than the combination of cottonseed flour and YE [20]. Cliquet and Jackson (1999) tested the effects of thirteen amino acids on blastospore yield of Isaria (formerly Paecilomyces) fumosoroseus (Mycotech strain 612) and found that glutamate, aspartate, and glycine resulted in higher blastospore yields (6.6–11.0 × 10⁸ blastospores/mL) than the nitrogen source of casamino acids (6.0 × 10⁸ blastospores/mL) [21]. When sucrose is used as a carbon source, the B. bassiana GHA strain prefers corn steep liquor as a nitrogen source to casaminoacids or peptone in blastospore production [22]. As for B. bassiana KK5, an optimized nutrient complex with plant substrates results in a maximum spore concentration of 8.5 × 10⁸/mL which is approximately 3 times that of pre-optimized nutrient [23]. M. flavoviride (IMI 330189) displays different blastospore productions in various synthetic and semi-synthetic broths, with higher concentrations of blastospores in richer media [24]. When using a high casamino acid concentration, the blastospore yield for Isaria (formerly Paecilomyces) fumosoroseus strain Mycotech 612 is significantly higher when compared to that in medium containing a lower casamino acid concentration [25].
In addition to carbon and nitrogen sources, nutritional additives have attracted more attention due to their important roles in blastospore production. When producing the blastospores of M. anisopliae var. anisopliae strain 97, its yield was significantly increased by the addition of 5% lecithin (10 fold), 3% collagen (3.7 fold), and 1.5% lactic acid (2 fold) compared to that in the standard medium [26]. Zinc ion is required for fungal growth and blastospore production of Isaria (formerly Paecilomyces) fumosoroseus (Mycotech strain 612); however, addition of vitamins does not result in a significant change in blastospore yield [21]. When producing the blastospores of Cordyceps javanica IF-1106, the maximum sporulation yield is obtained by the addition of an optimal complex of metal ions containing Mn2+, Cu2+, Fe2+, and Fe3+ [27]. As for Akanthomyces attenuatus JEF-147, magnesium sulfate (1%) significantly increases the blastospore production in a glucose-based liquid culture [28].
Entomopathogenic fungi exhibit diversified patterns for blastospore biogenesis [29]. Fungal strains of the same genus and species can behave differently in response to various nutritional components in culture media. These findings suggest that various nutrients have great potential for regulating blastospore production, but most of the information provided cannot be extrapolated to all strains within the genus and species. Therefore, when producing blastospores on a large scale, suitable strain-specific nutrients must be evaluated to achieve maximal productivity.
2.2. Fermentation Processes
Blastospores are produced in liquid culture fermentation, either in shake flasks or in deep-tank bioreactors for different scales of production [30]. Initial inoculation size has an important influence on blastospore production rate. As for Isaria (formerly Paecilomyces) strain 612, when blastospores are used as initial inocula, and a blastospore concentration of 106 spores/mL results in maximum concentrations of blastospores within 2 days. However, the concentration of 105 spores/mL causes one-day delay in presence of maximum yield [31]. Physicochemical properties of liquid medium have a great influence on optimal blastospore production, in which pH value and water availability (aw) of liquid media are considered as prior physicochemical factors. To obtain maximum blastospore yield of M. anisopliae (strain 416.96), the pH of the liquid medium is controlled at 6.8–8.0, and polyethylene glycol (molecular weight 200) (PEG 200) is used as the aw-modifying agent [20]. Similarly, PEG 200 greatly suppresses the generation of mycelial pellet and increases blastospore yield of M. anisopliae and B. bassiana [26,32]. In addition, PEG 200 decreases the blastospore size of B. bassiana [32]. However, M. anisopliae strains display different optimal pH for blastospore production [16]. Adoption of low-pH (pH 4) medium and relatively large initial inoculation size results in very low levels of bacterial contamination [30]. Téllez-Martínez et al. (2016) scaled up fermentation production of M. acridum blastospores in a stirred tank bioreactor with optimal nutrients and production parameters (constant stirring at 635 rpm, a temperature of 26 °C, and pH 3.3), which resulted in a yield of 1.25 × 10⁸ blastospores/mL [33].
The dissolved oxygen level is critical for blastospore formation under the submerged conditions [34]. Dissolved oxygen > 40% is beneficial for blastospore production by M. anisopliae strain MaQ01 [8]. The maximum blastospore yield of M. flavoviride Mf189 was obtained with pH and pO2 regulated to 7 and 100%, respectively [17]. Adequate dissolved oxygen levels combined with high glucose concentrations enhanced the blastospore yield of B. bassiana [35]. To increase dissolved oxygen level, constant agitation and aeration are explored in blastospore production of Isaria (formerly Paecilomyces) (strain 612) [22,36]. In the 6-L bioreactor, the filtered atmospheric air is initially pumped into B. bassiana culture at 1.5 L/min, and the dissolved oxygen level is maintained above 10% in the subsequent cultivation stage [13]. These findings suggest that fungal strains require different optimal physicochemical conditions, which must be optimized in the fermentation process. Particularly, the physiological and genetic bases for blastospore formation under various physicochemical conditions remain largely unknown, which deserves further investigation.
2.3. Harvesting, Drying, and Storage Technologies
Blastospores are produced in a liquid environment and must be harvested and dried for further formulation process. Usually, blastospores are harvested via centrifugation and filtration [23]. Isotonic solutions (e.g., PEG 200) are suitable for washing the harvested blastospores to increase the spore viability [37]. In application-oriented process design, the harvesting process is connected to the drying process. During blastospore production of B. bassiana and I. fumosorosea, the resultant culture is mixed with diatomaceous earth and vacuum-filtered. The resulting filter cake is ground and dried in an air drying chamber under a programed relative humidity [11,38,39]. In addition to diatomaceous earth, other powder are also used as support matrix in air drying of blastospores, including silica gel, sand, calcined kaolin clay, talc powder, and the like [40,41]. In blastospore production of Cordyceps species, liquid cultures are dried using a spray dryer equipped with a spinning disk atomizer. The parameters for spray drying are set as follows: inlet temperature at ~85 °C, outlet temperature at ~50 °C, and 5.7 bar at wheel atomizer [12]. Spray drying of blastospore with the addition of ascorbic acid improves product stability during storage [42]. The vacuum freeze-drying method is also used to dry EPF blastospores (e.g., Isaria (formerly Paecilomyces) ARSEF 4491 and Mycotech strain 612). Typically, the harvested blastospores are freeze dried in a lyophilizer with a eutectic-automatic program [21,43]. The rotary vacuum drum dryer is used to dry fungal biomass (e.g., blastospores) mixed with inert carrier (e.g., diatomaceous earth) and other additives to prepare a formulation [15]. Therefore, it is recommended to dry fungal biomass under vacuum conditions, which increases drying efficacy and fungal viability.
Dried blastospores are sealed in polypropylene plastic packages on vacuum-packaging machine and stored at a conventional refrigerator at 4 °C [4]. After a storage of 5 months at 4 °C, the survival rate for the lyophilized Isaria (formerly Paecilomyces) (strain ARSEF 4491) blastospores still exceeds 65%, and less than 25% of the air-dried blastospores are viable after 90-d storage. When stored at 22 °C, the lyophilized blastospores lose most viability within 30 d, none of the air-dried blastospores are alive [43]. When producing another Isaria (formerly Paecilomyces) (ARSEF 3581), the addition of proteinous substrates (e.g., whole milk) to starch-oil formulations significantly improves the storage stability of freeze-dried blastospores at 4 °C [44]. This indicates that further investigations are required to optimize the drying method and improve the storage stability of blastospores.
2.4. Formulation of Blastospores
As summarized in Table 1, a list of entomopathogenic fungi has been developed into blastospore-based formulations to control various arthropods. Blastospores are easily formulated into water or Tween solution due to their hydrophilic surface [7]. In many occasions, this type of formulation is only suitable for laboratory work (e.g., virulence test). Bead formulation is an emerging one, when compared with the traditional types (e.g., wettable powder and emulsifiable oil), but it could be considered as a variant of granule formulation. Obviously, given the physical states of existing formulations, the room for designing a new formulation type is rather limited. Kaiser et al., (2020) used a single substance or co-formulation of B. bassiana blastospore to control pollen beetles. For co-formulation, B. bassiana blastospores were combined with colza oil containing 2% surfactant. Single use of blastospores resulted in the mortality of 20%, and the co-formulation led to the mortality beyond 60%, which indicates a strong synergistic effect between blastospore and vegetable oil [45]. The air-dried blastospores of B. bassiana cultured on corn steep liquor are formulated with diatomaceous earth, and the formulation remains virulent against three-instar larvae of Plutella xylostella after 6-month storage at 4 °C [22]. Thus, many more investigations are needed to test different types of substrates and optimize the formula to improve blastospore stability. Blastospores are generally considered more virulent than conidia as they generate germ tubes and penetrate the host cuticle at a faster rate. However, the blastospores of M. brunneum ARSEF 4556 are less virulent against Culex quinquefasciatus larvae than conidia due to the lower adhesion rate of blastospores [46]. This indicates that the interaction of blastospores with the host cuticle must be seriously considered in designing the formula of the blastospore-based mycoinsecticides.
Table 1. Blastospore-based biocontrol formulations and their target hosts.
|
Fungal Species |
Formulation Type |
Addictive(s) |
Target Host(s) |
References |
|---|---|---|---|---|
|
Akanthomyces attenuatus JEF-147 |
Suspended in 0.03% siloxane solution, when use |
Tetranychus urticae |
[28] |
|
|
Akanthomyces dipterigenus CG829 |
Suspended in 0.05% Tween-80 solution, when use |
Bemisia tabaci, Aphis fabae, Planococcus sp. |
[47] |
|
|
Akanthomyces muscarius CG935 |
Dry powder |
Suspended in 0.05% Tween-80 solution, when use |
Bemisia tabaci, Aphis fabae |
[47] |
|
Akanthomyces lecanii CG824 |
Dry powder |
Suspended in 0.05% Tween-80 solution, when use |
Bemisia tabaci, Aphis fabae, Planococcus sp. |
[47] |
|
Beauveria bassiana ART2587 |
Emulsifiable oil |
colza oil, surfactant |
Brassicogethes spp. |
[45] |
|
Beauveria bassiana GHA |
Wettable powder |
diatomaceous earth |
Plutella xylostella |
[24] |
|
Beauveria bassiana GHA |
Wettable powder co-formulated with Bacillus thuringiensis |
montmorillonite K10 clay, halloysite nanoclay, albumin, sodium bicarbonate, calcium cassinate, chitosan |
Trichoplusia ni |
[48] |
|
Beauveria bassiana ESALQ1432 |
Wettable powder |
diatomaceous earth |
Tenebrio molitor |
[32] |
|
Beauveria bassiana Li- and ILB-series |
Wettable powder |
diatomaceous earth |
Thaumastocoris peregrinus |
[49] |
|
Beauveria bassiana Egy-series |
Wettable powder |
Not indicated |
Aulacaspis tubercularis, Icerya seychellarum |
[50] |
|
Cordyceps javanica Wf GA17 |
Emulsifiable oil |
JMS stylet oil |
Bemisia tabaci |
[51] |
|
Metarhizium anisopliae 97 |
Dry powder |
Suspended in 0.1% Tween-80 solution, when use |
Locusta migratoria migratorioides |
[26] |
|
Metarhizium anisopliae ESALQ 818 |
Dry powder |
Suspended in 0.01% Tween-80 solution, when use |
Aedes aegypti |
[9] |
|
Metarhizium robertsii ESALQ1426 |
Wettable powder |
bentonite, activated charcoal, Ca-lignin |
Dalbulus maidis |
[52] |
|
Metarhizium robertsii IP |
Granule |
microcrystalline cellulose, psyllium husk |
Rhipicephalus microplus |
[53] |
|
Metarhizium brunneum ARSEF 4556 |
Dry powder |
Suspended in 0.03% Tween-80, when use |
Culex quinquefasciatus |
[46] |
|
Dry powder |
Suspended in 0.03% Tween-80, when use |
Aedes aegypti |
[54] |
|
|
Metarhizium brunneum CB15-III |
Bead |
polyvinyl alcohol, polyethylene glycol, soy lecithin |
Tenebrio molitor |
[55] |
|
Isaria fumosorosea SFP-198 |
Emulsifiable oil |
corn oil, isotridecyl alcohol ethoxylated-3EO, alginic acid sodium |
Lycopersicon esculentum |
[56] |
|
Isaria fumosorosea ARSEF 3581 |
Wettable powder |
Diatomaceous earth, 0.1% Capsil |
Diaphorina citri |
[57] |
|
Isaria fumosorosea PFR-97TM |
Granule |
Inert ingredients (not informed) |
Microtheca ochroloma |
[58] |
3. Physiological Traits of Blastospore and Its Formulation
As discussed above, blastospore production is an essential prerequisite for large-scale application of blastospore-based formulations. Meanwhile, it is important to keep blastospore stability/viability in the subsequent biotechnological process from fermentation, to drying, to formulation, and finally to product storage. Drying blastospores is a desiccation process that imposes stressful challenges on fungal cells, including denaturation of macromolecules, loss of cytomembrane integrity, stoppage of cellular self-protection mechanisms, and so on. Therefore, desiccation is considered as an essential process in formulation development [14]. Dietsch et al. (2021) have summarized a slew of approaches to increase the blastospore tolerance to desiccation. In fermentation, in addition to nutrients, physicochemical conditions (e.g., osmotic stress) are optimized to produce desiccation-tolerant blastospores with an increased survival rate after drying. In addition to additives, formulation types (e.g., powder and granule) and processing method (e.g., encapsulation) are also considered in the fabrication of the final preparation [14]. There are only a limited number of options for formulation types and production methods. Thus, exploring various additives could create opportunities to improve the desiccation tolerance or storage stability of blastospore formulations, which is critical for commercial stability and viability.
As for conidial formulation, many antioxidant enzymes are revealed to be involved in conidial resistance to environmental stresses, including UV irradiation, high temperature, and various agrichemical agents [59]. In addition, mannitol biosynthesis-related enzymes have been functionally characterized in B. bassiana, and their losses greatly weaken conidial multi-stress tolerances [60]. Polyols (e.g., glycerol and mannitol) have been considered as the important index of blastospore quality, and the increased level of polyols enhances blastospore viability under stressful conditions. Accumulation of polyols is modified by nutrients and cultural conditions [20]. However, very few investigations provided the direct mechanisms on the environmental stability of blastospores.
Spore viability investigations indicate that conidia retained their stability for a longer period than blastospores [61]. Therefore, the current main challenges are to increase blastospore production and formulation stability. In depth-exploration of molecular mechanisms is very necessary for blastospore biogenesis and stress tolerance, which will enhance blastospore physiology via genetic modification.
4. Molecular Genetics and Blastospore Biogenesis
In the past decade, genetic dissection of functional genes has been greatly cumulated with the publication of the genomic sequences for a series of insect pathogenic fungi [62]. A recent review has summarized the understanding of sub-cellular structures (e.g., organelles and cell wall) and their associated proteins in asexual development (i.e., conidiation and blastospore generation) in entomopathogenic fungi [63]. Here, we focus on the molecular insights known about functional genes, signal transduction, and transcriptional regulation involved in fungal development into blastospores. Gene functions are analyzed through gene disruption with a strategy of homologous recombination [64]. However, most investigations are limited to blastospore formation under flask-scale assay conditions.
4.1. Signal Reception Pathways
G-protein signaling pathways are characterized by the recognition of environmental stimuli by the membrane-bound G-protein coupled receptor (Gpcr) and play essential roles in cell development and differentiation [64]. In B. bassiana, GPCR3 contributes to fungal development and stress resistance. Blastospore production is dramatically attenuated in the gene disruption mutant when cultured in minimal broth with glucose as a single carbon source. This phenotypic defect is repressed when using the trehalose-based minimal broth. BbGpcr3 mediates the glucose-induced blastospore production, and trehalose regulates blastospore formation via an alternative signal-reception pathway [65]. This finding suggests that in in vitro production of blastospores, BbGpcr3 mediates fungal response to different carbon sources. Glucose and trehalose are prevalent in the insect hemolymph [66]. Filamentous fungi preferentially utilize glucose as the favorite carbon source [67]. These findings imply that BbGpcr3 is involved in the early stage of in vivo dimorphism, when the fungus first reaches the host hemocoel, and ultimately contributes to fungal virulence [65]. Regulators of G protein signaling (RGS proteins) constitute the key elements of GPCR complexes and play important roles in conidiation of B. bassiana [68]. Unraveling their roles in blastospore generation will improve understanding of the G-protein signaling pathway involved in fungal development under submerged condition.
4.2. Signal Transduction Pathways
SNF1/AMPK protein kinase is highly conserved in eukaryotic organisms and regulates carbohydrate metabolism and energy generation [69]. In filamentous fungi, SNF1 is critical for fungal assimilation of complex carbon sources (e.g., cellulose and pectin) and asexual conidiation [70]. In addition to its well-known roles, SNF1 contributes to blastospore production and size in B. bassiana. Furthermore, the SNF1-mediated transcriptome is associated with metabolism, cell cycle, and substrate transport during blastospore formation [71].
Autophagy is a conserved cellular self-degradation mechanism for damaged and superfluous substrates [72]. More than forty genes have been characterized as autophagy-related genes (ATGs). In B. bassiana, autophagy and its related genes are required for fungal development into blastospores [73]. Atg1 is a serine/threonine protein kinase indispensable for autophagy initiation. B. bassiana Atg1 (BbAtg1) mediates a comprehensive proteome and phosphoproteome during conidiation, and this phosphoproteome is associated with various physiological terms, including metabolism, signal transduction, cell cycle, autophagy, and the like [74]. BbAtg1 plays an important role in blastospore production [75]. Presumably, Atg1 might also phosphorylate a slew of targets for blastospore formation in B. bassiana.
Mitogen activated protein kinase (MAPK) cascade is a prevalent signaling transduction pathway by which eukaryotic cells respond to environmental changes [76]. In B. bassiana, the homolog of yeast High-osmolarity glycerol 1 (Hog1) is a functional MAPK, and its loss has no significant effects on the formation of in vivo blastospores [77]. However, the MAPK kinase Ste7 is involved in blastospore formation and its activity is regulated by four C-terminal Ser/Thr residues [78]. ΔBbgpcr3 mutant strain restores the blastospore production in the trehalose-based broth, and most genes in MAPK signaling pathways appear in the trehalose-induced transcriptome [65]. Many MAPK components are critical for aerial development of entomopathogenic fungi, e.g., Mpk1 (Fus3/Kss1 pathway) and Slt2 (cell wall integrity pathway) [79]. In M. acridum, a FUS3/KSS1-type mitogen activated protein kinase is required for appressorium formation, cuticle penetration, and virulence of the entomopathogenic fungus [80]. Thus, the roles of MAPK members in blastospore formation are yet to be revealed in future investigations.
Protein phosphatase type 1 (PP1) dephosphorylates serine and threonine residues of phosphoproteins and plays an important role in fungal metabolism and development. A yeast ortholog of Glc8 contributes to fungal development into blastospores in B. bassiana, and genetic analysis indicates that Glc8 mediates the transcription of OSMC2 (a member of OsmC protein family) during blastospore genesis [81]. Overall, the phosphorylation and its converse process are associated with a variety of target proteins during blastospore generation, and these processes are balanced by a complex regulatory network.
As summarized above, understanding of signal transduction remains fairly limited in blastospore formation; particularly, cross-talk among different pathways. SNF1/AMPK pathway acts as the energy-sensing one, and the mechanistic target-of-rapamycin complex 1 (mTORC1) functions as the key sensor of cellular amino acids and glucose. SNF1/AMPK acts as a secondary modulator for dissociation of mTORC1 form the lysosome/vacuole when cellular responding to nutrient availability [69]. What the induction signals for blastospore formation are, and how these signaling pathways interplay, remain important and active areas of investigation.
4.3. Transcriptional Regulation Factors
Cell-division control is essential for fungal differentiation, and the cell-division cycle includes four stages of genome duplication (S-phase), nuclear division (M-phase), and two gap phases (G1 and G2). At the checkpoint of G1/S transition, transcription processes are regulated by two transcription-factor complexes (i.e., SBF and MBF), in which Swi6 acts as a common transcriptional activator, generating the SBF and MBF complexes with DNA-binding proteins Swi4 and Mbp1, respectively [82]. In B. bassiana, both Swi6 and Mbp1 localize in the nucleus and exhibit a direct interaction relationship. As for biological functions, both factors contribute to fungal dimorphism into blastospores. BbMbp1 contributes to blastospore formation by regulating the genes associated with metabolism, cell transport, and development; whereas, BbSwi6 regulates genes involved in metabolism and energy generation [83,84]. These findings suggest that, in addition to their roles in the MBF complex, Swi6 and Mbp1 function in blastospore production via dissimilar genetic pathways in B. bassiana. Forkhead (Fkh) transcription factors are conserved in eukaryotic organisms and regulate the cell cycle via activation of the cyclin-B gene cluster regulatory elements in the G2 phase. B. bassiana has a homolog of Fkh2, and its loss leads to a great increase in blastospore yield but a reduction in cell size [85]. Thus, transcriptional activation of cell cycle dependent activities is essential for blastospore generation.
Carbon catabolite repression is prevalent in fungi. In yeast, three transcription factors (Mig1, 2, and 3) contain Cys2His2 zinc-finger motif with DNA-binding activity and are required for transcriptional activation of the glucose-repressed genes [86]. In filamentous fungi, CreA is the homolog of yeast Mig1. B. bassiana CreA plays important roles in conidiation and blastospore production, in addition to its function as a carbon metabolism repressor [87]. As mentioned above, B. bassiana Gpcr3 couples carbon sensing to fungal development into blastospores [53]. However, more genetic evidence is still needed to elucidate the connection between signal sensing and transcriptional regulation pathways.
Zn(II)2Cys6 transcription factors are fungal specific transcription regulators. Tpc1 (Transcription factor for Polarity Control 1) belongs to this family and regulates chitin synthesis during blastospore generation [88]. In yeast, the transcription factor Wor1 is a master regulator of cell morphological transformation. B. bassiana Wor1 is required for blastospore production via transcriptional activation of cell-wall-protein genes (e.g., allergen-like protein gene) [89].
Multiprotein bridging factor 1 (Mbf1) is a highly conserved transcriptional co-activator. In general, Mbf1 mediates the connection between the basal transcription machinery and the transcription factor. In B. bassiana, Mbf1 contributes to the blastospore production in minimal media with saccharide as the sole carbon source; however, this impaired phenotype is not present on the rich medium [90]. This finding implies that Mbf1 mediates assimilation of saccharides during blastospore formation; however, the transcription factor recruited by Mbf1 remains to be elucidated.
Comparative transcriptomics indicates that M. anisopliae activates a series of physiological processes to produce blastospores, including oxidative stress, amino acid metabolism, respiration process, transmembrane transport, and secondary metabolism [91]. Blastospore production of B. bassiana is dramatically increased by combinational application of high glucose concentrations and aeration. Transcriptomic analysis reveals that the up-regulated genes by high glucose concentrations are related to cellular antioxidant, calcium transport, conidiation, and osmotic sensor [92].
Current researches have coupled transcription of the cell cycle and metabolism with fungal dimorphism. Accumulated transcriptomic data will facilitate the discovery of transcriptional regulation hubs during blastospore genesis.
4.4. Cell Cycle-Related Factors
Cell cycle is finely tuned for cell proliferation and development. Cyclin-dependent kinase 1 (Cdk1) determines the checkpoint of G2/M transition, and its phosphorylation and dephosphorylation processes are regulated by the nuclear kinase Wee1 and cell division cycle 25 (Cdc25, a dual-specificity phosphatase). In B. bassiana, the Cdk1 phosphorylation state is also controlled by the homologs of Wee1 and Cdc25, and single disruption of Wee1 and Cdc25 results in significant decrease in blastospore production and alteration in blastospore size [93]. Tudor domain-containing protein (Tdp1) contributes to Cdk1 activity and regulates the S, G2/M, and G0/G1 phases in the cell cycle involved in blastospore formation [94]. In yeast, Cdc14 inactivates CDK activity by dephosphorylation. Its homolog controls cytokinesis and fungal differentiation into blastospores in B. bassiana [95]. Cdc42, a small GTPase, functions as a switch molecule in cell cycle and polarized growth, and participates in blastospore generation via controlling pyruvate metabolism [96]. Cell division cycle factors participate in blastospore formation through potential multiple pathways.
4.5. Epigenetics
Epigenetics refers to the study of changes in gene expression that are not ascribed to alterations in the DNA sequence in response to intrinsic and extrinsic stimulations. Epigenetic regulatory mechanisms encompass DNA methylation, histone modification, chromatin remodeling, and microRNA expression [97]. The histone acetyltransferase (HAT) Gcn5 acts as a core subunit of the HAT complex. In B. bassiana, Gcn5 directly interacts with Ada2, which binds to Ada3, generating the HAT complex [98], and this complex is essential for the fungus to produce blastospores [99]. Histone deacetylase (HDA) represents a superfamily of enzymes that catalyze the reverse reaction of histone acetylation. Rpd3 and Sir2 belong to class I and class III HAD, respectively, and these HADs significantly contribute to blastospore production [100,101]. So, histone acetylation is greatly involved in comprehensive physiologies during fungal development, and the downstream targets remain largely unknown. Currently, only histone acetylation has been evaluated in entomopathogenic fungi, and other epigenetic mechanisms are highly anticipated in future studies on blastospore formation.
4.6. Central Developmental Pathway
The central developmental pathway (CDP), which involves three major transcription factors, BrlA, AbaA, and WetA, regulates the temporal and spatial expression of conidiation-related genes. In B. bassiana and M. robertsii, the CDP transcription factors have additional roles in blastospore formation [102,103,104]. The E3 ubiquitin ligase Ubr1 plays a key role in protein ubiquitylation as revealed in yeast. The Ubr1-mediated ubiquitylation regulates fungal dimorphic change in B. bassiana via transcriptional activation of genes involved in the central developmental pathway (BrlA, AbaA, and WetA) [105]. In filamentous fungi, the upstream developmental activation pathway (UDP) is essential for activation of BrlA gene when conidiation is initiated, which involves the key activator FluG (fluffy gene). FluG constitutes three transcriptional regulatory pathways with FlbA, FlbC, and FlbE-FlbD-FlbB axis [106]. However, FluG and other FluG-like proteins have a limited contribution to conidiation in B. bassiana, and negatively regulates blastospore formation under in vitro condition [107,108]. In addition, Zhang et al. (2019) summarized that the transcription of CDP genes are mediated by other pathways (e.g., histone post-translational modification and MAPK cascade) during conidiation [102]. However, the details underlying the interaction of CDP with other pathways remain largely unknown in blastospore biogenesis.
4.7. The Pathways for Micronutrient Acquisition
As revealed in C. javanica, exogenous metal ions increase the blastospore production [27]. Siderophores represent a group of small molecule iron chelators and are critical for iron acquisition in filamentous fungi. B. bassiana ARSEF 2860 holds a general siderophore biosynthesis pathway to produce a slew of siderophores. Ablation of siderophore synthesis results in a significant reduction in blastospore formation under the iron-limited condition [109]. B. bassiana ARSEF 3153 is a strain that does not produce siderophores at the early stage of growth. Overexpression of N5-hydroxyornithine acetylase gene (SidL) activates the siderophore production in early growth and increases the blastospore yield [110]. This implicates that the pathways for nutrient assimilation are the potential targets for the strain improvement in blastospore production. However, to date, pathways for acquiring micronutrients are limited in filamentous entomopathogenic fungi.
4.8. Other Proteins Related to Blastospore Biogenesis
14-3-3 protein represents a family of structurally similar phospho-binding proteins that regulate multiple cellular functions. In B. bassiana, Bmh1 and Bmh2 contribute equally to physiologies, and their single mutants show similar development defects in blastospore biogenesis, with a reduction of 60% in production and a decrease in cell size [111]. Mas5 and Mdj1 belong to the heat shock protein 40 (Hsp40) family, and their homologs contribute to about 60% and 80% of blastospore production in B. bassiana, respectively [112,113]. Gelsolin represents a superfamily of actin-binding proteins that contain three or six gelsolin-like domains. B. bassiana has a unique CapG protein (designated as BbGel1) with three gelsolin-like domains. BbGel1 mediates a comprehensive proteome during blastospore formation, and at least regulates the cellular level of a hydrophobin-like protein (Hyd4) [114]. Cyclophilin B is one of the prototypical proteins of the cyclophilin family. In B. bassiana, the homolog of cyclophilin B is localized in the cell wall and plays an essential role in blastospore production [115]. Class II lysyl-tRNA synthetase (KRS) is involved in cytosolic protein synthesis in budding yeast. Ablation of its homolog in B. bassiana results in an approximate 70% reduction in blastospore yield [116].
More and more functional genes have been linked to fungal development into blastospores under the flask-scale conditions, but their connections to large-scale production remain to be completely explored.
5. Conclusions and Outlook
In the past decade, great efforts have been made to explore the EPF blastospore as a new infectious inoculum in biocontrol of insect pests. For the large-scale production, utilization of low-cost materials and optimal physiochemical conditions are highly desirable in the process of fermentation, and optimization of ingredients and additives is greatly demanded in the formulation process. Advances in the molecular mechanisms of blastospore biogenesis will facilitate genetic engineering of pathways and functional genes, but more efforts are needed to explore the regulatory networks and interplay mechanisms among different pathways, particularly those involved in blastospore formation under large-scale production conditions. Furthermore, it is a main challenge to enhance blastospore viability/vitality during formulation and storage, in which the mechanisms remain to be revealed. Molecular understandings of blastospore biogenesis and bioactivity will open opportunities for prevision cell design, facilitating the production of the blastospores with economical productivity coupled with quality and effectiveness.
Supplementary Materials
The following supporting information can be found at: https://www.sciepublish.com/article/pii/1191, Table S1: Medium composition for blastospore production of various entomopathogenic fungi.
Author Contributions
N.H.: Formal analysis, Investigation, Writing—original draft. H.-R.X.: Formal analysis, Investigation. Z.-K.Z.: Formal analysis, Investigation. M.-G.F.: Writing—review & editing. S.-H.Y.: Conceptualization, Funding acquisition, Supervision, Writing—review & editing.
Ethics Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Not applicable.
Funding
This work was supported by National Natural Science Foundation of China (32572913) and Natural Science Foundation of Zhejiang Province (LZ24C140002).
Declaration of Competing Interest
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
References
- Meyling NV, Eilenberg J. Ecology of the entomopathogenic fungi Beauveria bassiana and Metarhizium anisopliae in temperate agroecosystems: Potential for conservation biological control. Biol. Control 2007, 43, 145–155. DOI:10.1016/j.biocontrol.2007.07.007 [Google Scholar]
- Ortiz-Urquiza A, Keyhani NO. Action on the surface: Entomopathogenic fungi versus the insect cuticle. Insects 2013, 4, 357–374. DOI:10.3390/insects4030357 [Google Scholar]
- Ding JL, Hou J, Feng MG, Ying SH. Transcriptomic analyses reveal comprehensive responses of insect hemocytes to mycopathogen Beauveria bassiana, and fungal virulence-related cell wall protein assists pathogen to evade host cellular defense. Virulence 2020, 11, 1352–1365. DOI:10.1080/21505594.2020.1827886 [Google Scholar]
- Corrêa B, Duarte VD, Silva DM, Mascarin GM, Delalibera I. Comparative analysis of blastospore production and virulence of Beauveria bassiana and Cordyceps fumosorosea against soybean pests. Biocontrol 2020, 65, 323–337. DOI:10.1007/s10526-020-09999-6 [Google Scholar]
- Hansen GH, Lübeck M, Frisvad JC, Lübeck PS, Andersen B. Production of cellulolytic enzymes from ascomycetes: Comparison of solid state and submerged fermentation. Process Biochem. 2015, 50, 1327–1341. DOI:10.1016/j.procbio.2015.05.017 [Google Scholar]
- Lopez-Perez M, Rodriguez-Gomez D, Loera O. Production of conidia of Beauveria bassiana in solid-state culture: Current status and future perspectives. Crit. Rev. Biotechnol. 2015, 35, 334–341. DOI:10.3109/07388551.2013.857293 [Google Scholar]
- Holder DJ, Keyhani NO. Adhesion of the entomopathogenic fungus Beauveria (Cordyceps) bassiana to substrata. Appl. Environ. Microbiol. 2005, 71, 5260–5266. DOI:10.1128/AEM.71.9.5260-5266.2005 [Google Scholar]
- Dong TY, Zhang BW, Wen QF, Hu QB. The production relationship of destruxins and blastospores of Metarhizium anisopliae with virulence against Plutella xylostella. J. Integr. Agric. 2016, 15, 1313–1320. DOI:10.1016/S2095-3119(15)61322-3 [Google Scholar]
- de Paula AR, Silva LEI, Ribeiro A, da Silva GA, Silva CP, Butt TM, et al. Metarhizium anisopliae blastospores are highly virulent to adult Aedes aegypti, an important arbovirus vector. Parasit. Vectors 2021, 14, 555. DOI:10.1186/s13071-021-05055-z [Google Scholar]
- Xu HR, Yang JP, Yu QX, Xu HJ, Feng MG, Ying SH. The entomopathogenic fungus Beauveria bassiana employs heterokaryon incompatibility genes in its competitive mechanism against cuticular yeasts of brown planthoppers. Pest Manag. Sci. 2026, 82, 1113–1120. DOI:10.1002/ps.70269 [Google Scholar]
- Mascarin GM, Jackson MA, Kobori NN, Behle RW, Júnior ÍD. Liquid culture fermentation for rapid production of desiccation tolerant blastospores of Beauveria bassiana and Isaria fumosorosea strains. J. Invertebr. Pathol. 2015, 127, 11–20. DOI:10.1016/j.jip.2014.12.001 [Google Scholar]
- Behle RW, Wu S, Toews MD, Duffield KR, Shapiro-Ilan DI. Comparing production and efficacy of Cordyceps javanica with Cordyceps fumosorosea. J. Econ. Entomol. 2022, 115, 455–461. DOI:10.1093/jee/toac002 [Google Scholar]
- Iwanicki NS, Lopes ECM, de Lira AC, Poletto TB, Fonceca LZ, Júnior ID. Comparative analysis of Beauveria bassiana submerged conidia with blastospores: Yield, growth kinetics, and virulence. Biol. Control 2023, 185, 105314. DOI:10.1016/j.biocontrol.2023.105314 [Google Scholar]
- Dietsch R, Jakobs-Schönwandt D, Grünberger A, Patel A. Desiccation-tolerant fungal blastospores: From production to application. Curr. Res. Biotechnol. 2021, 3, 323–339. DOI:10.1016/j.crbiot.2021.11.005 [Google Scholar]
- Mascarin GM, Golo PS, de Souza Ribeiro-Silva C, Muniz ER, de Oliveira Franco A, Kobori NN, et al. Advances in submerged liquid fermentation and formulation of entomopathogenic fungi. Appl. Microbiol. Biotechnol. 2024, 108, 451. DOI:10.1007/s00253-024-13287-z [Google Scholar]
- Kleespies RG, Zimmermann G. Production of blastospores by three strains of Metarhizium anisopliae (Metch.) Sorokin in submerged culture. Biocontrol Sci. Technol. 1992, 2, 127–135. DOI:10.1080/09583159209355226 [Google Scholar]
- Issaly N, Chauveau H, Aglevor F, Fargues J, Durand A. Influence of nutrient, pH and dissolved oxygen on the production of Metarhizium flavoviride Mf189 blastospores in submerged batch culture. Process Biochem. 2005, 40, 1425–1431. DOI:10.1016/j.procbio.2004.06.029 [Google Scholar]
- Ortiz-Urquiza A, Garrido-Jurado I, Borrego A, Quesada-Moraga E. Effects of cultural conditions on fungal biomass, blastospore yields and toxicity of fungal secreted proteins in batch cultures of Metarhizium anisopliae (Ascomycota: Hypocreales). Pest Manag. Sci. 2010, 66, 725–735. DOI:10.1002/ps.1934 [Google Scholar]
- Iwanicki NS, Ferreira BO, Mascarin GM, Júnior ÍD. Modified Adamek’s medium renders high yields of Metarhizium robertsii blastospores that are desiccation tolerant and infective to cattle-tick larvae. Fungal Biol. 2018, 122, 883–890. DOI:10.1016/j.funbio.2018.05.004 [Google Scholar]
- Ypsilos IK, Magan N. Characterisation of optimum cultural environmental conditions for the production of high numbers of Metarhizium anisopliae blastospores with enhanced ecological fitness. Biocontrol Sci. Technol. 2005, 15, 683–699. DOI:10.1080/09583150500136774 [Google Scholar]
- Cliquet S, Jackson M. Influence of culture conditions on production and freeze-drying tolerance of Paecilomyces fumosoroseus blastospores. J. Ind. Microbiol. Biotechnol. 1999, 23, 97–102. DOI:10.1038/sj.jim.2900698 [Google Scholar]
- Chong-Rodríguez MJ, Maldonado-Blanco MG, Hernández-Escareño JJ, Galán-Wong LJ, Sandoval-Coronado CF. Study of Beauveria bassiana growth, blastospore yield, desiccation-tolerance, viability and toxic activity using different liquid media. Afr. J. Biotechnol. 2011, 10, 5736–5742. Available online: https://www.ajol.info/index.php/ajb/article/view/94446/83819 (accessed on 27 August 2026).
- Pham TA, Kim JJ, Kim SG, Kim K. Production of blastospore of entomopathogenic Beauveria bassiana submerged batch culture. Mycobiology 2009, 37, 218–224. DOI:10.4489/MYCO.2009.37.3.218 [Google Scholar]
- Fargues J, Smits N, Vidal C, Vey A, Vega F, Mercadier G, et al. Effect of liquid culture media on morphology, growth, propagule production, and pathogenic activity of the Hyphomycete, Metarhizium flavoviride. Mycopathologia 2002, 154, 127–138. DOI:10.1023/A:1016068102003 [Google Scholar]
- Cliquet S, Jackson MA. Impact of carbon and nitrogen nutrition on the quality, yield and composition of blastospores of the bioinsecticidal fungus Paecilomyces fumosoroseus. J. Ind. Microbiol. Biotechnol. 2005, 32, 204–210. DOI:10.1007/s10295-005-0232-3 [Google Scholar]
- Kleespies RG, Zimmermann G. Effect of additives on the production, viability and virulence of blastospores of Metarhizium anisopliae. Biocontrol Sci. Technol. 1998, 8, 207–214. DOI:10.1080/09583159830270 [Google Scholar]
- Li Y, Gao M, Chen S, Diao H, Zhou W. Production of heat-resistant blastospores by Cordyceps javanica IF-1106 through optimizing metal ions composition. Biol. Control 2024, 193, 105518. DOI:10.1016/j.biocontrol.2024.105518 [Google Scholar]
- Song G, Lee MR, Kim JS. Production of mite-pathogenic Akanthomyces attenuatus JEF-147 blastospores in flask and bioreactor conditions. Mycobiology 2025, 53, 572–583. DOI:10.1080/12298093.2025.2532235 [Google Scholar]
- Wingfield LK. Morphological study, production and cryopreservation of blastospores of entomopathogenic fungi. ScienceAsia 2020, 46, 557–567. DOI:10.2306/scienceasia1513-1874.2020.078 [Google Scholar]
- Jackson MA, Payne AR, Odelson DA. Liquid-culture production of blastospores of the bioinsecticidal fungus Paecilomyces fumosoroseus using portable fermentation equipment. J. Ind. Microbiol. Biotechnol. 2004, 31, 149–154. DOI:10.1007/s10295-004-0127-8 [Google Scholar]
- Jackson MA, Cliquet S, Iten LB. Media and fermentation processes for the rapid production of high concentrations of stable blastospores of the bioinsecticidal fungus Paecilomyces fumosoroseus. Biocontrol Sci. Technol. 2003, 13, 23–33. DOI:10.1080/0958315021000054368 [Google Scholar]
- Mascarin GM, Kobori NN, Coleman JJ, Jackson MA. Impact of osmotic stress on production, morphology, and fitness of Beauveria bassiana blastospores. Appl. Microbiol. Biotechnol. 2023, 107, 4815–4831. DOI:10.1007/s00253-023-12631-z [Google Scholar]
- Téllez-Martínez MG, Alcalá-Gómez G, Jiménez-Islas H, Navarrete-Bolaños JL. Design of an efficient fermentation process for the production of Metarhizium acridum blastospores. Biocontrol Sci. Technol. 2016, 26, 1652–1667. DOI:10.1080/09583157.2016.1231775 [Google Scholar]
- Jackson MA. Dissolved oxygen levels affect dimorphic growth by the entomopathogenic fungus Isaria fumosorosea. Biocontrol Sci. Technol. 2012, 22, 67–79. DOI:10.1080/09583157.2011.642339 [Google Scholar]
- Mascarin GM, Jackson MA, Kobori NN, Mascarin GM, Jackson MA, Kobori NN, et al. Glucose concentration alters dissolved oxygen levels in liquid cultures of Beauveria bassiana and affects formation and bioefficacy of blastospores. Appl. Microbiol. Biotechnol. 2015, 99, 6653–6665. DOI:10.1007/s00253-015-6620-3 [Google Scholar]
- Lozano-Contreras MG, Elías-Santos M, Rivas-Morales C, Luna-Olvera HA, Galán-Wong LJ, Maldonado-Blanco MG. Paecilomyces fumosoroseus blastospore production using liquid culture in a bioreactor. Afr. J. Biotechnol. 2007, 6, 2095–2099. DOI:10.5897/AJB2007.000-2326 [Google Scholar]
- Ypsilos IK, Magan N. Impact of water-stress and washing treatments on production, synthesis and retention of endogenous sugar alcohols and germinability of Metarhizium anisopliae blastospores. Mycol. Res. 2004, 108, 1337–1345. DOI:10.1017/S0953756204001030 [Google Scholar]
- Jackson MA, Payne AR. Evaluation of the desiccation tolerance of blastospores of Paecilomyces fumosoroseus (Deuteromycotina: Hyphomycetes) using a lab-scale, air-drying chamber with controlled relative humidity. Biocontrol Sci. Technol. 2007, 17, 709–719. DOI:10.1080/09583150701527235 [Google Scholar]
- Lima VH, Matugawa AT, Mascarin GM, Fernandes ÉKK. Complex nitrogen sources from agro-industrial byproducts: Impact on production, multi-stress tolerance, virulence, and quality of Beauveria bassiana blastospores. Microbiol. Spectr. 2024, 12, e0404023. DOI:10.1128/spectrum.04040-23 [Google Scholar]
- Cliquet S, Jackson MA. Comparison of air-drying methods for evaluating the desiccation tolerance of liquid culture-produced blastospores of Paecilomyces fumosoroseus. World J. Microbiol. Biotechnol. 1997, 13, 299–303. DOI:10.1023/A:1018535124352 [Google Scholar]
- Sandoval-Coronado CF, Luna-Olvera HA, Arévalo-Niño K, Jackson MA, Poprawski TJ, Galán-Wong LJ. Drying and formulation of blastospores of Paecilomyces fumuosoroseus (Hyphomycetes) produced in two different liquid media. World J. Microbiol. Biotechnol. 2001, 17, 423–428. DOI:10.1023/A:1016757608789 [Google Scholar]
- Mascarin GM, Jackson MA, Behle RW, Kobori NN, Júnior ÍD. Improved shelf life of dried Beauveria bassiana blastospores using convective drying and active packaging processes. Appl. Microbiol. Biotechnol. 2016, 100, 8359–8370. DOI:10.1007/s00253-016-7597-2 [Google Scholar]
- Jackson MA, Mcguire MR, Lacey LA, Wraight SP. Liquid culture production of desiccation tolerant blastospores of the bioinsecticidal fungus Paecilomyces fumosoroseus. Mycol. Res. 1997, 101, 35–41. DOI:10.1017/S0953756296002067 [Google Scholar]
- Jackson MA, Erhan S, Poprawski TJ. Influence of formulation additives on the desiccation tolerance and storage stability of blastospores of the entomopathogenic fungus Paecilomyces fumosoroseus (Deuteromycotina: Hyphomycetes). Biocontrol Sci. Technol. 2006, 16, 61–75. DOI:10.1080/09583150500188197 [Google Scholar]
- Kaiser D, Handschin S, Rohr RP, Bacher S, Grabenweger G. Co-formulation of Beauveria bassiana with natural substances to control pollen beetles—Synergy between fungal spores and colza oil. Biol. Control 2020, 140, 104106. DOI:10.1016/j.biocontrol.2019.104106 [Google Scholar]
- Alkhaibari AM, Lord AM, Maffeis T, Bull JC, Olivares FL, Samuels RI, et al. Highly specific host-pathogen interactions influence Metarhizium brunneum blastospore virulence against Culex quinquefasciatus larvae. Virulence 2018, 9, 1449–1467. DOI:10.1080/21505594.2018.1509665 [Google Scholar]
- Lopes RB, Souza TAD, Mascarin GM, Souza DA, Bettiol W, Souza HR, et al. Akanthomyces diversity in Brazil and their pathogenicity to plant-sucking insects. J. Invertebr. Pathol. 2023, 200, 107955. DOI:10.1016/j.jip.2023.107955 [Google Scholar]
- Sayed AMM, Behle RW. Comparing formulations for a mixed-microbial biopesticide with Bacillus thuringiensis var. kurstaki and Beauveria bassiana blastospores. Arch. Phytopathol. Plant Protect. 2017, 50, 745–760. DOI:10.1080/03235408.2017.1372942 [Google Scholar]
- Abreo E, Simeto S, Corallo B, Martínez G, Lupo S, Altier N. Dual selection of Beauveria bassiana strains and complex substrate media for the massive production of submerged propagules with activity against the eucalyptus bronze bug Thaumastocoris peregrinus. Biocontrol Sci. Technol. 2019, 29, 533–546. DOI:10.1080/09583157.2019.1566952 [Google Scholar]
- Sayed AMM, Dunlap CA. Virulence of some entomopathogenic fungi isolates of Beauveria bassiana (Hypocreales: Cordycipitaceae) and Metarhizium anisopliae (Hypocreales: Clavicipitaceae) to Aulacaspis tubercularis (Hemiptera: Diaspididae) and Icerya seychellarum (Hemiptera: Monophlebidae) on mango crop. J. Econ. Entomol. 2019, 112, 2584–2596. DOI:10.1093/jee/toz187 [Google Scholar]
- Wu S, Toews MD, Behle RW, Barman AK, Sparks AN, Simmons AM, et al. Post-application field persistence and efficacy of Cordyceps javanica against Bemisia tabaci. J. Fungi 2023, 9, 827. DOI:10.3390/jof9080827 [Google Scholar]
- Iwanicki NS, Mascarin GM, Moreno SG, Eilenberg J, Delalibera I, Jr. Development of novel spray-dried and air-dried formulations of Metarhizium robertsii blastospores and their virulence against Dalbulus maidis. Appl. Microbiol. Biotechnol. 2021, 105, 7913–7933. DOI:10.1007/s00253-021-11576-5 [Google Scholar]
- Marciano AF, Mascarin GM, Franco RFF, Golo PS, Jaronski ST, Fernandes ÉKK, et al. Innovative granular formulation of Metarhizium robertsii microsclerotia and blastospores for cattle tick control. Sci. Rep. 2021, 11, 4972. DOI:10.1038/s41598-021-84142-8 [Google Scholar]
- Alkhaibari AM, Maffeis T, Bull JC, Butt TM. Combined use of the entomopathogenic fungus, Metarhizium brunneum, and the mosquito predator, Toxorhynchites brevipalpis, for control of mosquito larvae: Is this a risky biocontrol strategy? J. Invertebr. Pathol. 2018, 153, 38–50. DOI:10.1016/j.jip.2018.02.003 [Google Scholar]
- Hermann KM, Grünberger A, Patel AV. Polyvinyl alcohol coating releasing fungal blastospores improves kill effect of attract-and-kill beads. AMB Express 2023, 13, 72. DOI:10.1186/s13568-023-01575-2 [Google Scholar]
- Kim JS, Je YH, Skinner M, Parker BL. An oil-based formulation of Isaria fumosorosea blastospores for management of greenhouse whitefly Trialeurodes vaporariorum (Homoptera: Aleyrodidae). Pest Manag. Sci. 2013, 69, 576–581. DOI:10.1002/ps.3497 [Google Scholar]
- Morales-Reyes C, Mascarin GM, Jackson MA, Hall D, Sánchez-Peña SR, Arthurs SP. Comparison of aerial conidia and blastospores from two entomopathogenic fungi against Diaphorina citri (Hemiptera: Liviidae) under laboratory and greenhouse conditions. Biocontrol Sci. Technol. 2018, 28, 737–749. DOI:10.1080/09583157.2018.1487028 [Google Scholar]
- Montemayor CO, Avery PB, Cave RD. Infection and mortality of Microtheca ochroloma (Coleoptera: Chrysomelidae) by Isaria fumosorosea (Hypocreales: Cordycipitaceae) under laboratory conditions. Biocontrol Sci. Technol. 2016, 26, 605–616. DOI:10.1080/09583157.2015.1126222 [Google Scholar]
- Zhang LB, Feng MG. Antioxidant enzymes and their contributions to biological control potential of fungal insect pathogens. Appl. Microbiol. Biotechnol. 2018, 102, 4995–5004. DOI:10.1007/s00253-018-9033-2 [Google Scholar]
- Wang ZL, Lu JD, Feng MG. Primary roles of two dehydrogenases in the mannitol metabolism and multi-stress tolerance of entomopathogenic fungus Beauveria bassiana. Environ. Microbiol. 2012, 14, 2139–2150. DOI:10.1111/j.1462-2920.2011.02654.x [Google Scholar]
- Hegedus DD, Bidochka MJ, Miranpuri GS, Khachatourians GG. A comparison of the virulence, stability and cell-wall-surface characteristics of three spore types produced by the entomopathogenic fungus Beauveria bassiana. Appl. Microbiol. Biotechnol. 1992, 36, 785‒789. DOI:10.1007/BF00172195 [Google Scholar]
- Ortiz-Urquiza A, Keyhani NO. Molecular genetics of Beauveria bassiana infection of insects. Adv. Genet. 2016, 94, 165–249. DOI:10.1016/bs.adgen.2015.11.003 [Google Scholar]
- Ying SH. Subcellular biochemistry and biology of filamentous entomopathogenic fungi. Adv. Appl. Microbiol. 2024, 129, 35–58. DOI:10.1016/bs.aambs.2024.04.002 [Google Scholar]
- Bahn YS, Xue C, Idnurm A, Rutherford JC, Heitman J, Cardenas ME. Sensing the environment: lessons from fungi. Nat. Rev. Microbiol. 2007, 5, 57–69. DOI:10.1038/nrmicro1578 [Google Scholar]
- Ying SH, Feng MG, Keyhani NO. A carbon responsive G-protein coupled receptor modulates broad developmental and genetic networks in the entomopathogenic fungus, Beauveria bassiana. Environ. Microbiol. 2013, 15, 2902–2921. DOI:10.1111/1462-2920.12169 [Google Scholar]
- Lu YX, Zhang Q, Xu WH. Global metabolomic analyses of the hemolymph and brain during the initiation, maintenance, and termination of pupal diapause in the cotton bollworm, Helicoverpa armigera. PLoS ONE 2014, 9, e99948. DOI:10.1371/journal.pone.0099948 [Google Scholar]
- Adnan M, Zheng W, Islam W, Arif M, Abubakar YS, Wang Z, et al. Carbon catabolite repression in filamentous fungi. Int. J. Mol. Sci. 2017, 19, 48. DOI:10.3390/ijms19010048 [Google Scholar]
- Fang W, Scully LR, Zhang L, Pei Y, Bidochka MJ. Implication of a regulator of G protein signalling (BbRGS1) in conidiation and conidial thermotolerance of the insect pathogenic fungus Beauveria bassiana. FEMS Microbiol. Lett. 2008, 279, 146–156. DOI:10.1111/j.1574-6968.2007.00978.x [Google Scholar]
- Lin SC, Hardie DG. AMPK: Sensing glucose as well as cellular energy status. Cell Metab. 2018, 27, 299–313. DOI:10.1016/j.cmet.2017.10.009 [Google Scholar]
- Zhang T, Sun X, Xu Q, Zhu C, Li Q, Li H. PdSNF1, a sucrose non-fermenting protein kinase gene, is required for Penicillium digitatum conidiation and virulence. Appl. Microbiol. Biotechnol. 2013, 97, 5433–5445. DOI:10.1007/s00253-012-4593-z [Google Scholar]
- Wang XX, He PH, Feng MG,Ying SH. BbSNF1 contributes to cell differentiation, extracellular acidification, and virulence in Beauveria bassiana, a filamentous entomopathogenic fungus. Appl. Microbiol. Biotechnol. 2014, 98, 8657–8673. DOI:10.1007/s00253-014-5907-0 [Google Scholar]
- Zhang H. The genetics of autophagy in multicellular organisms. Annu. Rev. Genet. 2022, 56, 17–39. DOI:10.1146/annurev-genet-022422-095608 [Google Scholar]
- Ying SH, Feng MG. Insight into vital role of autophagy in sustaining biological control potential of fungal pathogens against pest insects and nematodes. Virulence 2019, 10, 429–437. DOI:10.1080/21505594.2018.1518089 [Google Scholar]
- Lin HY, Ding JL, Peng YJ, Feng MG, Ying SH. Proteomic and phosphoryproteomic investigations reveal that autophagy-related protein 1, a protein kinase for autophagy initiation, synchronously deploys phosphoregulation on the ubiquitin-like conjugation system in the mycopathogen Beauveria bassiana. mSystems 2022, 7, e0146321. DOI:10.1128/msystems.01463-21 [Google Scholar]
- Ying SH, Liu J, Chu XL, Xie XQ, Feng MG. The autophagy-related genes BbATG1 and BbATG8 have different functions in differentiation, stress resistance and virulence of mycopathogen Beauveria bassiana. Sci. Rep. 2018, 6, 26376. DOI:10.1038/srep26376 [Google Scholar]
- Salat-Canela C, Pérez P, Ayté J, Hidalgo E. Stress-induced cell depolarization through the MAP kinase-Cdc42 axis. Trends Cell Biol. 2023, 33, 124–137. DOI:10.1016/j.tcb.2022.06.004 [Google Scholar]
- Zhang Y, Zhao J, Fang W, Zhang J, Luo Z, Zhang M, et al. Mitogen-activated protein kinase hog1 in the entomopathogenic fungus Beauveria bassiana regulates environmental stress responses and virulence to insects. Appl. Environ. Microbiol. 2009, 75, 3787–3795. DOI:10.1128/AEM.01913-08 [Google Scholar]
- Wang ZK, Cai Q, Tong SM, Ying SH, Feng MG. C-terminal Ser/Thr residues are vital for the regulatory role of Ste7 in the asexual cycle and virulence of Beauveria bassiana. Appl. Microbiol. Biotechnol. 2018, 102, 6973–6986. DOI:10.1007/s00253-018-9148-5 [Google Scholar]
- Luo XD, Keyhani NO, Yu XD, He Z, Luo Z, Pei Y, et al. The MAP kinase Bbslt2 controls growth, conidiation, cell wall integrity, and virulence in the insect pathogenic fungus. Beauveria bassiana. Fungal Genet. Biol. 2012, 49, 544–555. DOI:10.1016/j.fgb.2012.05.002 [Google Scholar]
- Jin K, Han LR, Xia YX. MaMk1, a FUS3/KSS1-type mitogen activated protein kinase gene, is required for appressorium formation, and insect cuticle penetration of the entomopathogenic fungus Metarhizium acridum. J. Invertebr. Pathol. 2014, 115, 68–75. DOI:10.1016/j.jip.2013.10.014 [Google Scholar]
- Peng YJ, Ding JL, Feng MG, Ying SH. Glc8, a regulator of protein phosphatase type 1, mediates oxidation tolerance, asexual development and virulence in Beauveria bassiana, a filamentous entomopathogenic fungus. Curr. Genet. 2019, 65, 283–291. DOI:10.1007/s00294-018-0876-y [Google Scholar]
- Tripodi F, Nicastro R, Busnelli S, Cirulli C, Maffioli E, Tedeschi G, et al. Protein kinase CK2 holoenzyme promotes start-specific transcription in Saccharomyces cerevisiae. Eukaryot. Cell 2013, 12, 1271–1280. DOI:10.1128/EC.00117-13 [Google Scholar]
- Ding JL, Lin HY, Feng MG, Ying SH. Mbp1, a component of the MluI cell cycle box-binding complex, contributes to morphological transition and virulence in the filamentous entomopathogenic fungus Beauveria bassiana. Environ. Microbiol. 2020, 22, 584–597. DOI:10.1111/1462-2920.14868 [Google Scholar]
- Ding JL, Hou J, Li XH, Feng MG, Ying SH. Transcription activator Swi6 interacts with Mbp1 in MluI cell cycle box-binding complex and regulates hyphal differentiation and virulence in Beauveria bassiana. J. Fungi 2021, 7, 411. DOI:10.3390/jof7060411 [Google Scholar]
- Wang JJ, Qiu L, Cai Q, Ying SH, Feng MG. Transcriptional control of fungal cell cycle and cellular events by Fkh2, a forkhead transcription factor in an insect pathogen. Sci. Rep. 2015, 5, 10108. DOI:10.1038/srep10108 [Google Scholar]
- Westholm JO, Nordberg N, Muren E, Ameur A, Komorowski J, Ronne H. Combinatorial control of gene expression by the three yeast repressors Mig1, Mig2 and Mig3. BMC Genomics 2008, 9, 601. DOI:10.1186/1471-2164-9-601 [Google Scholar]
- Luo Z, Qin Y, Pei Y, Keyhani NO. Ablation of the creA regulator results in amino acid toxicity, temperature sensitivity, pleiotropic effects on cellular development and loss of virulence in the filamentous fungus Beauveria bassiana. Environ. Microbiol. 2014, 16, 1122–1136. DOI:10.1111/1462-2920.12352 [Google Scholar]
- Qiu L, Zhang J, Song JZ, Hu SJ, Zhang TS, Li Z, et al. Involvement of BbTpc1, an important Zn(II)2Cys6 transcriptional regulator, in chitin biosynthesis, fungal development and virulence of an insect mycopathogen. Int. J. Biol. Macromol. 2021, 166, 1162–1172. DOI:10.1016/j.ijbiomac.2020.10.271 [Google Scholar]
- Qiu L, Zhang TS, Song JZ, Zhang J, Li Z, Wang JJ. BbWor1, a regulator of morphological transition, is involved in conidium-hypha switching, blastospore propagation, and virulence in Beauveria bassiana. Microbiol. Spectr. 2021, 9, e0020321. DOI:10.1128/Spectrum.00203-21 [Google Scholar]
- Ying SH, Ji XP, Wang XX, Feng MG, Keyhani NO. The transcriptional co-activator multiprotein bridging factor 1 from the fungal insect pathogen, Beauveria bassiana, mediates regulation of hyphal morphogenesis, stress tolerance and virulence. Environ. Microbiol. 2014, 16, 1879–1897. DOI:10.1111/1462-2920.12450 [Google Scholar]
- Iwanicki NS, Júnior ID, Eilenberg J, De Fine Licht HH. Comparative RNAseq analysis of the insect-pathogenic fungus Metarhizium anisopliae reveals specific transcriptome signatures of filamentous and yeast-like development. G3 2020, 10, 2141–2157. DOI:10.1534/g3.120.401040 [Google Scholar]
- Mascarin GM, Iwanicki NS, Ramirez JL, Delalibera Í, Dunlap CA, Jr. Transcriptional responses of Beauveria bassiana blastospores cultured under varying glucose concentrations. Front. Cell Infect. Microbiol. 2021, 11, 644372. DOI:10.3389/fcimb.2021.644372 [Google Scholar]
- Qiu L, Wang JJ, Ying SH, Feng MG. Wee1 and Cdc25 control morphogenesis, virulence and multistress tolerance of Beauveria bassiana by balancing cell cycle-required cyclin-dependent kinase 1 activity. Environ. Microbiol. 2015, 17, 1119–1133. DOI:10.1111/1462-2920.12530 [Google Scholar]
- Qiu L, Li Z, Zhang L, Zhang TS, Hu SJ, Song JZ, et al. The Tudor domain-containing protein BbTdp1 contributes to fungal cell development, the cell cycle, virulence, and transcriptional regulation in the insect pathogenic fungus Beauveria bassiana. Microbiol. Spectr. 2021, 9, e0056421. DOI:10.1128/Spectrum.00564-21 [Google Scholar]
- Wang J, Liu J, Hu Y, Ying SH, Feng MG. Cytokinesis-required Cdc14 is a signaling hub of asexual development and multi-stress tolerance in Beauveria bassiana. Sci. Rep. 2013, 3, 3086. DOI:10.1038/srep03086 [Google Scholar]
- Guan Y, Wang D, Lin X, Li X, Lv C, Wang D, et al. Unveiling a novel role of Cdc42 in pyruvate metabolism pathway to mediate insecticidal activity of Beauveria bassiana. J. Fungi 2022, 8, 394. DOI:10.3390/jof8040394 [Google Scholar]
- Park J, Lee K, Kim K, Yi S-J. The role of histone modifications: from neurodevelopment to neurodiseases. Signal Transduct. Target Ther. 2022, 7, 217. DOI:10.1038/s41392-022-01078-9 [Google Scholar]
- Hu SJ, Zheng H, Li XP, Li ZX, Xu C, Li J, et al. Ada2 and Ada3 regulate hyphal growth, asexual development, and pathogenicity in Beauveria bassiana by maintaining Gcn5 acetyltransferase activity. Microbiol. Spectr. 2023, 11, e0028123. DOI:10.1128/spectrum.00281-23 [Google Scholar]
- Cai Q, Wang JJ, Fu B, Ying SH, Feng MG. Gcn5-dependent histone H3 acetylation and gene activity is required for the asexual development and virulence of Beauveria bassiana. Environ. Microbiol. 2018, 20, 1484–1497. DOI:10.1111/1462-2920.14066 [Google Scholar]
- Cai Q, Wang ZK, Shao W, Ying SH, Feng MG. Essential role of Rpd3-dependent lysine modification in the growth, development and virulence of Beauveria bassiana. Environ. Microbiol. 2018, 20, 1590–1606. DOI:10.1111/1462-2920.14100 [Google Scholar]
- Cai Q, Tian L, Xie JT, Jiang DH, Keyhani NO. Contributions of a histone deacetylase (SirT2/Hst2) to Beauveria bassiana growth, development, and virulence. J. Fungi 2022, 8, 236. DOI:10.3390/jof8030236 [Google Scholar]
- Zhang AX, Mouhoumed AZ, Tong SM, Ying SH, Feng MG. BrlA and AbaA govern virulence-required dimorphic switch, conidiation, and pathogenicity in a fungal insect pathogen. mSystems 2019, 4, e00140-19. DOI:10.1128/mSystems.00140-19 [Google Scholar]
- Wu H, Tong Y, Zhou R, Wang Y, Wang Z, Ding T, et al. Mr-AbaA regulates conidiation by interacting with the promoter regions of both Mr-veA and Mr-wetA in Metarhizium robertsii. Microbiol. Spectr. 2021, 9, e0082321. DOI:10.1128/Spectrum.00823-21 [Google Scholar]
- Zhang JG, Xu SY, Ying SH, Feng MG. Roles of BrlA and AbaA in mediating asexual and insect pathogenic lifecycles of Metarhizium robertsii. J. Fungi 2022, 8, 1110. DOI:10.3390/jof8101110 [Google Scholar]
- Wang DY, Mou YN, Du X, Guan Y, Feng MG. Ubr1-mediated ubiquitylation orchestrates asexual development, polar growth, and virulence-related cellular events in Beauveria bassiana. Appl. Microbiol. Biotechnol. 2021, 105, 2747–2758. DOI:10.1007/s00253-021-11222-0 [Google Scholar]
- Seo J-A, Guan Y, Yu J-H. FluG-dependent asexual development in Aspergillus nidulans occurs via derepression. Genetics 2006, 172, 1535–1544. DOI:10.1534/genetics.105.052258 [Google Scholar]
- Guo CT, Luo XC, Tong SM, Zhou Y, Ying SH, Feng MG. FluG and FluG-like FlrA coregulate manifold gene sets vital for fungal insect-pathogenic lifestyle but not involved in asexual development. mSystems 2022, 7, e0031822. DOI:10.1128/msystems.00318-22 [Google Scholar]
- Guo CT, Peng H, Tong SM, Ying SH, FengMG. Distinctive role of fluG in the adaptation of Beauveria bassiana to insect-pathogenic lifecycle and environmental stresses. Environ. Microbiol. 2021, 23, 5184–5199. DOI:10.1111/1462-2920.15500 [Google Scholar]
- Sun TF, Ge ZW, Xu HR, Zhang H, Huang SS, Feng MG, et al. Unlocking the siderophore biosynthesis pathway and its biological functions in the fungal insect pathogen Beauveria bassiana. J. Agric. Food Chem. 2024, 72, 18455–18464. DOI:10.1021/acs.jafc.4c02957 [Google Scholar]
- Yu QX, Sun TF, Feng MG, Ying SH. Genetic engineering of Beauveria bassiana for enhancing siderophore production and its virulence against the insect hosts. Biotechnol. Lett. 2026, 48, 37. DOI:10.1007/s10529-026-03706-8 [Google Scholar]
- Liu Q, Li JG, Ying SH, Wang JJ, Sun WL, Tian CG, et al. Unveiling equal importance of two 14-3-3 proteins for morphogenesis, conidiation, stress tolerance and virulence of an insect pathogen. Environ. Microbiol. 2015, 17, 1444–1462. DOI:10.1111/1462-2920.12634 [Google Scholar]
- Wang J, Ying SH, Hu Y, Feng MG. Mas5, a homologue of bacterial DnaJ, is indispensable for the host infection and environmental adaptation of a filamentous fungal insect pathogen. Environ. Microbiol. 2016, 18, 1037–1047. DOI:10.1111/1462-2920.13197 [Google Scholar]
- Wang J, Ying SH, Hu Y, Feng MG. Vital role for the J-domain protein Mdj1 in asexual development, multiple stress tolerance, and virulence of Beauveria bassiana. Appl. Microbiol. Biotechnol. 2017, 101, 185–195. DOI:10.1007/s00253-016-7757-4 [Google Scholar]
- He PH, Dong WX, Chu XL, Feng MG, Ying SH. The cellular proteome is affected by a gelsolin (BbGEL1) during morphological transitions in aerobic surface versus liquid growth in the entomopathogenic fungus Beauveria bassiana. Environ. Microbiol. 2016, 18, 4153–4169. DOI:10.1111/1462-2920.13500 [Google Scholar]
- Chu ZJ, Sun HH, Ying SH, Feng MG. Vital role for cyclophilin B (CypB) in asexual development, dimorphic transition and virulence of Beauveria bassiana. Fungal Genet. Biol. 2017, 105, 8–15. DOI:10.1016/j.fgb.2017.05.004 [Google Scholar]
- Zhu XG, Chu ZJ, Ying SH, Feng MG. Lysyl-tRNA synthetase (Krs) acts a virulence factor of Beauveria bassiana by its vital role in conidial germination and dimorphic transition. Fungal Biol. 2017, 121, 956–965. DOI:10.1016/j.funbio.2017.08.003 [Google Scholar]