Tidal Freshwater Forest Restoration at the European Elbe Estuary: Initial Establishment Success of Salix Species
Tidal Freshwater Forest Restoration at the European Elbe Estuary: Initial Establishment Success of Salix Species
Received: 22 June 2026 Revised: 30 July 2026 Accepted: 10 September 2026 Published: 22 September 2026

© 2026 The authors. This is an open access article under the Creative Commons Attribution 4.0 International License (https://creativecommons.org/licenses/by/4.0/).
1. Introduction
Estuaries are characterized by their dynamic nature, and most of them are changing through geological time, but the Anthropocene potentially indicates fast future changes along the LandSea interface [1]. For example, one of the largest deltas of the world, the Río de la Plata in South-America, comprises estuaries which are impacted by agriculture and forestry, hydroelectricity, and shipping infrastructure in addition to urbanization, and it is expected that all of these pressures will increase [2]. On the opposite site of the globe in western Europe, the Delta of the large rivers Rhine, Meuse, and Scheldt (The Netherlands (NL); Belgium (B)) changed due to navigation and flood control infrastructure and land use changes. Such changes contributed to the increased exposure to storm surges, e.g., the storm surge in 1953 led to losses of lives and called for more public safety. The Delta plan (NL) is working to keep NL safe against flooding, and the Sigma Plan (B) is working to keep Flanders safe against flooding. Both plans are meant to enhance adaptive management in these estuaries, which house the largest European ports of Antwerp (B) and Rotterdam (NL), including the need for accessibility for large vessels, simultaneously with nature-based solutions for flood control [3]. For the Elbe estuary (Germany (GER)), the integrated management plan [4] similarly aims to enhance ecological (species, habitats, and processes), economic (e.g., navigation), and social (e.g., flood defense) features of this large estuary, which gives access to the third largest European port of Hamburg [5].
In European lowland estuaries, tidal freshwater wetland forests have established as willow-dominated (species in the genus Salix) forests, which were historically managed for the production of willow branches by coppicing. Along the Scheldt estuary, the Rhine-Meuse estuaries, and the Elbe estuary, Salix shrubs and forests and plantations/coppices exist as relicts in tidal freshwater wetlands at higher elevation above the mean high-water level with less flooding frequency and duration [6]. A literature review and a survey on tidal wetland restoration sites showed that soil moisture controlled by site elevation and microtopography is a relevant factor for plant species distribution in tidal wetlands: Elevation controls wetland plant distribution, whereas initial establishment success is important for restoration, and the design of the restoration site relief affects the success or failure of plantings [7].
The genus Salix comprises about 500 species worldwide with deciduous trees and shrubs that form communities which colonize bare ground along watercourses: Salix humboldtiana Willdenow is a large tree species which grows along water courses in South America; Salix nigra Marshall trees form extended floodplain forests in eastern North America and is often used for bank stabilization; Salix alba L. trees form extended floodplain forests in Eurasian riverbank communities [8] and the foundation of the tidal freshwater forested wetlands (TFFW) of estuarine systems in Europe [6]. Field studies showed the limitation of S. alba occurrence in tidal freshwater wetlands under oligohaline conditions along the Elbe estuary and the performance of vegetative propagules in a hydroponic experiment [5]. Flood control infrastructure, urbanisation and agriculture led to large losses of TFFWs in Europe, where the remaining TFFWs occur along the Elbe, Rhine-Meuse, and Scheldt estuaries. In these Salix alba-dominated TFFWs, S. cinerea, S. caprea, S. triandra, S. fragilis, S. dasyclados, and S. viminalis are the main cooccurring shrub species [6], but TFFWs in Europe up to the river mouth at the North Sea are naturally composed of Salix alba, S. rubens, S. fragilis, S. triandra, S. viminalis, and additionally S. purpurea at sandy locations [9].
Willows are woody species with characteristics that have benefited societies and the environment for millennia: wood and non-wood products (e.g., basketry due to flexible twigs), rehabilitation of degraded land, bioenergy production, and mitigation of climate change [8]. Plantations as windbreaks and shelterbelts were implemented in large-scale programs, e.g., in the North American Prairie Province’s shelterbelt program and the Chinese Three North Shelterbelt program, with more than 20 million ha of Salicaceae (Poplars and Willows) plantations [10]. Floodplain willows are largely adapted to hydrological disturbance: White willow (Salix alba L.) trees even attenuated waves up to a 2.5 m wave height in a real scale experiment in the Delta flume, NL, suggesting that these floodplain forests may play a significant role in flood control [11]. Juvenile S. alba and S. viminalis (Basket willow) reduced the current velocity both in summer and leafless during winter in a flume study, indicating that floodplain Salix species with flexible twigs may be suitable for use in foreshore flood protection along estuaries where storm surges affect floodplains during winter [12]. Recently, the protective force of ecological floodplain forests to promote flow velocity reduction and sediment deposition along lower yellow river embankments was confirmed depending on forest density, biomechanical properties and stand width of trees [13]. Thus, floodplain forest restoration can be a useful Nature-Based Solution to create climate-resilient communities in lowland estuaries [14].
Large tidal freshwater wetlands are restricted to lowland estuaries (e.g., Chesapeake Bay (USA), Dutch Delta (NL), Elbe (GER), Scheldt (B, NL), Thames (UK)) in former river valleys [15], large river mouths in microtidal environments (e.g., Mississippi), or “tidal river estuaries” with high discharge and low salt water intrusion (e.g., Rio de la Plata). Maintaining natural structures and functions and restoring degraded habitats with respect to both ecological and socio-economic needs is challenging [16,17,18] since estuaries are linked to major population centres and particularly vulnerable to anthropogenic induced hazards [19,20] and hazards due to both extreme events and climate change [21]. More than a dozen types of natural up to anthropogenic hazards to the estuarine environment are detailed [22], including concerns regarding measures to protect the coastline against these hazards, which may result in a degraded ecosystem contravening nature conservation law. Jennerjahn and Mitchell [21] highlight in their syntheses on “Pressures, stresses, shocks and trends in estuarine ecosystems” the necessity to manage estuarine ecosystem restoration for both the ecosystem and the stakeholders. Solutions to protect and create valuable wetland habitats for both the environment and flood control, e.g., through measures such as vegetation restoration to form sediment traps and enhance accretion, are suggested [23]. The recognition of tidal freshwater wetland values has increased, and environmental regulations today require and drive the restoration to mitigate losses of tidal freshwater wetlands worldwide [24].
In Europe, legislation on estuaries includes the Floods Directive [25] as a framework to reduce negative consequences of flooding on the human population and the European Habitats Directive (HD) [26] and Wild Birds Directive (BD) [27], which aim to protect biodiversity on both the species and habitats level. Most of the European estuaries are designated as Natura 2000 sites according to the HD [26], a legally binding system of protected areas in EU member states. Within Natura 2000 sites for both habitat types and species, the conservation and restoration of a good conservation status is mandatory. Estuaries as a whole are protected, whereas an estuary may include other habitats, such as tidal freshwater forested wetlands (TFFW), and may represent habitats for endemic species [28]. To improve the conservation status of species and habitats, the Integrated Management Plan for the Elbe estuary [4], which is legally based on the HD [26] and BD [27], was made by the neighboring federal states, the Federal Administration for Waterways and Navigation, and the Hamburg Port Authority in participation with local stakeholders. In the Elbe estuary, TFFW is a target habitat for restoration due to the bad conservation status. TFFW should be restored via succession on bare ground, e.g., on estuarine islands and in dynamic tidal freshwater wetlands but initialization of tidal forests via plantation is indicated at many locations since bare ground is scarce, e.g., due to revetments [28]. Where dispersal pathways of desired species are interrupted, plantings are required to initiate the rapid establishment of desired species and reduce the establishment of non-native species [29]. However, despite policy mandates for restoration, empirical data on the initial establishment success of different Salix species in tidal freshwater wetlands for TFFW restoration are scarce.
Against this background, we investigated the initial establishment success of TFFW in the Elbe estuary. Six Salix species were planted in tidal freshwater wetlands. These plantations were conducted in different habitat types, from stream valley meadows, reed stands, and wet sinks to bare ground, banks of small bays, and tidal creeks, and were investigated in the restoration project. The goal of this study was to answer three targeted questions: (1) the difference in survival rate among different Salix species; (2) the effect of habitat type on growth metrics; (3) the interaction between species identity and habitat conditions.
2. Materials and Methods
2.1. Study Species and Study Site
Six Salix species characteristic for tidal freshwater forested wetland were selected for the initialisation of TFFW restoration. Autochthonous S. fragilis and S. x rubens trees, and S. purpurea, S. triandra, and S. viminalis shrubs were used in accordance with the requirements of conservation measures. Vegetative propagules were collected from Salix individuals from tidal freshwater wetlands at the macrotidal Elbe estuary upstream of the port of Hamburg and cultivated since 2013 in a professional tree nursery (Forest Tree Nursery Schrader; located north-west of Hamburg). This autochthonous plant material was used for initialisation plantings, e.g., in a small-scale pilot project with plantation of 500 rooted Salix rods in a tidal freshwater wetland (53°24′25.00″ N, 10°14′46.10″ E) along the bank above the revetment [28].
Contrary to this former small scale pilot project, the present study is based on a large-scale project where 2680 juvenile Salix trees were planted in a wide tidal freshwater wetland, which is exposed to the tidal dynamic of the Elbe estuary (53°24′06.1″ N, 10°12′12.0″ E). The restoration of the tidal dynamics and the TFFW was part of a compensation measure for the deepening of the Elbe estuary navigation channel, which took place in 2021 and was carried out by the federal state of Hamburg. This compensation measure generally aimed to develop tidal freshwater wetland habitats and specifically the settlement potential for the Elbe water dropwort (Oenanthe conioides [Nolte] (Lange)), a plant species of tidal freshwater wetlands endemic to the Elbe estuary listed as a priority species in the HD, and it aimed to establish tidal freshwater forest in tidal wetlands, listed as priority habitat which has to be restored according to the Habitats Diorective [26].
2.2. Restoration Design
First, the tidal freshwater wetland site was modelled in 2021 and 2022 to prepare the restoration of the tidal dynamic both on an Elbe Island and the mainland in front of the dikeline (Figure 1). Thereinafter, initial plantings were carried out according to a planting plan within the restoration site on 30 subplots on an Elbe Island (1 ha; Figure 1 left hand side) and the mainland in front of the dikeline (2.3 ha; Figure 1 right hand side).
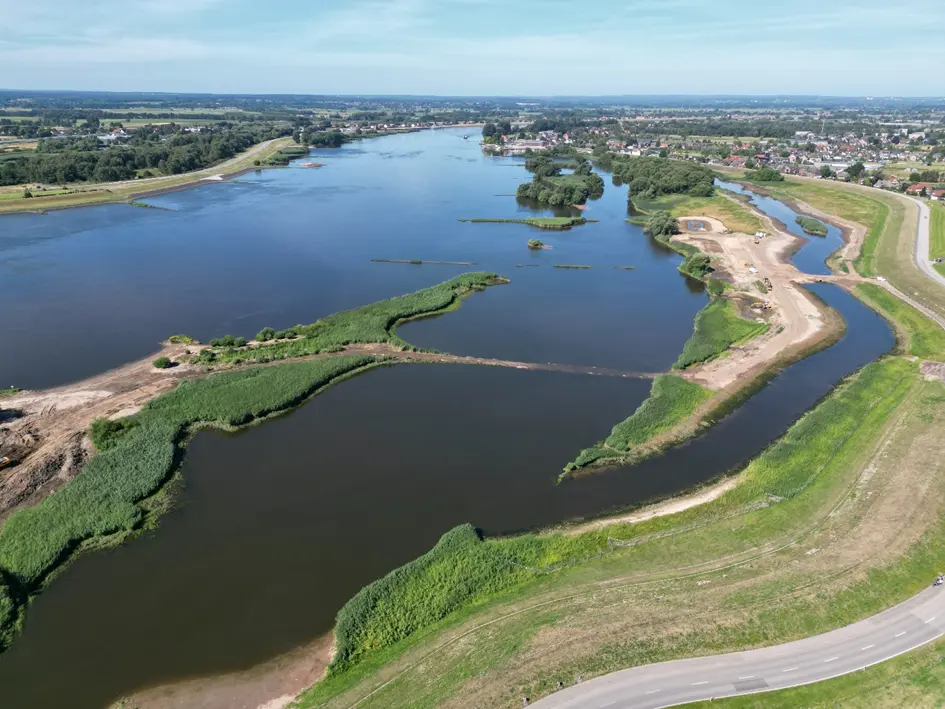
Figure 1. Tidal freshwater wetland in front of the dikeline upstream from port of Hamburg; restoration of tidal dynamics and tidal freshwater wetland forest in 2022 required as compensation measure for deepening of the navigation channel of the Elbe estuary; tidal freshwater wetland on an Elbe Island (left); tidal freshwater wetland on the mainland (right); photo Volker Dinse 2022, Nature Protection Agency; Ministry for Environment, Climate, Energy and Agriculture Hamburg.
In autumn 2022, before the beginning of the storm surge season, 2680 juvenile individuals of six Salix species, at a height of 1.5 m, with a planting distance of 3 m among them, were planted 30 cm deep in the ground. On 30 plots, 1254 S. alba, 381 S. rubens, 215 S. fragilis, 532 S. viminalis, 466 S. purpurea, and 198 S. triandra were planted in the tidal freshwater wetlands along the Elbe estuary.
Contrary to the small-scale study mentioned above in which mowing and removal of competing plants took place [30], no maintenance measures were carried out after the initial planting. The Salix individuals were planted in diverse habitats with different ecological conditions at the restoration site in the tidal freshwater wetlands: a higher elevated stream valley meadow, dense reed stands along water courses, wet sinks and small bays with reduced current velocities, bare ground without competing vegetation, and at tidal creeks with exposition to water currents. The six Salix species were planted in the diverse habitats according to their ecological behaviour and the site conditions. The spatial distribution of 30 subplots was thus arranged in a stratified design where the tidal gradient was considered. Since Salix alba is the key stone species of lowland floodplain forests [9] and forms willow forests in remaining tidal freshwater wetlands [6], the plantation was dominated by this species. Salix alba tolerates twice daily tidal flooding in the field [30] and shows xeromorph features since the leaves are covered densely with silvery hairs, which reflect the sunlight and give the species its name and silvery appearance [9]. Thus, Salix alba was planted in all habitat types and also on the higher elevated stream valley meadow. Since Salix floodplain trees usually occur in groups, these S. alba plantations were accompanied by a lower individuals number of the other treelike species S. fragilis and S. rubens. The shrublike Salix species S. triandra and S. viminalis are characteristic for low-elevated seam-shaped shrubberies along the tidal gradient and reed stands, whereas S. purpurea is even able to tolerate high current speed at water edges on bare ground [9]. Thus, the three shrublike Salix species were planted at low elevations along the tidal gradient along reed stands, wet sinks and small bays with reduced current velocities, but also on bare ground without competing vegetation, whereas S. purpurea was also planted at tidal creeks with exposition to water currents. Individuals of the six Salix species were grouped in clusters. These clusters were distributed in a stratified design among the different habitats at the restoration site (Figure 2).
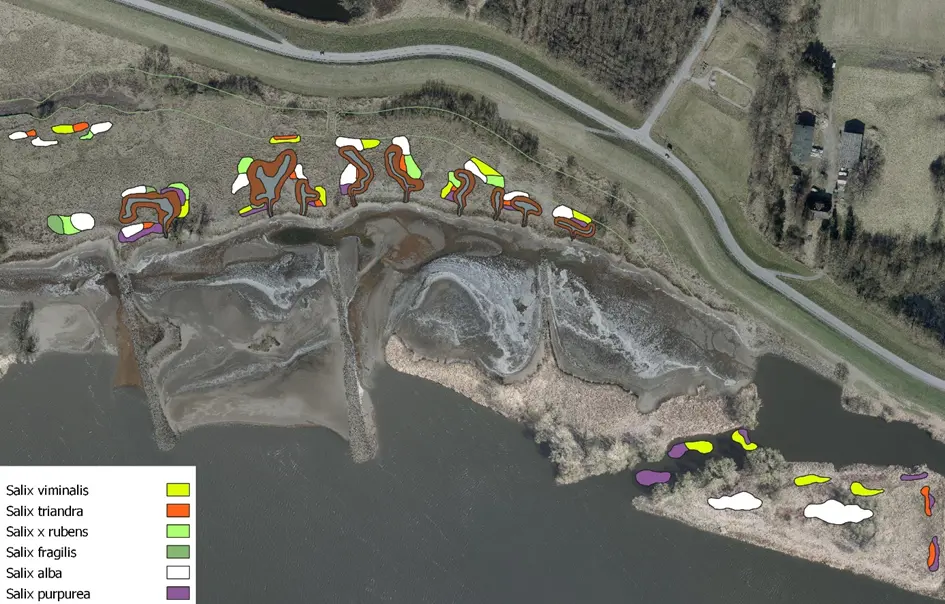
Figure 2. Tidal freshwater floodplain forest plantation map (status before modelling the site for restoration) with the position for the six planted Salix species (S. alba, S. fragilis, S. rubens, S. triandra, S. viminalis, S. purpurea). The restoration site is located in a tidal freshwater wetland in front of the dikeline upstream of Hamburg; restoration of tidal dynamics and tidal freshwater wetland forest in 2022 as a compensation measure for the deepening of the navigation channel of the Elbe estuary.
3. Data Collection and Statistical Analysis
The initial establishment success of the planted Salix individuals within the habitats at the restoration site in the tidal freshwater wetland was investigated in July and August 2022. The trunk height was measured, and the number of stems was recorded. Salix individuals in tidal freshwater wetlands are exposed to diverse disturbances and may be affected by estuarine currents and waves, storm surges, and ice scour, as well as by strong wind and periodic tidal flooding, which may cause root cease. This may induce changed trunk position, vitality of stem, and resprouting shoots. Thus, trunk position was recorded in categories: 1—erect, 2—inclined, 3—prostrate) and used as a response variable to refer to the complexity of the estuarine environment. Furthermore, the stem number was recorded. Browsing by game caused damage on some of the planted Salix individuals, e.g., the branches were eaten of and/or the bark was peeled. The browsing damage was recorded in two categories: browsing: 0—no browsing damage, 1—browsing damage. The damage due to drought was also visible as more or less dried leaves and shoots. The drought damage was recorded in three categories: 0—no drought damage, 1—moderate drought damage, and 2—intense drought damage. The vitality of the stems differed, e.g., due to different leaf numbers and canopy density. The vitality was recorded in four categories: 0—vital, 1—moderate reduced vitality, 2—reduced vitality, 3—dead. Floodplain willows show the capacity to resprout shoots after disturbance like browsing, drought, or other physical disturbance [31]. The resprouting capacity was recorded in three categories: 0—no resprouting shoots, 1—some resprouting shoots, and numerous resprouting shoots. Two-factorial ANOVAs were applied to analyze the effect of Salix species and habitat within the restoration site on height, stem number, trunk position, browsing and drought damage, vitality of the stem, and resprouting shoots. The program Sigma Plot 15.0 was used for statistical analyses and to create graphs. However, the statistical analysis has limitations, as the study is based on a public restoration measure and lacks a scientific experimental design. This indicates that the results are exploratory and should be interpreted with caution.
4. Results
4.1. Initial Establishment Success of Salix Individuals in TFFW Restoration in the European Elbe Estuary
In the study on the initial establishment success of the 2680 Salix individuals, which were planted in autumn 2022 to restore a TFFW at the Elbe estuary upstream of Hamburg, 2192 individuals were detected again in summer 2023. Of these 2192 Salix individuals 159 had died off. Accordingly, 2033 Salix individuals established, which corresponds to 75% of the initially planted individuals. With respect to the species diversity of the planted Salix treelike individuals, the following numbers were recorded: 756 of the initial 1254 S. alba individuals (60.3%), 278 S. rubens of 383 (72.6%), and 81 S. fragilis of 215 (37.7%). With respect to the diversity of the planted Salix shrublike individuals, the following numbers were recorded: 456 S. viminalis of 532 (85.7), 239 S. purpurea of 466 (51.3), and 140 of 198 initially planted S. triandra individuals (70.7) (Table 1).
Table 1. Initial establishment success of diverse Salix species (S. alba, S. rubens, S. fragilis, S. viminalis, S. purpurea. S. triandra) in a tidal freshwater wetland forest restoration project in the Elbe estuary upstream of Hamburg (a) initially planted Salix individuals in autumn 2022; (b) initially established Salix individuals in summer 2023; (c) establishment percentage.
|
Salix Species |
S. alba |
S. rubens |
S. fragilis |
S. viminalis |
S. purpurea |
S. triandra |
|---|---|---|---|---|---|---|
|
(a) Initially planted (no) |
1254 |
383 |
215 |
532 |
466 |
198 |
|
(b) Established (no) |
756 |
278 |
81 |
456 |
239 |
140 |
|
(c) Establishment percentage |
60.3 |
72.6 |
37.7 |
85.7 |
51.3 |
70.7 |
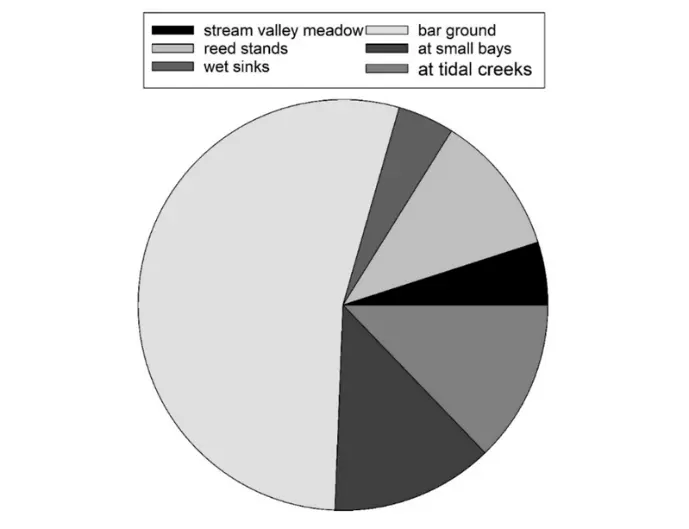
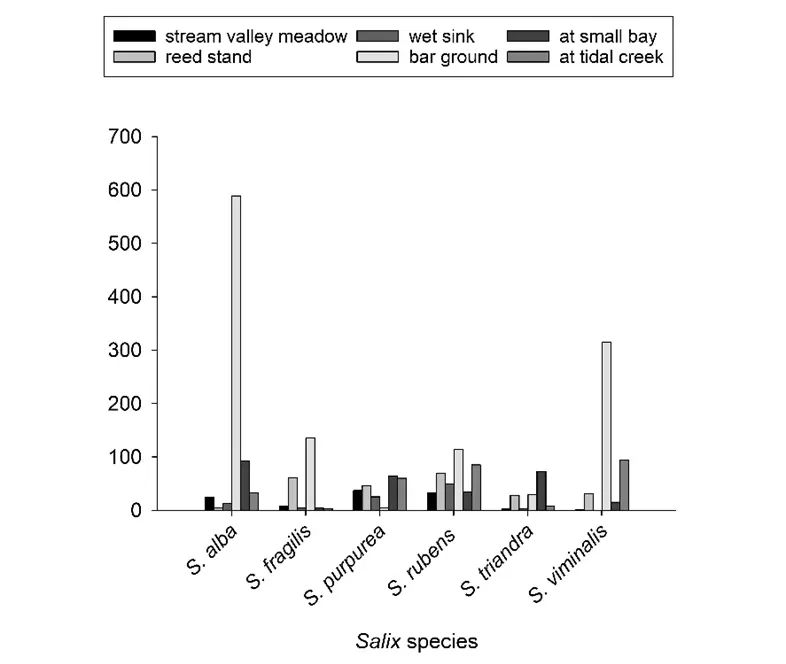
The 2192 Salix individuals that were detected in summer 2023 after plantation in autumn 2022 showed initial establishment success in diverse habitats (stream valley meadow, reed stands, wet sinks, bare ground, at small bays, at tidal creeks within the restoration site). Hundred Salix individuals were recorded in stream valley meadows, 240 individuals were found within reed stands, 95 in wet sinks, most of the Salix individuals (1187) established on bare ground, 282 at small bays, and 283 at tidal creeks (Figure 3a). Within this distribution among the diverse habitats, the majority of S. alba (589), S. fragilis (135), S. rubens (114), and S. viminalis (315) were found on bare ground, whereas S. purpurea (64) and S. triandra were mainly found at small bays within the tidal wetland restoration site (Figure 3b).
 |
 |
|
(a) |
(b) |
Figure 3. Diverse habitats within the tidal freshwater forest restoration site: (a) stream valley meadow, reed stands, wet sinks, bare ground, at small bays, at tidal creeks; (b) Diversity of Salix species (S. alba, S. rubens, S. fragilis, S. viminalis, S. purpurea, S. triandra) within these habitats at the Elbe estuary upstream of port of Hamburg recorded in summer 2023.
4.2. Differences Among Salix Species in Initial Establishment Success in TFFW Restoration
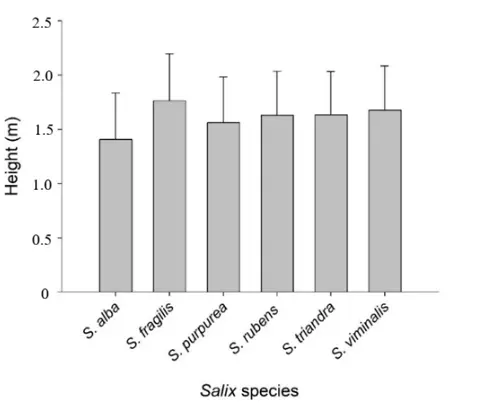
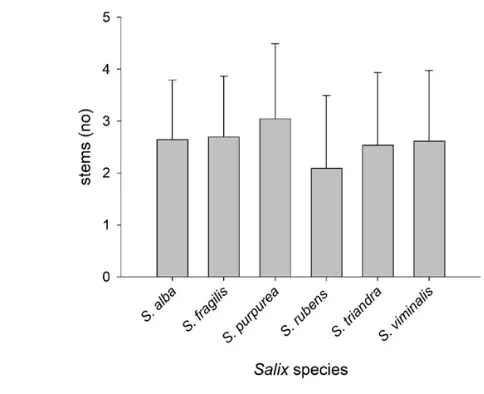
The two-factorial ANOVA showed significant effects of the factor species (F = 37.83; p < 0.001) and site (F = 10.799; p < 0.001) on the height of the diverse planted Salix species at the TFFW restoration site. Salix fragilis was higher compared to S. alba (p < 0.001), S. purpurea (p < 0.001), S. rubens (p < 0.001), and S. triandra (p < 0.01). Salix viminalis was higher compared to S. alba (p < 0.01), S. purpurea, and S. rubens (p < 0.001). Both Salix purpurea and S. triandra were higher compared to S. alba (p < 0.001) (Figure 4a). Regarding the factor habitat, Salix individuals were higher within the reed beds (p < 0.001), at the small bays (p < 0.05), and at the tidal creeks (p < 0.01) compared to those that were planted on bare ground. Moreover, the Salix individuals in the reed beds were higher compared to those at small bays (p < 0.05) and at tidal creeks (p < 0.05). The number of stems differed among the Salix species (F = 2.66; p < 0.001) (Figure 4b). Salix purpurea developed more stems compared to S. alba, S. fragilis, S. rubens, S. triandra, and S. viminalis (p < 0.001).
 |
 |
|
(a) |
(b) |
Figure 4. Effects of Salix species (S. alba, S. rubens, S. fragilis, S. viminalis, S. purpurea. S. triandra) on (a) the height (m) of planted individuals, and (b) the stem number on the initial establishment success in the tidal freshwater forest restoration at the Elbe estuary upstream of Hamburg recorded in summer 2023.
The effect of both species (F = 6.180; p < 0.001) and habitat (F = 32.618, p < 0.001) on the stem vitality of the Salix individuals was significant. Salix rubens showed the highest vitality, the vitality of S. alba, S. purpurea, and S. viminalis was intermediate, and the vitality of S. fragilis and S. triandra was lowest (Figure 5 and Figure 6; Table 2).
The factor species (F = 11.028; p < 0.001) and habitat (F = 8.371; p < 0.001) affected the stem position of the Salix individuals significantly. Multiple comparisons showed that the stem position of Salix viminalis was the least erect, contrary to S. rubens, which showed the most erect stem position. The stem position was more often inclined and prostrate in Salix individuals that established on bare ground compared to those in the stream valley meadows (p < 0.001), in reed stands (p < 0.001), in wet sinks (p < 0.01), and at tidal creeks (p < 0.01) (Figure 5 and Figure 6; Table 2).
The resprouting of shoots was significantly affected by both the factor species (F = 10.384; p < 0.001) and the habitat (F = 6.306; p < 0.001). Salix alba, S. fragilis, and S. viminalis developed more resprouting of shoots compared to S. purpurea, S. rubens, and S. triandra. The individuals that initially established on bare ground, at small bays, and at tidal creeks showed more resprouting shoots compared to those in the stream valley meadow and in reed stands (Figure 5 and Figure 6; Table 2).
The effect of both species (F = 61.721; p < 0.001) and habitat (F = 13.550; p < 0.001) on the browsing damage of the initially established Salix individuals was significant. In particular, S. alba was less affected by browsing compared to S. viminalis and S. triandra (p < 0.001). Salix purpurea was the least by browsing affected Salix species. Individuals that were established on bare ground were more affected by browsing compared to those in stream valley meadows, in reed stands, at small bays, and at tidal creeks (p < 0.001) (Figure 5 and Figure 6; Table 2).
The drought damage varied significantly among Salix species (F = 3.551; p < 0.01) and habitat (F = 105.963; p < 0.001), whereas it was highest in S. alba, S. purpurea, and S. rubens. The drought damage of Salix individuals that were planted in stream valley meadows was significantly higher compared to those in reed stands, at wet sinks, bare ground, at small bay, and at tidal creeks (all p < 0.001) (Figure 5 and Figure 6; Table 2).
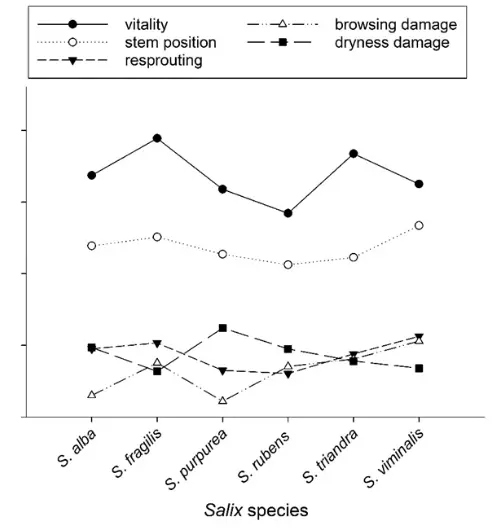
Figure 5. Effects of Salix species (S. alba, S. rubens, S. fragilis, S. viminalis, S. purpurea. S. triandra) on growth parameters recorded in categories (vitality of stem: 0—vital, 1—moderate reduced vitality, 2—reduced vitality, 3—dead; stem position: 1—erect, 2—inclined, 3—prostrate; resprouting: 0—no resprouting shoots, 1—some resprouting shoots, numerous resprouting shoots; browsing damage: 0—no browsing damage, 1—browsing damage; drought damage: 0—no drought damage, 1—moderate drought damage, 2—intense drought damage) on the initial establishment success in a tidal freshwater wetland forest restoration at the Elbe estuary upstream of Hamburg recorded in summer 2023, plantation in autumn 2022.
Table 2. Results of growth parameters of Salix species (S. alba, S. rubens, S. fragilis, S. viminalis, S. purpurea. S. triandra) recorded in categories (vitality of stem: 0—vital, 1—moderate reduced vitality, 2—reduced vitality, 3—dead; stem position: 1—erect, 2—inclined, 3—prostrate; resprouting: 0—no resprouting shoots, 1—some resprouting shoots, 2—numerous resprouting shoots; browsing damage: 0—no browsing damage, 1—browsing damage; drought damage: 0—no drought damage, 1—moderate drought damage, 2—intense drought damage) in the initial establishment success of a tidal freshwater wetland forest restoration at the Elbe estuary upstream of Hamburg recorded in summer 2023 after plantation in autumn 2022 (mean; ±SD).
|
Vitality of Stem |
Stem Position |
Resprouting |
Browsing Damage |
Drought Damage |
||||||
|---|---|---|---|---|---|---|---|---|---|---|
|
S. alba |
1.69 |
1.37 |
1.19 |
0.53 |
0.48 |
0.50 |
0.15 |
0.36 |
0.48 |
0.60 |
|
S. fragilis |
1.94 |
1.35 |
1.26 |
0.51 |
0.52 |
0.50 |
0.38 |
0.40 |
0.32 |
0.59 |
|
S. purpurea |
1.59 |
1.35 |
1.14 |
0.51 |
0.32 |
0.50 |
0.11 |
0.39 |
0.62 |
0.63 |
|
S. rubens |
1.42 |
1.32 |
1.06 |
0.46 |
0.30 |
0.49 |
0.35 |
0.42 |
0.47 |
0.65 |
|
S. triandra |
1.84 |
1.33 |
1.11 |
0.46 |
0.44 |
0.49 |
0.40 |
0.43 |
0.39 |
0.64 |
|
S. viminalis |
1.63 |
1.30 |
1.34 |
0.48 |
0.56 |
0.50 |
0.53 |
0.46 |
0.34 |
0.62 |
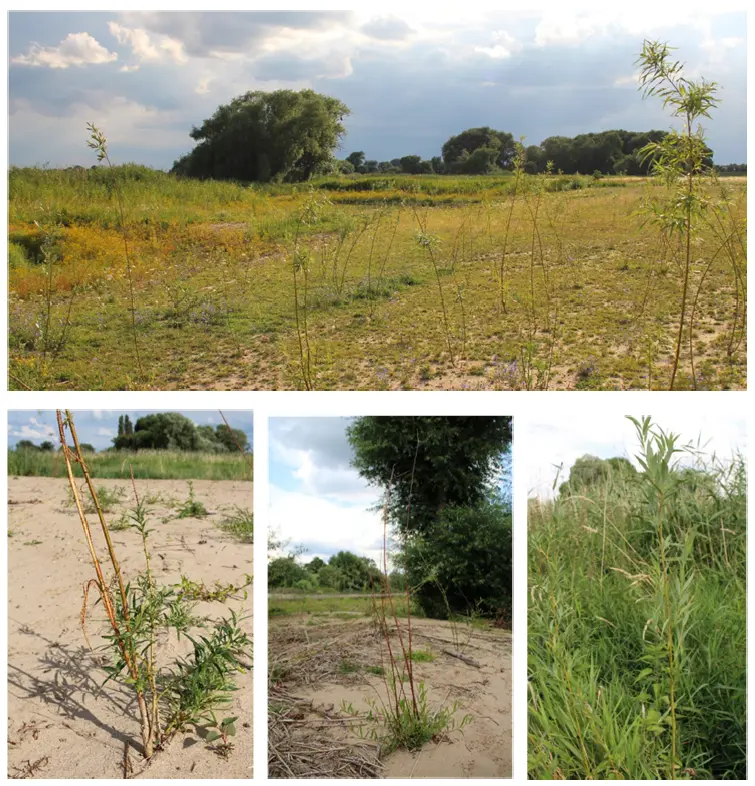
Figure 6. Salix species initial establishment success in tidal freshwater wetland forest restoration at the European Elbe estuary—see White-tailed eagle (Haliaeetus albicilla L.) in mature Salix spec. in the back of the restoration site (on top); Browsing damage and resprouting shoots of S. viminalis (left); Drought damage and resprouting shoots of S. alba planted on bare ground (center); vital S. rubens established with an erect stem in a reed stand (right); recorded in summer 2023, plantation in autumn 2022; photos Matthias Michalczyk.
5. Discussion
5.1. Initial Establishment Success of Salix Individuals in TFFW Restoration in the European Elbe Estuary
In the tidal freshwater wetlands at the Elbe estuary upstream of Hamburg, a restoration of tidal freshwater forest was initiated in 2022. The study on the initial establishment success of six willow species (genus Salix) showed that 75% of the initially planted Salix individuals established successfully. Plantings may be generally necessary to rapidly establish desired species and reduce the establishment of non-native species where dispersal pathways of desired species are interrupted [24]. Similarly, alternative strategies of floodplain forest restoration sites with restoration via succession were dominated by the invasive Canarygras (Phalaris arundinacea), whereas tree planting sites had developed closed tree canopies consisting of the desired tree species. This floodplain forest restoration by tree plantings included the tree species Acer saccharinum, Betula nigra, Fraxinus pennsylvanica, Plantanus occidentalis, Populus deltoides, Quercus bicolor, and Quercus palustris. The restoration was implemented in the Rock River floodplain in Illinois, USA, which was flooded on average four times per year at an average maximum depth of 2.0 m, and the tree plantation was regarded as an efficient restoration method 15 years thereafter [32]. European lowland floodplain forests above the mean high-water level are characterized by Fraxinus excelsior, Ulmus glabra, Ulmus laevis, Quercus robur, but at low lying sites, Populus alba and Populus nigra [9,26], and thus consist of some of the same genera (e.g., Fraxinus, Populus, Quercus) as the floodplain forests in the USA. However, the only genus characteristic for European lowland tidal freshwater wetland forest sites below mean high-water level and more frequent flooding is the genus Salix with a high species diversity within the genus [6,9], similar to that in tidal freshwater forested wetlands in the Scheldt (B), the Dutch Delta, and the Elbe estuary [6,28]. Since Salix dominated floodplain forest is the final stage of succession at sites below the mean high-water level, this study demonstrates promising short-term establishment success of the planted Salix species. However, the long-term development of a structurally and functionally restored forest ecosystem remains to be studied, since the restoration of tidal forests is one goal of a compensation measure for the deepening of the navigation channel of the Elbe estuary, which generally aims to restore tidal dynamics and tidal freshwater wetland habitats.
Within the 75% initially established individuals, the biodiversity of the planted Salix species (S. alba, S. rubens, S. fragilis, S. viminalis, S. purpurea, S. triandra) in the diverse habitats (stream valley meadow, reed stands, wet sinks, bare ground, in small bays, at tidal creeks) where they have been planted at the restoration site has been preserved. This corresponds to Diefenderfer et al. [7], who highlight that the restoration site’s topographic heterogeneity affects plant diversity in tidal wetland restoration projects, where soil moisture was controlled by site elevation, and this microtopography controlled wetland plant distribution. Since plants initial establishment success is important for restoration, the design of the restoration site microtopography affects the success or failure of plantings [8]. In Europe, tidal freshwater wetland vegetation zonation depends on flooding frequency, with Phragmites australis, Bolboschoenus maritimus, Schoenoplectus spp., and Salix spp. as the most frequent species. Above the reed stands, TFFWs are established as the final stage of succession in Salix-dominated systems at higher elevations above the mean high-water level, with the typically co-occurring herbs Caltha palustris, Epilobium hirsutum, Impatiens glandulifera, and Urtica dioica [6]. To the contrary, TFFWs in eastern North America differ largely in species composition depending on geographic and microtopography [7]. Moreover, Salix alba and S. viminalis developed juvenile plants from vegetative propagules up to a half meter of twice daily flooding in a tidal flooding experiment [28] and mature S. alba trees were found up to a half meter below mean high-water level in in tidal freshwater wetlands of the Elbe estuary [30] which may explain their initial establishment success in all habitats at the restoration site in this study. The maintained Salix species composition at the restoration site, as listed in the literature [6,9], can be regarded as a milestone for restoration. Species composition is an important evaluation criterion for vegetation in restored tidal freshwater wetlands, and the species list of reference sites should be similar to that at the restoration site, but differences in species abundance should be accepted [28].
5.2. Differences Among Salix Species in Initial Establishment Success in TFFW Restoration
In our study, S. purpurea shrubs were most reduced in individual number one year after plantation. The nearly 50% reduction in individual number of S. purpurea may have been due to the fact that this light demanding species can be forced out due to shading, as microclimate, along with microtopography, creates the distribution of forest communities [33], and the species was also planted in reed stands in the studied restoration project. The loss of S. purpurea individuals may also be due to the species life history characteristic: preferences of highly disturbed sand and gravel banks close to the water edge [9] which were less present at the restoration site since one the one hand the banks of the tidal creeks may have been too steep and on the other hand the banks of the small bays may have been too little disturbed by water currents. Floodplain Salix species generally show a high adaptability to disturbed river floodplains in the temperate climate and establish predominantly in exposed and disturbed riverine sediments due to fast growth and high regeneration ability [31], but this is particularly true for S. purpurea, which even settles at gravel banks of mountain streams [9].
One reason for the overall loss of 25% of the Salix individuals one year after plantation could be the dry weather conditions in May 2023. According to the German Weather Service [34], May 2023 had an above-average temperature level, more hours with sunshine (255 h instead of 213 h), and less precipitation (23 L/m2 instead of 58 L/m2) in Hamburg. This may also explain in part the reduced stem vitality and the drought damage. The mean number of dead stems (0.93) compared to vital stems (1.65) was high, and 670 of 2033 individuals showed drought damage. The reduced stem vitality and the drought damage may have been enhanced due to the fact that most of the individuals were planted on bare ground in this sandy and sun exposed habitat. The drought damage was highest for S. purpurea but intermediate for S. alba. Although S. alba is the keystone species in Eurasian riverbank communities, it can also survive in drier soils due to its xeromorphic features, whereas S. purpurea is confined to moist sand, river banks, and damp meadows [9], thus, the dry May in 2023 after plantation in 2022 may have affected predominantly S. purpurea.
The floodplain Salix species have life characteristics, such as high regeneration capacity and fast growth [31], that vary widely among Salix species and genotypes [9]. More than half of the individuals in our study showed resprouting shoots, which corresponds to resprouting as a response to drought damage. Ellenberg and Leuschner [9] highlight the high regeneration capacity of floodplain Salix species, with responses to disturbance by increased resprouting shoots. Although the drought damage was highest for S. purpurea and intermediate for S. alba, solely S. alba but not S. purpurea showed high resprouting capacity, which may explain in part the highest individual loss in S. purpurea compared to all other studied Salix species at the restoration site.
To the contrary, S. purpurea showed the least browsing damage in our study. This species is extremely bitter tasting, which may limit the feeding damage from insects and browsing damage from mammals [8]. A similar low browsing damage on S. alba was found in our study. The bark of some Salix species is rich in bioactive phenolic compounds and salicylates known for pharmaceutical use, whereas the accumulation of secondary plant metabolites can be influenced by environmental factors: Drought stress on S. purpurea reduced shoot biomass but led to an increase in bark phenolic compounds [35], which may explain the low browsing damage in S. purpurea compared to most other Salix species in our study. Contrary to S. alba and S. purpurea, S. viminalis was heavily affected by browsing—this Salix species showed the by far highest browsing damage. Salix viminalis is not known for herbivory defense due to high contents of secondary compounds compared to those in S. alba and S. purpurea [35]. Deer species prefer naturally occurring Salix species and use them for browsing during all seasons. However, the fast-growing S. viminalis, which is often used for bioenergy production, e.g., in southern Sweden, can be particularly affected by herbivory by roe deer (Capreolus capreolus), which can cause serious damage to both naturally occurring and individuals in short rotation coppices [36]. Salix was selected for bioenergy production because of high production to testen potential, high resprouting capacity after harvest, limited pest problems, and short production cycle [37]. Members of the Salicaceae are recognized as woody plants for short rotation forestry, but S. viminalis has been the species of choice for coppice cultures due to extremely fast growth and excellent resprouting capacity, and was introduced from Eurasia to North- and South-America where it has been used for basketry, stream bank protection, and as a bioenergy crop [8]. This suggests, S. viminalis was most affected by browsing due to lower phytochemical defense, but regenerated fast by developing new shoots, whereas S. alba was less affected by herbivory due to phytochemical defense but was largely affected by drought and responded with numerous fast resprouting shoots.
6. Conclusions
More than 75% of the Salix individuals initially established, the diversity among Salix species characteristic of TFFW was maintained, and Salix individuals of all planted species established in diverse habitats at the restoration site one year after an initial plantation at the European Elbe estuary upstream from Hamburg. This suggests that the planting of Salix individuals may be an appropriate measure to initiate the restoration of tidal freshwater forests in European lowland estuaries where tidal dynamics are lacking. Plantings may promote the rapid establishment of desired species and reduce the establishment of non-native species where dispersal pathways of desired species are interrupted, and the window of opportunity for TFFW restoration via succession is not given. However, the one-year monitoring period demonstrates initial establishment success, but it is not sufficient to conclude long-term restoration success. Conclusions about the full functional recovery of tidal freshwater forest and restoration require long-term studies on the Salix species, including the resprouting capacity after drought damage and browsing damage. Restoration via succession can also be an option for TFFW restoration for natural colonization on bare ground that can easily be reached by dispersal of native species at sites with tidal dynamics and high moisture, but this has to be tested. In the present study, however, initial plantings led to the rapid initial establishment success of the desired Salix species, which are characteristic for TFFW and protected as habitat type by the HD [26], and may contribute to facilitate climate resilient communities in lowland estuaries due to flood protective values [18]. This has important management implications and can serve as a model for the successful initial establishment of Salix species for the restoration of TFFW at European estuarine upstream sites and elsewhere.
Acknowledgments
Thanks to the German Nature Conservation Authority (BUKEA Hamburg) for the permission to use the data, report, and aerial image of the restoration project to produce this manuscript which is intended to enhance science-based TFFW restoration. Thanks to Christian Michalczyk and Matthias Michalczyk for assistance in the field and photos.
Ethics Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The data are accessible on demand from the author.
Funding
This research received no external funding.
Declaration of Competing Interest
The author declares that she has no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
References
- Duarte CM, Losada IJ, Hendriks I, Mazarrasa I, Marbà N. The role of coastal plant communities for climate change mitigation and adaptation. Nat. Clim. Change 2013, 3, 961–968. DOI:10.1038/nclimate1970 [Google Scholar]
- García-Alonso J, Lercari D, Defeo O. Río de la Plata: A Neotropical Estuarine System. In Coasts and Estuaries; Wolanski E, Elliott M, Ramachandran R, Eds.; Elsevier: Burlington, UK, 2019; pp. 45–56. [Google Scholar]
- Elliott M, Day JW, Ramachandran R, Wolanski E. A synthesis: What is the future for coasts, estuaries, deltas and other transitional habitats in 2050 and beyond? In Coasts and Estuaries; Wolanski E, Elliott M, Ramachandran R, Eds.; Elsevier: Burlington, UK, 2019; pp. 1–28. [Google Scholar]
- Integrated Management Plan for the Elbe Estuary. 2012. Available online: http://www.natura2000-unterelbe.de/links-Gesamtplan.php (accessed on 27 September 2024).
- Markus-Michalczyk H, Hanelt D, Ludewig K, Müller D, Schröter B, Jensen K. Salt intrusion in tidal wetlands: European willow species tolerate oligohaline conditions. Estuar. Coast. Shelf Sci. 2024, 136, 35–42. DOI:10.1016/j.ecss.2013.11.008 [Google Scholar]
- Struyf E, Jacobs S, Meire P, Jensen K, Barendregt A, Studies PC, et al. Plant communities of European tidal freshwater wetlands. In Tidal Freshwater Wetlands; Barendregt A, Whigham DF, Baldwin AH, Eds.; Backhuys Publishers: Leiden, The Netherlands, 2009; pp. 59–70. [Google Scholar]
- Diefenderfer HL, Sinks IA, Zimmerman SA, Cullinan VI, Borde AB. Designing topographic heterogeneity for tidal wetland restoration. Ecol. Eng. 2018, 123, 212–225. DOI:10.1016/j.ecoleng.2018.07.027 [Google Scholar]
- Dickman DI, Kuzovkina YA. Poplars and Willows of the World. With Emphasis on Silvicultural Important Species. In Poplars and Willows: Trees for Society and the Environment; Isebrands JG, Richardson J, Eds.; CAB International and FAO Food and Agriculture Organisation of the United Nations (FAO): Rome, Italy, 2014; pp. 8–91. [Google Scholar]
- Ellenberg H, Leuschner C. Vegetation Mitteleuropas mit den Alpen, 6th ed.; Ulmer: Stuttgart, Germany, 2010. [Google Scholar]
- Carle J, Ma Q. Challenges of translating science into practice: Poplars and other species in the Three North Region of China. Unasylva 2005, 56, 31–37. Available online: https://www.fao.org/4/a0026e/a0026e09.pdf (accessed on 20 June 2026).
- van Wesenbeeck BK, Wolters G, Antolínez JA, Kalloe SA, Hofland B, de Boer WP, et al. Wave attenuation through forests under extreme conditions. Sci. Rep. 2022, 12, 1884. DOI:10.1038/s41598-022-05753-3 [Google Scholar]
- Markus-Michalczyk H, de Smit J, Zhu Z, Mchedlishvili A, van Bree J, Bouma TJ. Seasonality and spacing determine the effect of juvenile floodplain willows (Salix alba and Salix viminalis) on water current velocities. Estuar. Coast. Shelf Sci. 2020, 238, 106697. DOI:10.1016/j.ecss.2020.106697 [Google Scholar]
- Wu X, Zhang X, Zhang X, Xu Z. Assessing Ecological Protective Forests for Reducing Flow Velocity and Promoting Sediment Deposition Along Lower Yellow River Embankments. Water 2026, 18, 1498. DOI:10.3390/w18121498 [Google Scholar]
- Markus-Michalczyk H, Michalczyk M. Floodplain Forest Restoration as a Nature-Based Solution to Create Climate-Resilient Communities in European Lowland Estuaries. Water 2023, 15, 440. DOI:10.3390/w15030440 [Google Scholar]
- Baldwin AH, Barendregt A, Whigham DF. Tidal freshwater wetlands, an introduction to the ecosystem. In Tidal Freshwater Wetlands; Barendregt A, Whigham DF, Baldwin AH, Eds.; Backhuys Publishers: Leiden, The Netherlands, 2009; pp. 1–10. [Google Scholar]
- Boerema A, Meire P. Management for estuarine ecosystem services: A review. Ecol. Eng. 2016, 98, 172–182. DOI:10.1016/j.ecoleng.2016.10.051 [Google Scholar]
- Bouma TJ, Temmerman S, van Duren LA, Martini E, Vandenbruwaene W, Callaghan DP, et al. Organism traits determine the strength of scale-dependent bio-geomorphic feedbacks: A flume study on three intertidal plant species. Geomorphology 2013, 180–181, 57–65. DOI:10.1016/j.geomorph.2012.09.005 [Google Scholar]
- Elliott M, Mander L, Mazik K, Simenstad C, Valesini F, Whitfield A, et al. Ecoengineering with Ecohydrology: Successes and failures in estuarine restoration. Estuar. Coast. Shelf Sci. 2016, 176, 12–35. DOI:10.1016/j.ecss.2016.04.003 [Google Scholar]
- Lotze HK, Lenihan HS, Bourque BJ, Bradbury RH, Cooke RG, Kay MC, et al. Depletion, Degradation, and Recovery Potential of Estuaries and Coastal Seas. Science 2006, 312, 1806–1809. DOI:10.1126/science.1128035 [Google Scholar]
- Barbier EB, Hacker SD, Kennedy C, Koch EW, Stier AC, Silliman BR. The value of estuarine and coastal services. Ecol. Monogr. 2011, 81, 169–193. DOI:10.1890/10-1510.1 [Google Scholar]
- Jennerjahn TC, Mitchell SB. Pressures, stresses, shocks and trends in estuarine ecosystems—An introduction and synthesis. Estuar. Coast. Shelf Sci. 2013, 130, 1–8. DOI:10.1016/j.ecss.2013.07.008 [Google Scholar]
- Elliott M, Cutts ND, Trana A. A typology of marine and estuarine hazards and risks as vectors of change: A review for vulnerable coasts and their management. Ocean. Coast. Manag. 2014, 93, 88–99. DOI:10.1016/j.ocecoaman.2014.03.014 [Google Scholar]
- Temmerman S, Meire P, Bouma TJ, Herman PMJ, Ysebaert T, De Vriend HJ. Ecosystem-based coastal defense in the face of global change. Nature 2013, 504, 79–83. DOI:10.1038/nature12859 [Google Scholar]
- Baldwin AH, Hammerschlag RS, Cahoon DR. Evaluating Restored Tidal Freshwater Wetlands. In Coastal Wetlands, 2nd ed.; Perillo GME, Wolanski E, Cahoon DR, Hopkinson CS, Eds.; Elsevier: Amsterdam, The Netherlands, 2019; pp. 889–912. [Google Scholar]
- Directive 2007/60/EC of the European Parliament and of the Council of 23 October 2007 on the Assessment and Management of Flood Risks. Available online:https://eur-lex.europa.eu/legal-content/DE/TXT/HTML/?uri=CELEX:32007L0060 (accessed on 20 June 2026).
- Council Directive 92/43/EEC of 21 May 1992 on the Conservation of Natural Habitats and of Wild Fauna and Flora. Available online: https://eur-lex.europa.eu/legal-content/DE/TXT/?uri=CELEX:01992L0043-20130701 (accessed on 20 June 2026).
- Directive 2009/147/EC of the European Parliament and of the Council of 30 November 2009 on the Conservation of Wild Birds. Available online: https://eur-lex.europa.eu/legal-content/DE/TXT/?uri=CELEX:32009L0147 (accessed on 20 June 2026).
- Markus-Michalczyk H, Michalczyk C. “Make me a willow cabin at your gate”: Legislation and implementation of tidal forest restoration at estuarine upstream sites. Estuar. Coast. Shelf Sci. 2018, 210, 1–6. DOI:10.1016/j.ecss.2018.06.004 [Google Scholar]
- Michalczyk C, Koch N, Markus-Michalczyk H. Die Strategie zur Verbesserung des Erhaltungszustands von Lebensraumtypen der FFH-Richtlinie in Hamburg. Nat. Und Landsch. 2016, 91, 553–563. DOI:10.17433/12.2016.50153425.553-563 [Google Scholar]
- Markus-Michalczyk H, Hanelt D. Willow species vary in elevational occurrence and morphological characteristics on the tidal freshwater section of the Elbe estuary. Ecohydrol. Hydrobiol. 2016, 19, 14–23. DOI:10.1016/j.ecohyd.2018.08.006 [Google Scholar]
- Karrenberg S, Edwards PJ, Kollmann J. The life history of Salicacaceae living in the active zone of floodplains. Freshw. Biol. 2002, 47, 733–748. DOI:10.1046/j.1365-2427.2002.00894.x [Google Scholar]
- Matthews JW, McIntyre S, Peralta AL, Rodgers C. Long-Term Assessment of Alternative Strategies for the Restoration of Floodplain Forest in the Presence of an Invasive Grass, Phalaris arundinacea. Wetlands 2020, 40, 655–665. DOI:10.1007/s13157-019-01204-4 [Google Scholar]
- Kevey B. Floodplain Forests. In The Drava River; Lóczy D, Ed.; Springer: Cham, Switzerland, 2019. DOI:10.1007/978-3-319-92816-6_18 [Google Scholar]
- DWD. Available online: https://www.dwd.de/DE/presse/pressemitteilungen/DE/2023/20230530_deutschlandwetter_mai2023_news.html (accessed on 20 June 206).
- Köhler A, Förster N, Zander M, Ulrichs C. Compound-specific responses of phenolic metabolites in the bark of drought-stressed Salix daphnoides and Salix purpurea. Plant Physiol. Biochem. 2020, 155, 311–320. DOI:10.1016/j.plaphy.2020.07.004 [Google Scholar]
- Moritz KK, Parachnowitsch AL, Julkunen-Tiitto R, Björkman C, Ayres MP, Stenberg JA. Roe deer prefer mixed-sex willow stands over monosexual stands but do not discriminate between male and female plants. Environ. Exp. Bot. 2018, 146, 62–67. DOI:10.1016/j.envexpbot.2017.10.015 [Google Scholar]
- Balatinecz J, Mertens P, De Boever L, Yukun H, Jin J, van Acker J. Properties, Processing and Utilization. In Poplars and Willows: Trees for Society and the Environment; Isebrands JG, Richardson J, Eds.; CAB International and FAO Food and Agriculture Organisation of the United Nations (FAO): Rome, Italy, 2014; pp. 527–562. [Google Scholar]